
Table of Contents
Keywords: eucalyptus, water deficit, population growth, wettability, contact angle, spatial distribution, water repellency, biomass.
Abstract
The biological design solutions of the Eucalyptus genus can be mathematically modelled to evaluate their functions. The water management systems of the trees can be modelled by the Penman-Monteith transpiration equation and net deep drainage equation, both of which contribute to the calculations of water potential and analysis of responsive water management. The geometry of the vertical eucalyptus leaves allows for wettability in their arid environments due to nanoscale, hierarchical wax structures which can be topologically modelled. The ability of water droplets to form on the leaves' surface is quantified through Gibbs free energy equation and the Cassie-Baxter equation. Additionally, both the biomass allocation and nutrient concentration of the eucalyptus can be modelled using regressive, parameter-dependent equations which help to analyze the purpose of the tree's composition. Finally, the trees' population dynamics and reproduction can be investigated through statistical analysis of seed dispersal and logistic growth models. This essay seeks to describe the biological processes and design solutions of the eucalyptus tree through mathematical analysis.
Introduction
The eucalyptus genus, which includes more than 700 species, is one of the most widespread and adaptable types of trees. Native mainly to Australia, though now found in many regions worldwide, eucalyptus trees thrive in a range of environments; from wet tropical forests to dry, nutrient-poor woodlands. Their remarkable adaptability comes from a combination of structural and physiological traits that enable them to conserve water, withstand drought, and efficiently manage energy and growth. Features such as specialized leaf geometries, deep root systems, and wax-coated surfaces reflect evolved strategies for survival under challenging environmental conditions.
Mathematical modeling provides a way to describe and analyze these survival strategies in quantitative terms. By examining factors like leaf surface geometry, water transport efficiency, and biomass distribution, researchers can identify the underlying physical and biological principles that are responsible for eucalyptus resilience. Equations that represent processes such as stomatal regulation, water flow, and population dynamics help reveal how these trees maintain stability in different climates. In this way, the eucalyptus serves as a strong example of how mathematical analysis can be used to interpret and predict natural design solutions.
Range of Eucalyptus Species
The eucalyptus species thrive in a wide range of environmental conditions. Some species are more tolerant of arid or dry conditions, while others thrive in moist areas. It is believed that their ability to survive in different conditions is characterized by interspecific differences in the physiological or chemical traits of eucalyptus. The species measured, as shown in Table 1, vary in annual rainfall and growth habit, with the tallest tree, E. oblique, receiving the most annual rainfall, and E. camaldulensis having the largest range in annual rainfall.
Table 1: Eucalyptus species with their respective annual rainfall and growth habit
| Species | E. obliqua | E. rubida | E. camaldulensis | E. polyanthemos | E. tricarpa | E. cladocalyx |
|---|---|---|---|---|---|---|
| Annual Rainfall (mm) | 600-2400 | 550-1400 | 150-1100 | 450-970 | 500-800 | 380-650 |
| Growth Habit | Tall to very tall, 45-90m | Varies from small to tall (35m) | Medium-sized to tall, Up to 45m | Small to medium-sized, 15-25m | Small to medium-sized, 10-25m | Small to tall, 8-35m |
One way to measure this eucalyptus's ability is to observe the changes in osmotic potential in response to water deficits. It has been proposed that the various ways to alter the osmotic potential in the eucalyptus genus account for the differing salt and drought tolerances (Grieve, C. M., & Shannon, M. C., 1999).
Eucalyptus Responses to Water Deficit
All six species were placed in a treatment period and a water deficit period. During the treatment period, the biomass of all species grew differently, within a range of 1.02g - 1.85g of additional biomass. However, during the water deficit period, the relative growth rate of all species decreased by approximately 50%, indicating that all species responded similarly.
As seen in Figure 1, the water deficit greatly impacted the tree’s ability to undergo photosynthesis and controlled the stomatal conductance of the plant. The control group had a maximum rate of photosynthesis ranging from 15 μmol CO2 (1 / m2s) (E. camaldulensis) to 30 μmol CO2 (1 / m2s) (E. polyanthemos), indicating the normal range of values for water treatment. Meanwhile, for the plants with a water deficit, the maximal rate of photosynthesis ranged in value between 5 μmol CO2 (1 / m2s) (E. polyanthemos) and 10 μmol CO2 (1 / m2s) (E. tricarpa) (Merchant, et al., 2008).

Fig. 1. Maximum rates of photosynthesis and stomatal conductance for the well-watered and drought-exposed eucalyptus species (Merchant, et. al., 2008)
The larger trees, which annually receive more millimetres of rainfall, reacted much more to the water drought than the smaller to medium-sized trees, which annually receive smaller quantities of rainfall.
Water uptake by plant roots is an efficient way for plants to adapt to drought conditions. Most trees generally have exponentially decreased fine root biomass as the roots go deeper and usually don’t surpass 1m in depth (Schenk, 2008). However, certain species which need to obtain large quantities of water grow roots to depths of 10 m or larger (Christina, 2016).
The eucalyptus species can be better understood by utilizing certain equations to understand the uptake and flow of water, the soil water balance and the stomatal conductance/resistance. The Penman-Monteith equation, as demonstrated by Equation 1, measures transpiration, which typically decreases when the soil moisture level decreases. During a drought, the stomatal resistance (with subscript a) will increase, overall decreasing our transpiration.
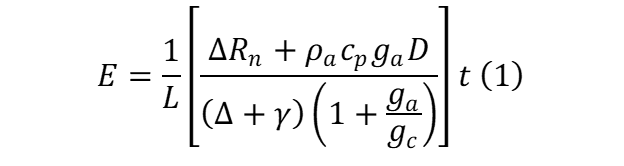
Another equation which measures the water soil content is denoted by Equation 2.

This equation specifically represents the net deep drainage, which is the difference between the deep drainage below the root layer and the upward movement into the same layer (Almeida, 2001). P represents the precipitation, I represent interception, and the outgoing water is denoted by Et, Es, Qnet which represent the transpiration, soil evaporation and net deep drainage, respectively. Using this equation for a plant in a drought setting, evaporation and soil evaporation decrease as the soil water content decreases. The plant’s stomata are not open anymore and the net deep drainage diminishes significantly.

Equation 3 models the relationship between leaf water potential and stomatal conductance. The variable gs represents stomatal conductance, gsmax represents maximum stomatal conductance, Ψ1 is the leaf potential, and Ψ1min represent the minimum leaf potential which can induce stomatal closure. Once again, inducing a drought on a plant, the Epsilon1 variable will increase, resulting in a decrease in overall stomatal conductance. This relationship makes sense because trees close their stomata to stay hydrated during periods of low water availability.
Plants must weather periods of excess rainfall and drought, and through evolutionary adaptation, develop biological methods to preserve their species. The growth of deep roots, which enhances water uptake, especially during periods of drought, allows eucalyptus species to continue thriving in their tropical environment (Almeida, 2001).
Eucalypt Surface Geometry and Wettability
The eucalyptus tree has evolved an intricate mathematical design on its leaf surfaces that enables the species to thrive in extremely arid and drought-prone climates. Beyond its root mechanisms for water storage, the survival of eucalyptus species relies on geometry, and specifically the way their leaves manipulate water through structured surfaces governed by the mathematics of wettability and energy minimization (Ganassoli, 2025). Despite their often-vertical leaf orientation (see Eucalyptus Physics), droplets adhere strongly to eucalyptus leaves, seen in Figure 2, a mechanism especially important when considering the low-water environments the trees inhabit, and their need for water retention for survival.

Fig. 2. Water droplet adhesion to vertical eucalyptus leaves (Billy Heroman’s, 2018).
Leaf Microstructures
In general, the surface of eucalyptus leaves is covered by very fine nanoscale wax structures, as well as microscopic papillae and stomata, producing hierarchical roughness across at least two size scales (Koch, 2008). In a study by Guo and colleagues (2019), the use of scanning electron microscopy (SEM) on three species of eucalyptus, E. woodwardii, E. pachyphylla, and E. dolorosa showed that eucalyptus leaves are covered with hemisphere-like papillae, arranged in quasi-hexagonal patterns, shown on a micrometer scale in Figure 3. Looking deeper, on a nanometer level, the different wax morphologies are unveiled. Needle-like wax particles (5 µm in length, 200 nm in diameter) are present on the surface of E. woodwardia (Figure 3a2), string-like wax coats E. pachyphylla (Figure 3b2), and a flakier wax blankets E. dolorosa (Figure 3c2) (Guo, et al., 2019).

Fig. 3. SEM images of the surface morphologies of three eucalyptus leaves at two different magnifications: (a) woodwardii, (b) Eucalyptus pachyphylla, and (c) Eucalyptus dolorosa (Guo, et al., 2019).
The microstructures, combined with the overlay of nanometer wax forms a hierarchical surface that influences how water droplets would behave on a eucalyptus leaf. The basic geometric parameters of this surface: radius (r0), height (h0), and edge-to-edge spacing (2d0) define the physical topography of each papilla, shown in Figure 4 (Ganassoli, 2025). In the same study as above by Guo (2019), it was found that r0 ranges from 8-10 μm across Eucalypt species, h0 is effectively zero (signifying a flat base), and 2d0 ranges from 9-16 μm. This displays a texture that is smoother and more widely spaced apart than that of the lotus flower, which is often considered when talking about plant hydrophobicity due to the “lotus effect”.

Fig. 4. Generalized physical model of microscopic surface features for (a) eucalyptus leaf; parameters adopted from E. pachyphylla, and (b) lotus leaf (Guo, et al., 2019).
Leaf Wettability
In the eucalyptus, the hemispherical bumps serve a distinct purpose in that they increase the contact area between the leaf and water droplets while still preventing the droplet from spreading too much (Wang, et al., 2015). The curved surfaces let the droplet partially conform to the bumps, increasing the actual liquid-solid area (SLS), and thus the adhesive force per unit length (by increasing said length), given by:

where γLV is the liquid-vapor surface tension, and θ is the contact angle (Lai, et al., 2025). The behaviour of these droplets can be quantified using a contact angle analysis, a core mathematical measure of wettability. The contact angle (θ) is the angle between the tangent of the water droplet and the surface at the point of contact, as can be seen in Figure 5a. A surface with an obtuse angle (>90°) is said to be hydrophobic, and anything over 150° is considered superhydrophobic (the lotus flower for example) (Lai, et al., 2025). The angle reflects the balance between interfacial tensions of the solid, liquid and vapor phases, described by Young’s equation:

where γSV, γSL, γLV represent the solid-vapor, solid-liquid, and liquid-vapor surface energies respectively (Lai, et al., 2025). This Young angle corresponds to a perfectly smooth surface. Deviations from flatness, such as microscopic bumps and pores change the apparent contact angle, allowing rough surfaces to become far more hydrophobic than their chemical composition alone would suggest.
Two classical mathematical models, Wenzel and Cassie-Baxter, extend Young’s law to rough surfaces. A visual comparison of the models can be seen in Figure 5.

Fig. 5. Liquid droplet behavior on the surface for (a) Young’s model, (b) Wenzel’s model, and (c) Cassie-Baxter’s model (Lai, et al., 2015)
The Wenzel model applies when water fully penetrates the microstructure’s surface:

where r is the roughness factor, defined as the ration of actual surface area to its projected (flat) area, and θW and θY are the Wenzel and Young contact angles, respectively (Lai, et al., 2025). The Cassie-Baxter model, by contrast, describes partial wetting, where air pockets remain trapped beneath the droplet, yielding:

where f is the fraction of the solid surface in direct contact with the liquid, and rf is the roughness ratio of that contact fraction (Lai, et al., 2025). Together, these models describe how geometry changes wettability: high degree of roughness (r > 1) and smaller contact fractions (f) amplify hydrophobicity.
In the eucalyptus, the surface is neither purely Wenzel nor Cassie-Baxter, but a composite of the two. On the microscale, droplets partially penetrate the papillae (Wenzel-like), while on the nanoscale, wax and air pockets maintain Cassie-Baxter-like hydrophobicity. This combination produces large apparent contact angles (>140°), while maintaining adhesion; a feature opposite to the lotus, whose superhydrophobic leaves cause water to roll off easily (Guo, et al., 2019).
To probe how much of this behaviour comes from geometry versus chemistry, Guo and colleagues (2019) performed a wax-removal experiment, where eucalyptus leaves were immersed in chloroform to dissolve the wax layer, and contact angles were measured again. The average contact angle dropped about 12°, a relatively minor change given initial angles were near 150°, shown in Figure 6. This demonstrates that although wax enhances wetting robustness, stabilizing the air pockets and reducing surface energy fluctuations, the primary determination of hydrophobicity is geometrical, not chemical.

Fig. 6. Experimental water contact angles of eucalyptus leaves before and after wax removal. While they all decrease after wax removal, they remain very high, indicating hydrophobicity (Guo, et al., 2019).
Energy Implications of Wettability
The wetting state can also be analyzed energetically using Gibbs free energy, which depends on the interfacial areas between phases:

where Sij represents the interface area. The system tends towards configurations that minimize total surface energy, and transitions between wetting states (Cassie to Wenzel) require overcoming an energy barrier (Wang, et al., 2022).
Guo and colleagues (2019) went on to further model the eucalyptus leaf as a plane covered with hemispheres of radius ro, spaced by distance 2d0. When a droplet penetrates the surface gaps to a depth h, it can be expressed as a normalized variable x = h/r0. The roughness and contact area at each penetration depth can be described mathematically as:


These relations were substituted into the Cassie-Baxter and Gibbs free energy equations to compute how the surface energy changes as the droplet sinks into the microstructure. The minimum energy was found to occur at x = 0.75, meaning the water partially fills the wells, but does not fully wet the surface (which matches the observed behaviour of eucalyptus leaves having pinned droplets) (Guo, et al., 2019).
As a droplet sits on the eucalyptus leaf, it can either stay perched on the bumps (composite state) or sink down between them (wetted state). The energy barrier (ΔG₁) between the composite and fully wetted states quantifies the resistance to water infiltration. Modeling revealed that ΔG₁ depends strongly on the edge-to-edge spacing d₀. Smaller d₀ yields higher barriers, increasing hydrophobic stability (Guo, et al., 2019).
A second quantity, the energy potential (ΔG₂), measures the total energy difference between the composite minimum and the wetted minimum. Larger d₀ values increase ΔG₂, meaning that while the wetted state may be energetically favorable, the droplet remains trapped in the composite state because of the barrier ΔG₁ (Guo, et al., 2019). This is metastability, and it ensures that water droplets adhere to the leaves even under disturbance (Wang, et al., 2015).
Comparing eucalyptus to the lotus highlights how geometry dictates function. For lotus leaves, h₀ (cylindrical height) is nonzero, producing much greater ΔG₁ values, but smaller liquid–solid contact areas (Guo, et al., 2019). Eucalyptus leaves, with h₀ ≈ 0 and wider spacing, show a smaller barrier but a much larger contact area. This mathematical difference explains their opposite biological behaviors: the lotus repels water for cleanliness, while the eucalyptus retains it for hydration (Lenz, et al., 2021). The adhesion force given in Equation (1) multiplied by the larger contact area, produces a retention effect, helping the leaf hold droplets even when the leaves are hung vertically. This is a necessary mechanism for maintaining hydration and regulating temperature in dry, windy environments, where rainfall and dew are scarce and evaporate quickly. By holding onto droplets, the eucalyptus leaves extend the availability of water on their surfaces, allowing gradual absorption through stomata and reducing transpiration loss. From a design perspective, this geometry acts as a passive water-retention system; a natural mathematical solution that maximizes water use efficiency without energy expenditure (Wang, et al., 2015).
Modelling Biomass Allocation
The analysis of plant biomass (the organic material in a unit area) and its distribution within an organism illuminates the functional purpose of the tree’s composition. Biomass equations are often used in forestry, environmental management, and pulp/paper manufacturing industries to study and optimize the use of organic tree material (Bonechi et al., 2017). They also aid in the indication of forest carbon stock and the progress of carbon sequestration in forests as carbon sinks (Huang et al., 2025). In 2005, Saint-Andre et al. sought to evaluate hard-to-measure tree characteristics from data like the tree’s diameter at breast height (about 1.37 m; at “breast height” of the observer), the tree’s total height, and tree age. The objective was to construct mathematical models that accurately predicted and analyzed tree biomass.
The target population was a grouping of E. urophylla x E. grandis hybrids in plantations in coastal Congo. Due to the complex, interconnected intricacies of biological components, mathematical models must overcome three main difficulties: heteroscedasticity, genericity, and additivity (Saint-Andre et al., 2004). Heteroscedasticity describes the differing variance in the dependent variable for different independent variable values (e.g. shorter trees have less variance in ratios of small diameter to large diameter roots while taller trees have more variance in root-diameter ratios) (Huang et al., 2025). Genericity describes the ability of the model to be an accurate generalized model, and additivity describes the accuracy of the different subdivision models of biomass (ex. above-ground and below ground) truly totaling to total biomass (Jalal-Kamali et al., 2012). Plots were chosen to have no missing trees (to replicate homogenous growth) and have clean undergrowth without unwanted roots, herbs or shrubs (Saint-Andre et al., 2004). Above-ground biomass calculations used measurements of stem wood, stem bark, leaves, dead branches, and living branches. Below-ground biomass calculations used the measurements of the stump, fine/medium roots, and large roots. The trees were felled and the length and height of the total tree, first living branch, and crown length were measured. The stem was then cut into one-meter sections, and each part of the tree was weighed.
Three equations were made: the first containing all the above-ground measurements for above-ground biomass, the second containing all the below-ground measurements for below-ground biomass, and the last with the sum of all the biomasses (Saint-Andre et al., 2004). For below-ground biomass, the tree’s territory was identified using a Voronoi polygon (allocating each tree a region of soil around it). Roots were collected by digging 7 m down and were then sorted/sieved to be classified as of fine (<5 mm) or medium (between 5 mm and 10 mm). For large root biomass, trees were felled, and roots were excavated and cut 10 cm from the stump before biomass was weighed.
Overall, the biomass calculations could be written as a system of equations of each biomass compartment (biomass subsection, like fine roots) of the forms:


depending on if the relationship between variables was linear or non-linear, respectively. The models were refined to the form:

where the a-intercept represents the baseline biomass, the b slope represents how the compartment biomass increases with tree size, the d slope represents how aging (α) affects the biomass allocation of the compartment, and the c exponent denotes if the biomass scales like tree volume (c=3), surface area (c=2), or some other value. The variance parameter X shows how variability and error increases with tree size (Saint-Andre et al., 2004).
The results of constructing the models yielded visible patterns in the biomass distribution in the eucalyptus hybrid, as seen in Figure 7.

Fig. 7. Modelled relative biomass distribution within Eucalyptus tree stands. Eleven-month-old groupings of trees had 36% biomass represented by leaves and fine roots while the stem only accounted for 19%. Meanwhile, 75-month-old groupings of trees had 62% biomass represented by the stem while leaves and fine roots accounted only for 10%. 7% biomass of bark, 6-9% biomass of large roots, and 1-2% biomass of medium roots stayed consistent independent of age. By compartment equation, below-ground biomass represented 30% of biomass in the young 11-month-old trees but only 16% of biomass in older 135-month-old trees (Saint-Andre et al., 2004).
Function behind Biomass Allocation
The results solidified previous hypotheses about the relationship between tree age and biomass allocation. As the eucalypts grow, their functional priorities shift. Young eucalypts allocate more carbohydrates to branches and leaves to boost photosynthetic productivity and allow for rapid growth (Huang et al., 2025). As the tree’s height increases, the biomass distribution shifts towards the stem to provide mechanical support and devote more resources to hydraulic processes. Trees will also modify their biomass allocations to meet competitive demands, such as crowded crown space or limited water resources (Keeley & Pausas, 2017). Specifically for eucalypts, the initial large allocation to leaves and crown growth aids in epicormic resprouting, or the fire-activation of dormant buds under the bark that allows for recovery of the tree after fire-induced crown damage (Keeley & Pausas, 2017). Additionally, the eucalypt equations also demonstrated elevated bark allocation values compared to other species, harping on the importance of bark as a protective, fire-resistant sheath.
Modeling Nutrient Concentration in Eucalypti
Similarly to the model of biomass distribution, nutrient concentration can be mathematically modelled and used to conclude about varying nutrient roles. Bouvet et al. in 2013 constructed models for nutrient concentration in different biomass compartments in the Eucalyptus hybrid of E. gunnii x E. dalrympleana. They analyzed the distribution of five major nutrients—nitrogen, phosphorus, potassium, calcium, and magnesium—for each of the four main biomass compartments: wood, bark, branches, and leaves; hence 20 models were developed. To find the most accurate equations, five forms were tested for each model:


where the nutrient concentration y is dependent on variations of the baseline nutrient concentration value a, diameter D, age α, and parameters b and c. The results and their corresponding most accurate models are seen in Figure 8.

Fig. 8. Nutrient concentrations in eucalyptus biomass compartments. Each nutrient is assigned one of the above-mentioned models based on lowest error calculated (Bouvet et al., 2013).
Function behind Nutrient Concentration
The levels of nutrients decreased with stand age because of the resulting increase in tree diameter. The first stages of tree growth have nutrient supply coming mainly from the soil due to active and dominant root systems and nutrient-demanding young tissues. But as the vertical growth rate of the eucalypt decreases and the crown closes, the nutrient demand is fulfilled by the recycling of nutrients through biochemical processes (Resquin et al., 2020). Another factor to consider is that as heartwood develops and overtakes immature nutrient-rich stem tissue, the concentrations of resulting cellulose and lignin exceed and dilute the concentrations of previously abundant nutrients like nitrogen and potassium (Resquin et al., 2020).
Mathematical biomass and nutrient concentration models help quantify the dynamic allocation systems with the Eucalyptus. Making biological habits measurable helps highlight how a responsive system optimizes its performance and function to better attune itself for survival.
Population Growth Model and Space Distribution of Eucalyptus
The eucalyptus genus is known for its fast-growing ability and its ecological dominance in hot climate. Introduced all over the world by humans, the genus thrives in diverse environments -from Ethiopia’s arid deserts to California’s mountains. Its superior fitness makes it an invasive tree that threatens the native biodiversity. At the same time, Eucalyptus was found itself to be very valuable in the wood industry, yielding enormous amount of wood for construction and multiple other domains. Consequently, modeling their population growth and spatial distribution is highly relevant in context of sustainable forestry or ecological preservation.
Seed Dispersal
The spatial dynamics of eucalyptus begin at the scale of a single tree. Each tree releases\thousands of seeds following a leptokurtic dispersal pattern (Calviño-Cancela, 2013). In this distribution, most seeds fall near the parental tree, shown in Figure 9. In fact, leptokurtic distributions are distribution that have a strong degree of peaked distribution. Lower degree of distribution is called normal distribution of platykurtic distribution (AnalystPrep, 2019).

Fig. 9. Different kurtosis distribution patterns; Leptokurtic, Normal and Platykurtic (AnalystPrep, 2019)
This means that most of the seeds fall within a few meters of the tree, while a small proportion is carried by wind or other outer forces. Approximately 84% of the seeds fall in the first 5 m of the tree, 98.6% within 15 m and 99.7% in the first 25 m, seen in Figure 10. (Calviño-Cancela, 2013).

Fig. 10. Proportions of fallen seeds for each slice of 5 meters for E. globulus (Calviño-Cancela, 2013)
Data shows a strong leptokurtic pattern with some seeds even reaching a distribution distance of 40m from the tree.
While the ground near the tree is concentrated in seeds, very few will actually survive. Clustering causes high seed density area, but this also causes intense competition for resources. Hence, seeds that fall close to the parent tree have a lower seedling and sapling survival rate than seeds far from the tree (Calviño-Cancela, 2013; Booth, 2017). Spatial distribution of seeds establishes the initial ground of population dynamics. From thereon, each seed will become an individual that will compete against other for resources and space.
Population Growth over Time
Mathematical modeling is very useful in understanding population dynamics. Indeed, population growth can be illustrated in multiple different mathematical models.
The first apparent mathematical model in ecological literature is the exponential growth. This model expresses the change in a population as a derivative of the number of individuals with respect to time and equates it to the growth rate times the number of individuals in the population. The solution to the differential equation is an exponential function (Boelkins et al., 2017; Vandermeer, 2010).

Where

and where C is a constant.
However, the exponential model is highly simplistic as it assumes unlimited resources and no competition, which is unrealistic for natural ecosystems. Resources availability and population density limits the number of individuals in a population. This key concept in ecology is called carrying capacity. The carrying capacity of a species is the number of individuals a given environment can sustain (OpenStax, 2018). Different factors like climate, resource availability and competition define the carrying capacity of a species.
The carrying capacity of eucalyptus is often reached early after the introduction of the tree to a new environment (Skolmen & Ledig, n.d.). Furthermore, E. grandis or E. urophylla are estimated to start self-thinning, a process of reduction of population, at densities around 2000 stems per hectare (William, 2017). This can help to estimate the carrying capacity of eucalyptus. However, no definitive numbers are displayed in the literature.
The logistic growth model incorporates the idea of carrying capacity in its equation. This model extends the previous differential equation by adding a term regulating population growth in function of the carrying capacity (Boelkins et al., 2017; Vandermeer, 2010).

Where the solution to the initial value problem is:

and is displayed in Figure 11.

Fig. 11. The population size in according to the function of time, from the logistic model (Khan Academy, 2016).
It is possible to see that as the number of individuals reach the carrying capacity, the rate of change in the population decreases. Furthermore, the graph illustrates how the population grows as a function of time. The growth quickly slows down as resources gets limited (OpenStax, 2018). This model is one of the most popular in ecological mathematics. In fact, it depicts accurately species in colonization situation. Yet, eucalyptus often deviate this smooth logistic pattern.
While the logistic model effectively captures progressive stabilization, it doesn’t take in count possible population overshoot – a situation quite frequent in fast growing organisms like eucalyptus. The Ricker function model best describes cases of population overshoot and strong density dependence. This discrete equation describes how the next generation’s population depends on the current population. This mathematical pattern found in nature models a population by time step highlighting growth dynamics over generations (Pontarp, 2025).

Where, Nt is current number of individuals in the population, Nt + 1 is the future number of individuals in the population, r is the recruitment potential (how many new recruits could be created per individuals), and K is the carrying capacity. The recruits of a population are the new individuals added to the current population.
As the current population (Nt) approaches the carrying capacity (K), the future population approaches the current population. This connects to the logistic growth model because if the population approaches the carrying capacity the population plateaus over time, meaning there is no change in population number and that the future population equals the current one. However, as the population exceeds the carrying capacity the exponential term becomes negative, and the number of recruits tends to zero. This observation makes sense since when carrying capacity is exceeded, resources become limited, and individuals alongside recruits will have difficulty to thrive.
The graph of this equation can be plotted as the future population (Nt+1 or here Xt+1) against the current population (Nt or here Xt), shown in Figure 12.

Fig. 12. Graph of Equation 23. Population recruits (Xn+1) in functions of current population (Xn).
We can see that the function peaks at a given current population which indicates that this population will yield the most recruits. This is interesting in context of agriculture and forestry for stock and biomass yield.
Plantation studies of fast-growing eucalyptus species in China revealed that when population density becomes very high (~ 2000 trees per hectare), the plantation starts to self-thin – hinting that the population has reached or exceeded it carrying capacity (William, 2017). As eucalyptus is a fast-growing tree and has a fast population growth, its populations often exceed their carrying capacity in a colonization context. Yet, the logistic model cannot take that into perspective. Consequently, the Ricker function best describes population dynamics in eucalyptus.
Empirical research confirms this pattern: as population density increases, recruitment first increases, but declines once resources vanish (Taylor, 2014). Studies use this new equation to describe the number of eucalypti recruits in function of the population density in stems per hectare.

Where r is the number of recruits, n is the number of eucalyptus stems in each area, and a & b are constants. The graph of this relationship was plotted based on collected data, shown in Figure 13.

Fig. 13. The Number of Future Recruits in Function of the Population Density in E. camaldulensi, E. largiflorens, E. melliodora and E. populnea. (Taylor, 2014)
At low densities, there are fewer mature eucalyptus able to reproduce. Subsequently, there are less recruits created by the ongoing population. As density increases, the number of adults increases, and more recruits are produced. However, beyond one point (~50 stems per hectare) eucalyptus recruit population starts to decrease. With a higher concentration, the recruit population tends to zero. This can be explained by multiple factors notably, intraspecies competition, limited resources and space, and allelopathy (see Eucalyptus Chemistry), a chemical property that inhibits growth of other plants around.
In summary, Ricker’s function provides a quantifiable and realistic illustration of eucalyptus population dynamics. By allowing researchers to model overshooting population growth and the regulation through self-thinning, Ricker’s function is used to establish sustainable harvesting practices and understand the ecological risks associated with eucalyptus population growth.
Conclusion
Eucalyptus stands as a compelling example that mathematics can bridge the gap between biology, ecology, and engineering. Through quantitative analysis, one can express the complexity of biological systems into understandable and predictable models. For example, water scarcity can be portrayed in equations of photosynthesis rate, transpiration rate, gas exchanges and stomatal conductance giving us insight on the eucalyptus drought resiliency. Similarly, leaf geometry and wettability can be depicted through Young’s, Wenzel’s and Cassie-Baxter’s equations revealing how the unique leaf microstructure of eucalyptus creates a hydrophobic surface able to conserve water and remove pathogens. At a larger scale, equation of biomass production quantifies how matter and energy move around in eucalyptus ecosystems, while population distribution and growth models capture how the genus expands in space and in numbers. From a bioengineering standpoint, predictions are indispensable in design of innovative systems inspired by nature’s efficiency. Meanwhile, for ecologists, these models and predictions are vital in the preservation of native biodiversity. In both cases, mathematics plays an essential at connecting precision and the intricacy of life. Deconstructing eucalyptus though this lens highlights the relevancy of mathematics as a unifying language bridging biology, ecology and engineering.
References
References
Almeida, A.C., & Soares, J. V. (2001). Modeling the water balance and soil water fluxes in a fast growing Eucalyptus plantation in Brazil. Journal of Hydrology, 253(1-4), 130-147. https://doi.org/10.1016/S0022-1694(01)00477-2
Austin, D., Boelkins, M., & Schlicker, S. (2017, April 27). Models for Population Growth. LibreTexts. https://math.libretexts.org/Bookshelves/Calculus/Map%3A_Calculus__Early_Transcendentals_(Stewart)/09%3A_Differential_Equations/9.04%3A_Models_for_Population_Growth
Bouvet, A., Nguyen-The, N., & Melun, F. (2013). Nutrient concentration and allometric models for hybrid eucalyptus planted in France. Annals of Forest Science, 70(3), 251–260. https://doi.org/10.1007/s13595-012-0259-3
Calviño-Cancela, M., & Rubido-Bará, M. (2013). Invasive potential of Eucalyptus globulus: Seed dispersal, seedling recruitment and survival in habitats surrounding plantations. Forest Ecology and Management, 305, 129–137. https://doi.org/10.1016/j.foreco.2013.05.037
Christina, M., et al. (2016). Importance of deepwater uptake in tropical eucalypt forest. Functional Ecology, 31(2), 509-519. https://doi.org/10.1111/1365-2435.12727
“Eucalyptus Care: Billy Heroman’s Florist: Baton Rouge, La.” Billy Heroman’s Florist, www.billyheromans.com/knowledge/flower-dictionary/eucalyptus/.
Ganassoli, Ana Paula, et al. “Wettability of Eucalyptus and Corymbia wood: Analysis of the sections and regions of the stem.” Journal of the Indian Academy of Wood Science, vol. 22, no. 1, 31 Jan. 2025, pp. 97–104, https://doi.org/10.1007/s13196-025-00364-7.
Grieve, C. M., & Shannon, M. C. (1999). Ion accumulation and distribution in shoot components of salt-stressed Eucalyptus clones. Journal of the American Society for Horticultural Science, 124(5), 559-563. https://www.ars.usda.gov/arsuserfiles/20360500/pdf_pubs/P1624.pdf
Hua Guo, Zonghan Xie, Jeremy Shaw, Kingsley Dixon, Zhong-Tao Jiang, Chun-Yang Yin, Xuemei Liu. Elucidating the surface geometric design of hydrophobic Australian Eucalyptus leaves: experimental and modeling studies. Heliyon 5 (2019) e01316. doi: 10.1016/j.heliyon.2019. e01316
Huang, R., Zhu, W., Du, A., Xu, Y., & Wang, Z. (2025). Stand Age Affects Biomass Allocation and Allometric Models for Biomass Estimation: A Case Study of Two Eucalypts Hybrids. Forests, 16(2), 193. https://doi.org/10.3390/f16020193
Jalal-Kamali, A., Ondrej Nebesky, Durcholz, M. H., Vladik Kreinovich, & Luc Longpré. (2012). Towards a “Generic” Notion of Genericity: From “Typical” and “Random” to Meager, Shy, etc.. Journal of Uncertain Systems, 6(x). https://www.researchgate.net/publication/273816744_Towards_a_Generic_Notion_of_Genericity_From_Typical_and_Random_to_Meager_Shy_etc
Khan Academy. (2016). Exponential and logistic growth. Khan Academy. https://www.khanacademy.org/science/ap-biology/ecology-ap/population-ecology-ap/a/exponential-logistic-growth
Koch, Kerstin, and Hans-Jürgen Ensikat. “The hydrophobic coatings of plant surfaces: Epicuticular Wax Crystals and their morphologies, crystallinity and molecular self-assembly.” Micron, vol. 39, no. 7, Oct. 2008, pp. 759–772, https://doi.org/10.1016/j.micron.2007.11.010.
Kurtosis and Skewness Example Question | CFA Level I - AnalystPrep. (2019, August 17). AnalystPrep | CFA Study Notes. https://analystprep.com/cfa-level-1-exam/quantitative-methods/kurtosis-and-skewness-types-of-distributions/
Lai, Y. J., Oh, P. C., Chew, T. L., & Ahmad, A. L. (2025). Surface Repellency beyond Hydrophobicity: A Review on the Latest Innovations in Superomniphobic Surfaces. ACS omega, 10(6), 5172–5192. https://doi.org/10.1021/acsomega.4c08269
Laurent Saint-André, Armel Thongo M’Bou, André Mabiala, Mouvondy, W. J., Jourdan, C., Olivier Roupsard, Philippe Deleporte, Hamel, O., & Yann Nouvellon. (2005). Age-related equations for above- and below-ground biomass of a Eucalyptus hybrid in Congo. Forest Ecology and Management, 205(1-3), 199–214. https://doi.org/10.1016/j.foreco.2004.10.006
Lenz, A. K., Bauer, U., & Ruxton, G. D. (2022). An ecological perspective on water shedding from leaves. Journal of experimental botany, 73(4), 1176–1189. https://doi.org/10.1093/jxb/erab479
Merchant, A., Callister, A., Arndt, S., Tausz, M., & Adams, M. (2007). Contrasting physiological responses of six eucalyptus species to water deficit. Annals of botany, 100(7), 1507–1515. https://doi.org/10.1093/aob/mcm234
Pausas, J. G., & Keeley, J. E. (2017). Epicormic Resprouting in Fire-Prone Ecosystems. Trends in Plant Science, 22(12), 1008–1015. https://doi.org/10.1016/j.tplants.2017.08.010
Pontarp, M. (2025). The Ricker (logistic) model. Blogspot.com. https://equation-of-the-month.blogspot.com/2014/02/the-ricker-logistic-model.html
Resquin, F., Navarro-Cerrillo, R. M., Carrasco-Letelier, L., Casnati, C. R., & Bentancor, L. (2020). Evaluation of the nutrient content in biomass of Eucalyptus species from short rotation plantations in Uruguay. Biomass and Bioenergy, 134, 105502. https://doi.org/10.1016/j.biombioe.2020.105502
Schenk H. J. (2008). Soil depth, plant rooting strategies and species' niches. The New phytologist, 178(2), 223–225. https://doi.org/10.1111/j.1469-8137.2008.02427.x
Skolmen , R. G., & Ledig, F. T. (n.d.). Eucalyptus globulus Labill. Www.srs.fs.usda.gov. https://www.srs.fs.usda.gov/pubs/misc/ag_654/volume_2/eucalyptus/globulus.htm
Taylor, J. E., Ellis, M. V., & Rayner, L. (2014). Growth, recruitment and attrition of Eucalyptus tree species in semi-arid temperate woodland. Forest Ecology and Management, 331, 25–34. https://doi.org/10.1016/j.foreco.2014.07.023
Vandermeer, J. (2010). How Populations Grow: The Exponential and Logistic Equations. Nature.com. https://www.nature.com/scitable/knowledge/library/how-populations-grow-the-exponential-and-logistic-13240157/
Wang, H., Shi, H., & Wang, Y. (2015). The Wetting of Leaf Surfaces and Its Ecological Significances. InTech. doi: 10.5772/61205
Wang, X., Fu, C., Zhang, C., Qiu, Z., & Wang, B. (2022). A Comprehensive Review of Wetting Transition Mechanism on the Surfaces of Microstructures from Theory and Testing Methods. Materials (Basel, Switzerland), 15(14), 4747. https://doi.org/10.3390/ma15144747
Williams, R. A. (2017). Open AccessJournals | List of Open Access Journals | Juniper Publishers. Juniperpublishers.com. https://juniperpublishers.com/artoaj/ARTOAJ.MS.ID.555657.php