
Table of Contents
Keywords: Maple, seed, dispersal, aerodynamic forces, durability, grain
Abstract
The maple tree, a notorious symbol of Canada’s woodland, has many physical and mechanical attributes that play a key role in species success. Over the course of evolution, it has developed these traits to defend itself from environmental difficulties that would otherwise greatly affect its chance of survival. The maple tree’s seed dispersal technique exploits aerodynamic forces, such as lift, and structural optimization, specifically its wing-like design, in the interest of decreasing descent time. With a larger range in seed distribution, the maple tree reduces the risk of competition for essential resources. Moreover, maple wood is known for its structural qualities, such as strength and durability, that can be attributed to certain evolved characteristics, namely grain arrangement, Young’s modulus (E’), specific modulus (E’/ρ), damping coefficient (tanδ) and anisotropy. These features assist the maple tree in coping with formidable challenges, such as violent storms, snow load, etc. Furthermore, these design solutions have been harnessed through biomimicry to create applications that emulate the maple trees’ physical and mechanical properties. For instance, maple seed structure and aerodynamics have inspired wind turbines for renewable energy. In addition, maple wood constitutional and vibrational traits are exploited in furniture, flooring, and musical instruments.
Introduction
The Canadian flag, the Coat of Arms of Canada and the Toronto Maple Leaves hockey team are all inspired by the official Canadian arboreal emblem, the maple tree. The leaves of this legendary tree symbolize the strength, unity and endurance of the Canadian people. In fact, the maple family, Aceraceae, has had great historical importance since the Paleogene period, when the first of its kind took root in temperate climates across the Northern Hemisphere (Prakash, 2024). Today, there exists over 100 maple species, 10 of which, including sugar, black and red maple, are native to Canada (Prakash, 2024). Other regions across North America, Europe, Asia and even Africa are all home to maple trees despite having various climates and habitats. The wide variety of populations and natural habitats specific to maple trees can be explained by the evolutionary effects of continental drift and climate change (Prakash, 2024). Indeed, roughly 200 million years ago, around the time of the Mesozoic era, the supercontinent Pangaea began to break apart. The separation of Earth’s singular landmass prompted maple species to migrate across land bridges, thereby colonizing multiple continents with distinct environments (Prakash, 2024). The ecological adaptability of the maple species continues to expand, influenced by climate change, human interference, and habitat isolation.
Maple trees have an extensive range of physical traits that can vary wildly between diverse species. Some maples can be exceptionally large, towering up to 35 meters tall, while others can be significantly smaller, reaching less than 10 meters high (Farrar, 2000). Furthermore, as shown is Figure 1, despite having similar basic characteristics, maple leaves have unique shapes amongst species. In fact, maple leaves can take on a simple form (Fig. 1 all except f), having a singular broad blade, or a compound form (Fig. 1 f), having two or more leaflets (smaller leaflike sections) on each petiole (Glimn-Lacy & Kaufman, 2006). The maple species have palmately veined leaves, meaning their veins originate at a single point and disperse like fingers from a palm (Grimm, 2002). In general, maple leaves have 3-9 toothed lobes (Fig.1), where each lobe corresponds to a prominent vein (Farrar, 2000). Finally, Maple trees are characterized by an opposite arrangement in which the leaves grow in pairs, across from each other along the stem (Glimn-Lacy & Kaufman, 2006).

Fig. 1. Distinct leaf morphologies of 9 different maple species. (a) Silver Maple morphology, (b) Red Maple morphology, (c) Bigleaf Maple morphology, (d) Striped Maple morphology, (e) Mountain Maple morphology, (f) Manitoba Maple morphology, (g) Sugar Maple morphology, (h) Vine Maple morphology, (i) Black Maple morphology, modified from Spence (Spence, 2025).
The maple tree undergoes significant seasonal changes. Indeed, the Aceraceae family is of the deciduous kind, meaning it sheds its leaves annually, marking the end of a growing period (Farrar, 2000). Maple foliage is famous for its spectacular display of radiant colours during this growth cycle, particularly during autumn. In fact, as winter approaches and North American temperatures drop, the chlorophyll responsible for the leaves' green colour breaks down. Thus, alternative pigments, such as yellow carotenoid pigments, are more pronounced (Matile, 2000). However, anthocyanin, a pigment responsible for other colours such as red, is not revealed by chlorophyll degradation. Instead, this pigment is synthesized by the leaves at the midpoint of their biological degradation, which occurs during autumn. (Lev-Yadun & Gould, 2007). (see Maple Chemistry)
The maple tree, alike most living organisms, has developed several very interesting mechanisms to increase survival. In fact, in the interest of minimizing competition, the Aceraceae family has developed a distinctive dispersal technique for its seed (Seale & Nakayama, 2020). First, the fruit of the maple tree is winged and is assembled in pairs, called samaras (Farrar, 2000). Thus, the samara contains two fruits, often referred to as keys, that each hold a seed (Farrar, 2000). As a result of its optimal structural design, the maple seed utilizes natural winds to increase dispersal. Indeed, components such as size and wind curvature give rise to a helicopter-like mechanism that maximises the maple seeds’ descent time (Seale & Nakayama, 2020). Therefore, by favoring a broad dispersal of its seeds, the maple tree limits the chance of overpopulation in a particular area of land.
Maple Seeds
Structure of Maple Seeds and Rotation
Maple seeds, also known as samaras, have a unique structure that grants them their slow descent through their rotational motion. This allows them to disperse wider and to germinate far from the parent tree, which results in several advantages. For instance, the further the new tree is from its parent, the less they compete for resources, thereby increasing their chance of survival. Avoiding competition with the parent tree for resources, escaping environments that can get compromised and adapting to diverse and unknown habitats, are among the other advantages of seed dispersal (Beckman & Sullivan, 2023). The underlying reason for this elegant dance resides in the structure of the seed. The samara is composed of two parts: a central nutlet containing the embryo, and a wing-like fibrous, flat and thin leaf structure with a thicker leading edge elongating from the center (El Makdah et al., 2022). Different maple seeds are presented in Fig. 2, as well as a tomographic image to highlight its structure in Fig. 3.
Precession, Rotation and Gyration are different ! Precession is wobble of the spinning axis of an object (gyroscope). Gyration is the motion in a circular path around an axis. Rotation is the spin around the object’s axis.

Fig. 2. Examples of maple seed morphologies (Schaeffer et al., 2024).
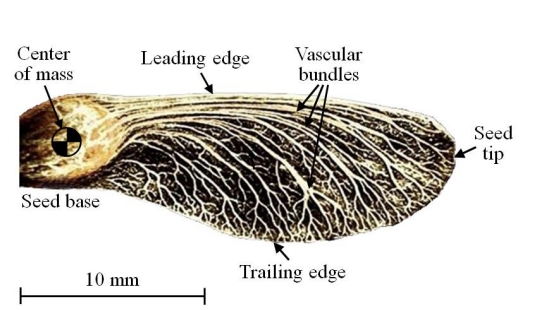
Fig. 3. Tomographic 3D image of the maple seed (A. palmatum) (Sohn, 2016).
Two samaras can join in their center and produce what is known as a double samara, with the two nutlets adjoined at the middle and one wing on each side, at a slight angle. These wings, through autorotation around its nut center, generate a high aerodynamics force, known as lift, that opposes the weight of the seed and allows for it to glide, significantly increasing the descent time (El Makdah et al., 2022). The surface area of the wing, increases the contact surface with the air, therefore accentuating the effect of drag, which also favors a slower descent (Schaeffer et al., 2024).
As it falls, the maple seed takes its characteristic helical motion traced by the seed tip (Fig. 5) (Varshney et al., 2011). However, this motion goes through some turbulence which is known as the transition phase before attaining its steady state. This transition occurs through 3 steps: a tumble about the span-wise direction (z-axis), then a tilt in the chord-direction (y-axis), which evolves into rotation (Varshney et al., 2011), and finally a steady rotational motion, accompanied by the opening of a cone angle (Fig. 4).

Fig. 4. Geometrical configuration of the seed during its free-fall together with Euler angles and the symbols used. Dashed (yellow) lines show laboratory axes whereas dotted (red) lines show local seed axes (Varshney et al., 2011).
Unexpectedly, even samaras with cut wings achieve this rotation, although their deceleration suffers from the weakening of the aerodynamics forces. Experiments were conducted where maple seeds were progressively cut from their wing tip to their nut center, and their rotation was studied. Samaras that kept a fraction of their leading edge were still able to achieve rotation. It is only when only the seed base is kept and the rest is removed, meaning there is no aerodynamic forces, that the seed plummets to the ground (Varshney et al., 2011). In order to study this, multiple samaras with progressively cut wings or nuts were filmed during their descent (Table 1).
Table 1. Free flight parameters of free-falling seeds in steady state after removing wings as well as nut gradually (Varshney et al., 2011).

Looking at the measured values for the free-falling seeds with gradual wing cutting (0 is uncut,5 is fully cut), the descent velocity (Vz) drops drastically, highlighting the importance of the aerodynamic forces generated by the wing. However, the rotation does not stop. In fact, the angular velocity seems to increase as the wing is cut. Apart from that, the cut seed and uncut one seem to be falling with the same path, keeping a relatively similar cone angle (Varshney et al., 2011).
Using a high-speed camera and an appropriate experimental setup, it is possible to study the kinematics of the free fall of the samaras, particularly the uncut one and the 4th cut (Fig. 5).

Fig. 5. Side views of typical trajectories of a falling maple seed with intact and cut wings (Varshney et al., 2011).
Looking at first at the maple seed, one would think that the torque generated by the aerodynamic forces would be the underlying reason for the rotation. However, this rotation is still obtained with a cut seed but vanishes completely once these forces are nullified. This suggests that the aerodynamic forces are important to maintain the steady rotation, but are not the only mechanism for the autorotation of the maple seed (Varshney et al., 2011).
The autorotation mechanism can be explained by examining carefully the transition phase before the seed attains steady rotation, and by understanding the implications of the structure of the seed and the mass distribution. The nutlet concentrates most of the mass, whereas the wing is lighter. The linear mass density can be determined by sectioning the seed and weighing every section (Fig. 6).

Fig. 6. Sectioning and weighing of maple seed. (a) A Norway maple seed (Acer platanoides) is sliced into sections and weighed in order to estimate the spanwise linear mass density, that is, mass per unit spanwise length, (b), shown on a relative scale for 30 natural Norway maple seeds, as well as an average and the center of mass(Nave et al., 2021)
The center of mass, as shown in Fig. 6, is calculated based on a weighted sum of every position. However, in order to understand the underlying mechanism of the rotational movement, it is more pertinent to look at the mode of the mass distribution to visualize where the gravity forces are the most concentrated, but also the mode of the area distribution, as they indicate where the drag is the most concentrated. Using MATLAB, and by making an approximation using a Maxwell-Boltzmann distribution, the allure of both distributions can be sketched (Fig. 7)
In statistics, the mean is obtained by adding numbers and dividing by how many there are. The median is the middle number when the set is ordered. The mode is the most frequent value. In the mass context, it is the position where the mass is the highest.

Fig. 7. Mass and Area distribution across a maple seed (Own work by Rayene Zanina).
The mode in the mass distribution corresponds to the nutlet, and the gravitational forces are the strongest at that position. The mode in the area distribution is in the middle of the wing part of the seed, and the drag is the most intense at that position. After its release, gravity pulls more on the nutlet than the wing. The maple seed experiences air damping, which is the resistance of the air to the motion of the seed, and generates a drag force that concentrates at the wing. The offset between the gravitational forces and the drag forces, each acting on the leaf in a different direction, leads to a first tumble along the span wise direction, which has the lowest moment of inertia, then the seed is tilted up about the chord direction. The chord direction is inherently unstable, and the rotational energy due to the torque is fed into the other directions, initiating the helical motion (Varshney et al., 2011). The tilt along the chord direction leads to a tangential component in the aerodynamic forces, leading to a torque, hence the rotation.
Another consequence of the uneven mass distribution that further strengthens the lift generated by the wing (which will be covered in more detail in the second subsection) is the low moment of inertia of the maple seed. The definition for the moment of inertia is as follows:

Where I is the moment of inertia, r is the distance from the axis and m is the mass. The farther the mass is from the axis of rotation, the more it will account for in the moment of inertia. However, for the samara, most of the mass in concentrated in the nutlet, near the rotation axis. Consequently, maple seeds have low moment of inertia, which results in a higher angular velocity, with respect to the following formula:

Where L is the angular momentum and ω is the angular velocity. This can be rearranged as:

This means that, the structure of the seed favors a higher rotation velocity, which increases the lift force.
It seems that there are 3 components to achieve auto rotation: uneven mass distribution, air damping leading to a tilt and aerodynamic forces to reach the steady rotational state (Varshney et al., 2011).
Aerodynamics of Maple Seed and Force Modelling
As they descend, maple seeds are able to generate high lift with very high performance despite their relatively small size and small angular velocity, if we compare them to a helicopter which has similar mechanisms. This lift can be attained by generating a compact and stable leading-edge vortex (LEV) as the seed descends, which is the aerodynamic solution that hovering insects and bats also rely on (Lentink et al., 2009). These were demonstrated using numerical methods and applications of Navier-Stokes equation to simulate the flow of air (Chen & Lan, 2022). A leading-edge vortex is stable vortex of air flowing that remains attached to the leading edge. The air flowing around the maple seeds swirls above the upper surface of the maple seed along its span near the leading edge, generating a negative pressure area on the leeward surface (Fig. 8). This leads to a suction in the upwards direction, which is the physical phenomenon that generates the lift force (Chen & Lan, 2022). LEVs are not uniform across the wing’s span. They are tighter near the nutlet, but get larger as we get further away, then thin at the tip (Fig. 8).

Fig. 8. Flow field characteristics of the maple seed. (a) Dimensional vorticity in the y direction on the cross section at three spanwise locations: 0.25 R, 0.5 R, and 0.75 R from the rotation center, respectively. (b) Dimensional pressure distribution on the windward and leeward surfaces of the maple seed (Chen & Lan, 2022).
Leading Edge Vortices (LEV) depend on multiple factors, such as the shape of the maple seed, but also the wing’s angle of attack, which is the angle between the wing and the incoming flow, and Reynolds number Re. This dimensionless quantity represents the ratio of inertial and viscous forces. Reynolds number allows to predict fluid flow patterns. A low Re means the flow is laminar and smooth, whereas a high Re can indicate turbulence and chaotic behaviours. This number can be defined as follows:

where ρ is the fluid density, V is the flow velocity, L is the characteristic length and μ is the dynamic viscosity of the fluid. Measurements in a vertical wind tunnel show that maple seeds flow at angles of attack ranging from 12° to 32°, and Reynolds numbers of order of magnitude 1000 (Lentink et al., 2009). The Reynolds number for these measurements lies in a middle range indicating a transitional regime between laminar and turbulent flow. Viscous forces are significant, as shown in the formation of vortices, but are not totally taking over inertial forces, avoiding chaotic behaviour and maintaining a stable state.
A very simply model for the forces acting on the maple seed can be proposed in order to conduct a classical mechanics study on the samaras (Fig. 9).

Fig. 9. Force equilibrium with seed in autorotation. L is the lift force, D is the drag force and Fz is gravity (Desenfans, 2019).
Once steady state is attained, the seed reaches a terminal constant velocity, meaning the acceleration is null, and that the sum of forces is zero. From that, we derive the equality:

where Fz is the gravity force, L is the lift and D is drag. Forces can be modelled using the following equations:
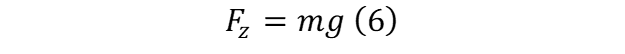
where m is the mass and g is the gravitational acceleration. Lift can be modelled using this equation:

where ρ is the fluid density, Vrad is the radial velocity, CL is the lift coefficient and S is the area. The radial velocity depends on the radius as well as the angular velocity Vrad = ωR , meaning the lift force can be expressed as:

Lift is proportional to the square of the angular velocity, which shows how having a small moment of inertia can lead to high lift forces. Drag can be modelled with the following equation:

where Vz is the descent velocity, CD is the drag coefficient.
The lift and drag coefficients are defined as dimensionless quantities and can be measured empirically.

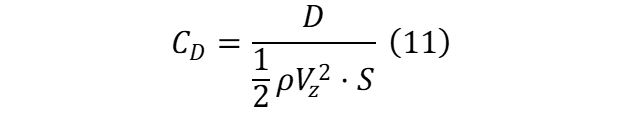
The angular velocity can be assumed to be an average value from empirical measurements, being 86.29 rad/s (Desenfans, 2019).
It is then possible to compute the descent velocity from known parameters. One example of calculation is done using this method, from the following parameters (Table 2).
Table 2. Known parameters of example seed and assumed value for calculations (Desenfans, 2019).
| g (m/s2) | ρ (kg/m3) | cL | CD |
| 9.81 | 1.225 | 1.0586 | 1.98 |
| m (mg) | S (mm2) | ω (rad/s) | vz (m/s) |
| 170.6 | 612.8 | 77.9 | 0.94 |
Using the equality, the velocity can be calculated to be 0.84 m/s. This value is not precise, due to a lot of assumptions and simplifications made. Complicated numerical methods are used to generate a better estimate for the value. Ultimately, the study reaches a value of 0.89 m/s, which deviates 5.47% from the measured velocity (Desenfans, 2019). By using the fact that red maple species grow on average to be 21.3 meters tall, the study compares the freefall time for an object with no aerodynamic forces, and the maple seed falls 11.4 times longer in the air (Desenfans, 2019). This means that, assuming constant horizontal velocity, maple seed’s aerodynamic forces allow it to be dispersed 11.4 times farther than a regular object. However, it is important to mention that this is simply one example of calculation on one specific seed, but it is still a good way to get some sort of idea on how efficient this slow descent is.
Resistance of Maple Seeds to Natural Environments
In the previous sections, the motion of the maple seed was mostly studied launched from rest in vertical wind tunnels, where no external forces, such as wind, are interfering. These ideal settings allow for a thorough study of the rotation mechanism. However, these settings are very different from natural environments that introduce multiple factors affecting the samara.
In nature, intense wind gusts and the elastic recoil of the branching can detach the maple seed with a high initial impulse vertically or horizontally (Ortega-Jimenez et al., 2019). It is important to highlight that, high winds mean a high flow velocity, which could lead to high Reynolds numbers that can reach orders of magnitude of 104. This would mean that the motion becomes much more turbulent and unstable. From the previous section, it is known that maple seeds rely on stable LEVs that remain attached to the wing in order to generate lift though the pressure difference (Chen & Lan, 2022). A high turbulence in the flow may compromise the aerodynamic performance of the maple seed (Ortega-Jimenez et al., 2019). To study maple seeds behaviour in such conditions, maple seeds were launched horizontally and vertically using a catapult. Their motion was studied using high-speed cameras, and the translational speed ut, the deceleration at as well as the rotational frequency n were measured (Fig. 10).

Fig. 10. Behaviour of maple seeds over time at steady-state(black), vertical launch(red) and horizontal launch(blue). Translational velocity(a), deceleration(b) and angular frequency(c) as a function of time (Ortega-Jimenez et al., 2019).
The steady state descent was characterized by a descent velocity around 1.0 m/s. Maple seeds that were thrown at initial speeds varying from 7 m/s to 10 m/s decelerated at maximum values around 6g for the horizontal launch and 12g for the vertical launch, reaching their minimum descent speed at 140-150 ms. Their rotational velocity is higher than the steady state frequency, indicating stronger lift forces, but it quickly drops. However, maple seeds that were launched took longer to enter a stable autorotation motion (Fig. 10). A very interesting observation is that the deceleration is initially relatively weak, but increases as the maple seeds settle into rotation, and experience their peak when maple seeds reach stable autorotation motion. Both proceed to drop over time. This shows that the maple seed is capable of resisting these high initial impulsions by generating strong lift forces to quickly decelerate and reach a steady state. Initial settings do not stop the maple seed from reaching its equilibrium, and random tosses always end in the same rotation (Varshney et al., 2011). Maple seeds are thus capable of resisting turbulence, making it even better at dispersal, as atmospheric models predict that turbulence significantly increases. Samaras turn these chaotic events into an advantage, as the higher rotational frequencies measured can lead to stronger lift forces, which result in height gain and ultimately farther dispersal (Ortega-Jimenez et al., 2019).
Another factor that could alter the dispersal of the maple seeds are the mass fluctuations. Samaras are susceptible to environment moisture or resting insects, as well as drying as they turn from green to brown. However, maple seeds seem to always be able to rotate. They must then possess a resistance to these mass fluctuations (Schaeffer et al., 2024). In order to study the behaviour of maple seeds under different mass fluctuations, maple seeds were either dunked in molten wax for mass addition, or their nutlets are shaved off for mass reduction, with varying degrees. Their reduced descent velocity, reduced angular velocity, reduced cone angle and drag are then plotted versus the reduced mass for different species of maple trees. The reduced quantity is the dimensionless ratio of the altered value and the unaltered one (Fig. 11).

Fig. 11. Behaviour of maple seeds for different species after mass addition or reduction and the fit. Reduced velocity(a), angular velocity(b) and cone angle(c) as a function of reduced mass, as well as drag vs gravity (d) (Schaeffer et al., 2024).
The descent velocity is lightly altered, with a 5% increase for a 50% mass increase. However, the response in angular velocity is more important. The fit shows a 50% increase in the rotation velocity for a 50% mass increase (Fig. 11), and thus high lift forces can increase to up to 125% using the previous lift force model (The lift force is proportional to the square of the angular velocity). This is the first hypothesized reason for the little influence of mass fluctuation. Another explanation is the smaller cone angle when mass is added, which makes the maple seed flatter, and causes an increase in the aerodynamics forces (Schaeffer et al., 2024). It must be noted that that this study uses a slightly different model for both aerodynamics forces. These mechanisms are key to the little influence of mass fluctuance, specifically mass addition, on the descent velocity and the samara’s resistance to mass alteration.
Physical & Acoustic Properties of Maple Wood
Maple wood possesses a plethora of physical properties that enable it to overcome everyday challenges posed by nature. Maple trees are susceptible to damage by storms, wind, and more; said damage can be categorized into dynamic and static loading. Maple trees may be whipped back and forth by the dynamic force of wind and storms, or subject to static force from snow or ice loading of the branches and limbs, both of which are common occurrences due to the geographic distribution of maple species (Lilly & Sydnor, 1995).
The behavior of maple wood is characterized by its many vibrational and physical properties, including grain arrangement, Young’s modulus (E’), specific modulus (E’/), damping coefficient (), and their anisotropy between longitudinal (L) and radial (R) directions (Alkadri et al., 2018). The damping coefficient is a parameter that quantifies how quickly a system’s oscillations dissipate due to external forces like friction. The Young’s modulus is a property in physics that refers to a material’s resistance to deformation under axial stress, hence providing a measure for its stiffness. Whereas the specific modulus is a ratio calculated by dividing the Young’s modulus by the material’s density. The anisotropy delineates direction-dependant growth patterns in trees, and the microfibril angle, MFA (Fig. 12) describes to the orientation angle of cellulose microfibrils within the secondary cell wall of wood fibres, relative to the longitudinal axis (Petroudy, 2017).

Fig. 12. Image displaying the difference between a high (A) and low (B) microfibril angle (MFA) and their influence on longitudinal and transverse shrinking (Hein, 2011).
Maple wood, specifically sycamore maple wood, possesses a unique wavy grain arrangement, resulting from undulating, S-shaped fiber growth in the wood. This is a unique fibre pattern, that deeply benefits maple wood’s acoustic properties as well as the stability of the sycamore maple tree. A 2018 study quantified the correlation using Pearson’s coefficient between this waviness of sycamore maple fibres (Fig. 13) and its vibrational properties. The grain angle (Fig. 14) and degree of waviness was calculated as a ratio of the amplitude to the wavelength, using the formula w=A/, the value of which was then used to quantify this correlation. The microfibril angle was measured on radial sections stained with iodine-potassium iodide using light spectroscopy, and the waviness parameters were determined by scanning images of split wood blocks, assuming a sinusoidal wave model. The study revealed a positive correlation between the grain waviness and the microfibril angle (r=0.45-50), as well as the damping coefficient (Alkadri et al., 2018). However, it was found that the wavy grain sycamore exhibits a lower specific modulus, and that waviness correlates negatively with the specific modulus, which can be explained by the undulations causing the wood fibres to change orientation, leading to a decrease in stiffness. This all works in favor of the sycamore and its stability; its wavy fibre orientation causes more internal friction and energy loss as waves propagate through the wood (Dinulica et al., 2023), hence the high damping coefficient. The high microfibril angle aids in preventing the tree’s collapse due to resonance by making the wood more flexible and less stiff, dissipating vibrational energy rather than allowing it to build up, similarly to the wavy grain’s internal friction.

Fig. 13. Diagram displaying a split block, measuring the parameters of wavelength and amplitude of the fibre waviness (Alkadri et al., 2018).

Fig. 14. Description of grain angle measurement (Alkadri et al., 2018), where the angle in radians can be calculated using the following equation:

A tree and its branches can be thought of as a system of cantilevers; systems of projecting beams fixed at one end are free to oscillate. Cantilevers deflect depending on the load applied and their flexural strength — the product of the Young’s modulus and the second moment of area. They can also face deformation due to resonance, a phenomenon in which the natural frequency of a cantilever’s vibrations matches the frequency of oscillations of external forces, causing an aggressive and rapid rise in amplitude of oscillations, leading to structural failure. This is a common issue trees face in nature; resisting deformation due to resonance with ubiquitous environmental forces such as wind gusts. The natural frequency of a cantilever — and hence a tree and its branches — can be described through the following formula:
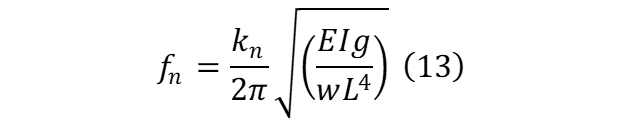
Where E is the material’s Young’s modulus, I is the moment of inertia of the cantilever’s cross section, w is the load per unit length applied on the cantilever, L is the cantilever’s length, and Kₙ is constant parameter that varies depending on n, which refers to the mode of vibration (Budynas & Sadegh, 2020). From this equation, it can be inferred that the natural frequency of vibration is directly proportional to the square root of the wood’s Young’s modulus, a property that was proven to have a negative correlation with grain waviness in the wood, since the specific modulus is simply a ratio of the Young’s modulus to the density. Hence, it can be assumed that in the context of the referenced study, sycamore maple wood branches would have a relatively lower natural frequency. This is favorable for the tree and its structural stability, as it allows them to avoid the frequencies of common natural forces and keep them out of range (Fig. 15), remaining better tuned to dissipate vibrational energy (James, 2014). This reduces the risk of the tree collapsing or experiencing structural failure due to resonance with external forces. Moreover, lower frequencies are associated with lower deflections, which reduces the stress on the branch.

Fig. 15. Graph displaying the relationship between the frequency, resonant frequency, and amplitude (Meney, 2025).
The vibrational and physical properties of sycamore maple wood that have been studied, quantified and measured by scientists reveal themselves to be a perfectly engineered system of properties when analyzed on a microphysical level; working together to cope with nature’s everyday challenges and keep the sycamore maple tree standing. From a bioengineering perspective, the fascinating and complex systems within maple wood can inspire many real-world design solutions, ranging from applications in music due to its favorable acoustic properties — which could also aid in interior design — to resonance resistant beams.
Conclusion
Maple trees have evolved by developing physical properties that enable them to adapt to the environment’s stresses and competition. First, the winged shape of samaras allows them to be carried by the wind, thus promoting seed dispersion. Three components minimize the rate of fall by causing autorotation:
The uneven mass distribution concentrated near the nutlet lowers the moment of inertia and stabilizes the autorotation, which generates sufficient lift.
An optimized surface area of the wing maximizes air damping during the turbulent phase, increasing drag and slowing the fall rate.
Wing features, such as spanwise thinning, sustain the formation of stable leading-edge vortexes. Well-balanced proportions and structures allow a smooth transition in the intermediate flow, at an angle of attack between 12 ° and 32 °, favor steady LEVs, and increase lift.
As a result, the fall is significantly slower than that of a regular similar-sized object lacking aerodynamic optimization. There are parameters that compromise seed dispersion. However, maple seeds display resistance to certain unfavorable conditions.
High turbulence in the flow causes changes in aerodynamic forces that challenge the seed’s performance. However, even under high Reynolds number conditions, the seed counters high initial impulsion with better lift forces, thanks to greater angular velocity.
The presence of moisture and insects causes the mass of the seed to fluctuate, for instance. However, maple seeds exhibit resistance to such changes. The mass increase causes rising descent velocity, but this effect is canceled by a greater angular velocity and a smaller angle of cone formation, making the seed flatter and subject to stronger aerodynamic forces.
The samara’s auto-rotating trajectory and geometric features inspired the design of low-scale bioinspired wind turbines (Omidvarnia & Sarhadi, 2024).
Second, Maples grow in harsh environments that expose them to wind loads and extreme weather. Consequently, maple wood evolved to resist static and dynamic loading. More particularly, the resistance of sycamore wood is a result of the wavy grain arrangement, caused by the S-shaped fiber growth that provides stability.
The study of a sinusoidal wave model reveals that high wavy patterns lead to low specific modulus, and therefore less stiffness, causing more internal friction to disperse shock waves.
Similarly, high microfibril angles prevents collapse due to resonance by dissipation of vibrational energy. The model was further simplified by comparing it to a system of cantilevers. Wave formulas demonstrate how the low specific modulus of the wood provides low natural resonance frequencies, which is ideal to prevent matching frequencies with surrounding forces.
It's important to note that sycamore trees exhibit this physical trait more prominently. Nonetheless, other maple species also display similar patterns, though to a lesser extent.
One of the most direct applications of maple wood’s acoustic qualities is the design of string musical instruments. Studies revealed that increasingly defined wave patterns, which correlates negatively with the wavy-grain pattern wavelength, indicates more pronounced undulations, and hence a higher quality of sound, as well as a highly efficient sound propagation along the longitudinal direction of the wood. (Dinulica et al., 2023). This said, these acoustic qualities make wavy grain sycamore maple wood ideal for crafting musical instruments.
References
References
Alkadri, A., Carlier, C., Wahyudi, I., Gril, J., Langbour, P., & Brémaud, I. (2018). Relationships between anatomical and vibrational properties of wavy sycamore maple. Iawa Journal, 39(1), 63-86. https://doi.org/10.1163/22941932-20170185
Beckman, N. G., & Sullivan, L. L. (2023). The Causes and Consequences of Seed Dispersal. Annual Review of Ecology Evolution and Systematics, 54(1), 403-427. https://doi.org/10.1146/annurev-ecolsys-102320-104739
Budynas, R. G., & Sadegh, A. M. (2020). Roark's formulas for stress and strain. McGraw-Hill Education.
Chen, T. T., & Lan, S. L. (2022). Numerical analysis of dynamic stability of falling maple samaras. Acta Mechanica Sinica, 38(12), 322111. https://doi.org/10.1007/s10409-022-22111-x
Desenfans, P. (2019). Aerodynamics of the Falling Maple Seed. In: Aircraft Design and Systems Group (AERO).
Dinulica, F., Savin, A., & Stanciu, M. D. (2023). Physical and Acoustical Properties of Wavy Grain Sycamore Maple ( L.) Used for Musical Instruments. Forests, 14(2), 197. https://doi.org/10.3390/f14020197
El Makdah, A. M., Zhang, K., & Rival, D. E. (2022). On the robust autorotation of a samara-inspired rotor in gusty environments. Bioinspir Biomim, 17(4), 044001. https://doi.org/10.1088/1748-3190/ac68bb
Farrar, J. L. (2000). Trees in Canada (7 ed.). Fitshenry & Whiteside Limited
Glimn-Lacy, J., & Kaufman, P. B. (2006). Botany illustrated : introduction to plants, major groups, flowering plant families (2nd ed.). Springer. https://doi.org/10.1007/0-387-28875-9
Grimm, W. C. (2002). Illustrated book of trees: the comprehensive field guide to more than 250 trees of eastern North America. Stackpole Books.
Hein, P. R. G. (2011). Genetic and environmental control of microfibril angle on Eucalyptus wood: its effects on wood traits and implication for selection Université Montpellier II-Sciences et Techniques du Languedoc].
James, K. R. (2014). A study of branch dynamics on an open-grown tree. Arboriculture & Urban Forestry (AUF), 40(3), 125-134.
Lentink, D., Dickson, W. B., van Leeuwen, J. L., & Dickinson, M. H. (2009). Leading-edge vortices elevate lift of autorotating plant seeds. Science, 324(5933), 1438-1440. https://doi.org/10.1126/science.1174196
Lilly, S., & Sydnor, T. D. (1995). Comparison of branch failure during static loading of silver and norway maples. Arboriculture & Urban Forestry (AUF), 21(6), 302-305.
Matile, P. (2000). Biochemistry of Indian summer: physiology of autumnal leaf coloration. Exp Gerontol, 35(2), 145-158. https://doi.org/10.1016/s0531-5565(00)00081-4
Meney, D. (2025). structure vibration-how,much is too much?: Yemen. Yenem Engineering services.
Nave, G. K., Jr., Hall, N., Somers, K., Davis, B., Gruszewski, H., Powers, C., Collver, M., Schmale, D. G., 3rd, & Ross, S. D. (2021). Wind Dispersal of Natural and Biomimetic Maple Samaras. Biomimetics (Basel), 6(2), 23. https://doi.org/10.3390/biomimetics6020023
Omidvarnia, F., & Sarhadi, A. (2024). Nature-Inspired Designs in Wind Energy: A Review. Biomimetics (Basel), 9(2), 90. https://doi.org/10.3390/biomimetics9020090
Ortega-Jimenez, V. M., Kim, N. S., & Dudley, R. (2019). Superb autorotator: rapid decelerations in impulsively launched samaras. J R Soc Interface, 16(150), 20180456. https://doi.org/10.1098/rsif.2018.0456
Petroudy, S. D. (2017). Physical and mechanical properties of natural fibers. In Advanced high strength natural fibre composites in construction (pp. 59-83). Elsevier.
Prakash, I. (2024). Comprehensive Review of Maple Trees: Evolution, Biogeographical Distribution, Ecology, and Economic Significance with Emphasis on Canada. Indian J. Ecol, 15, 1418-1423.
Schaeffer, B. M., Truman, S. S., Truscott, T. T., & Dickerson, A. K. (2024). Maple samara flight is robust to morphological perturbation and united by a classic drag model. Communications Biology, 7(1), 248. https://doi.org/10.1038/s42003-024-05913-3
Seale, M., & Nakayama, N. (2020). From passive to informed: mechanical mechanisms of seed dispersal. New Phytol, 225(2), 653-658. https://doi.org/10.1111/nph.16110
Sohn, M. H. (2016). Aerodynamic Features of Maple Seeds in the Autorotative Flight. Journal of the Korean Society for Aeronautical and Space Sciences, 44(10), 843-852. https://doi.org/10.1016/j.mechrescom.2023.104104
Varshney, K., Chang, S., & Wang, Z. J. (2011). The kinematics of falling maple seeds and the initial transition to a helical motion. Nonlinearity, 25(1), C1.