
Table of Contents
Abstract
The Ficus genus demonstrates ecological optimization and survival through its mathematical patterns. Its physical form operates as an efficient biological network, where graph theory reveals a balance between minimal transport paths and resilient, looped structures. Allometric scaling governs its growth, strategically trading hydraulic efficiency for mechanical strength, while its fractal canopy, which is modellable by Lindenmayer systems, maximizes light capture. These principles extend to the roots, where strangler fig growth in particular, mirrors computational models like diffusion-limited aggregation, providing a blueprint for biomimetic design and structural engineering.
Introduction
Ficus trees are a 75-million-year-old keystone species mostly situated in rainforest or savanna territories. The trees range from large banyan trees to small shrubs. For example, the banyan tree, the Ficus benghalensis, develops a large canopy which provides shade for a significant area and can extend between 30-200 meters in diameter. Furthermore, the Ficus species forms nursery mutualistic relationships with wasp species where the fig fruit is a breeding site for wasp larvae, and the wasp aids the Ficus pollinate. The Ficus are aggressive conquerors of their environment: the Ficus aurea, the strangler fig, forms a pseudo trunk by choking a host tree’s trunk with its roots, ultimately killing the host tree for its ecological benefit (Aumeeruddy-Thomas & Hossaert-McKey, 2024).
Beneath this fractal canopy, Ficus networks operate like living graphs which are rooted, branching systems that optimize flow, stability, and communication. By applying graph theory, its structure can be understood as an evolving network that minimizes transport distance while maximizing resilience, a balance achieved through both acyclic and cyclic configurations. The structural and physiological success of Ficus trees lies in their ability to balance energy capture, water transport, and mechanical stability through efficient scaling strategies. As they expand from small saplings into towering giants, Ficus species must continuously optimize the relationship between form and function. Allometric scaling provides a better understanding of these adjustments, revealing how proportional growth patterns sustain hydraulic conductivity, mechanical resilience, and metabolic efficiency. This section explores how Ficus species apply fundamental scaling laws to distribute resources effectively, maintain hydraulic flow under variable conditions, and reinforce mechanical integrity. All of which contribute to their ecological dominance and longevity. Ficus trees such as the Ficus benghalensis (bayan tree) form large tree crowns which are the branches, foliage and flowers growing above the tree trunk (Patrut et al., 2023). Traditional Euclidean geometry provides an essential framework for describing idealized, human-made forms like lines, planes, and spheres. However, it proves insufficient for capturing the irregular and intricate shapes found throughout nature. These complex forms are better described by fractal geometry. A fractal is a shape that is infinitely complex and self-similar, meaning its smaller components resemble the overall structure. For example, a small twig reflects the branching pattern of a larger limb, which in turn mirrors the entire tree. This unique complexity leads to a defining property, a fractional dimension. In traditional geometry, the dimension of a space is defined by the number of vectors needed to span it. A fractal’s dimension, however, does not fit these whole-number categories. Instead, it is a measure of how completely a fractal fills space and its complexity (Amir et al., 2010). The recursive branch growth in Ficus crowns and canopies can be molded with Lindenmayer systems. The fractal patterns in the Ficus tree allow the tree to survive and become a keystone species in its environment. Strangler figs (Ficus) are remarkable examples of natural engineering, capable of stabilizing even steep stone walls through intricate networks of roots. Their growth patterns, both adaptive and fractal, resemble processes seen in diffusion-limited aggregation (DLA), where structure emerges from random motion and accumulation. Modeling these dynamics offers insight into how biological systems achieve stability through self-organization, bridging ecology, mathematics, and design (Prusinkiewicz & Lindenmayer, 1990).
See Ficus Physics for an extensive introduction
Graph Theory & Network Topology of Roots and Branches
The Rooted Tree Graph
Graphs have been developed to depict the intricate geometry of Ficus trees, capturing the complexity of their natural design. The trunk acts as the root node, branches as edges, and each budding junction as a vertex in nature’s equation. Over time, the tree appears to “compute” the most efficient design, minimizing effort while maximizing reach (Prusinkiewicz & Lindenmayer, 1990).
In mathematical terms, the Ficus can be represented as a rooted tree graph, a connected acyclic network described by fundamental parameters. The average vertex degree

expresses how many branches (edges, E) emerge per node (N), while the average path length

measures the mean distance between nodes. These parameters express the balance between connectivity and efficiency. A high vertex degree increases canopy reach but raises hydraulic cost, while a smaller degree conserves energy but limits sunlight capture. The Ficus achieves an equilibrium close to a minimum spanning tree, minimizing total edge length while maintaining reach (Barthelemy, 2011) (Fig. 1).
This trade-off between construction cost and spatial coverage is visualized in spatial network models, where denser connectivity shortens mean path length L at the expense of additional edges. Algorithmic models make this hidden logic visible. L-system simulations generate recursive, self-similar patterns resembling real growth (Prusinkiewicz & Lindenmayer, 1990; Sharma & Tiwari, 2017), while the space colonization algorithm allows branches to grow toward unoccupied space. This is precisely how Ficus canopies expand (Runions et al., 2007). The fractal character of Ficus branching can be quantified by its dimension:

where N is the number of self-similar sub-branches at scale. Empirically, Df is about 2.3-2.5, balancing planar expansion and volume fill.
Physiologically, this geometry translates to function. Within each edge of the network, xylem conduits transport water and nutrients according to the Hagen–Poiseuille law:

Large, short vessels near the trunk taper into finer capillaries at the periphery, optimizing hydraulic resistance and safety (Brodribb et al., 2023; Sack et al., 2008; Zwieniecki et al., 2002).

Fig. 1. This figure illustrates a spectrum of spatial network geometries that highlight the trade-off between construction cost and transport efficiency. (a) Sparse, tree-like structure with no loops. (b) Hierarchical branching with occasional reinforced loops. (c) Dense radial network with limited cross-links. (d) Highly loopy, mesh-like structure with extensive cross-connections that minimize path length but raise construction cost. Among these, (b) most closely resembles Ficus root systems, which use hierarchical branching and selective loops to improve redundancy without the high cost of fully loopy architectures (Barthelemy, 2011).
Acyclic vs Cyclic Networks
While underground roots and primary branches follow an acyclic topology, many Ficus species develop aerial roots that descend and reconnect with the trunk or soil, forming loops. These reconnections transform the network from tree-like to cyclic.
When transport systems face damage or fluctuating loads, the optimal configuration shifts from treelike to loopy (Katifori, Szöllősi, & Magnasco, 2010). Loops function as redundancy mechanisms, preserving flow when a path fails. The banyan (Ficus benghalensis) exemplifies this principle: aerial roots anchor into soil and rejoin the system, redistributing both weight and fluid. Mathematically, loop formation increases the clustering coefficient

and reduces average path length, enhancing both connectivity and resilience (Barthelemy, 2011). Computational models of transport networks show the same transition, whereas load variability rises, loops self-organize to preserve flow efficiency (Fig. 2).
Mechanically, each loop distributes bending stress. Hydraulically, it ensures continuity under drought or injury. Studies of venation patterns confirm that redundancy prevents embolism and stabilizes flow (Sack et al., 2008; Zwieniecki et al., 2002). At the biochemical level, aerial roots extend this redundancy into communication. When they reconnect with the substrate, they create new exchange zones that reshape local chemistry and microbial activity. Root exudates such as organic acids, sugars, and signaling molecules mediate these interactions and continuously recon flow pathways (Robert et al., 2025; Walker et al., 2003).

Fig. 2. Panels A–D illustrate the modeled transition from acyclic to cyclic transport networks as load variability increases. Panel A shows an initially sparse, treelike configuration with minimal redundancy. As variability rises, B exhibits the spontaneous formation of the first loops, which shorten alternative paths and begin to distribute flow across multiple routes. Continued fluctuations produce the more interconnected geometry seen in C, where repeated reconnection events generate mid-scale cycles that stabilize transport. By D, the network has developed into a densely loopy structure capable of maintaining efficient flow despite local damage or fluctuating demand. This progression mirrors the behavior of aerial roots in Ficus benghalensis, in which reconnection and loop formation enhance both mechanical support and hydraulic resilience. (Adapted from Barthelemy, 2011).
Modeling of Nutrient and Signal Transport with Traversal Algorithms
Within this looping lattice, water, ions, and electrical signals move like data through a living network. Each node acts as a junction and each conduit as a wire, forming a biological circuit that adjusts dynamically to internal and environmental changes. Graph traversal algorithms help describe how these flows propagate throughout the Ficus system.
A breadth-first search (BFS) pattern mirrors how pressure waves travel through xylem, advancing layer by layer from trunk to leaf, ensuring that each tier of branches is hydrated before the next (Zwieniecki et al., 2002). Conversely, depth-first search (DFS) reflects localized signaling, where electrical and hormonal messages move along a single pathway to coordinate rapid responses to injury or light variation (Fromm & Lautner, 2007). These millivolt-scale signals transmit faster than chemical diffusion, functioning like a primitive nervous system encoded in sap.
In modeling studies, nutrient and signal transport can also be viewed through the lens of network optimization. Trees dynamically adjust vessel conductance to minimize energy loss while maintaining stable flow. In more complex, looped networks, the same principle applies to resilience: when a path is blocked, alternate routes automatically redistribute pressure and resources. Computational models of optimal transport networks show that introducing loops improves both flow continuity and energy efficiency under fluctuating conditions (Katifori et al., 2010). This explains why banyan trees evolve multiple aerial roots; they serve as natural bypasses that keep the system functional even under drought or physical damage.
At finer scales, root systems exhibit similar adaptability. Hydraulic architecture is tuned to balance flow stability and transport efficiency (Li et al., 2017), while root exudation regulates chemical exchanges that enhance nutrient availability (Robert et al., 2025). Together, these mechanisms allow Ficus networks to self-organize, maintaining function even as environmental inputs shift.
Viewed through this mathematical lens, the Ficus behaves as a biological algorithm, minimizing transport time, stabilizing flow, and preserving signal fidelity through structural loops and adaptive feedback. Each new root or reconnection effectively rewrites part of the system, improving its performance over time (Fig. 3).

Fig. 3. Log–log distributions of edge betweenness b for two transport architectures. (a), the Minimum Spanning Tree, shows a steep drop-off, meaning most flow is forced through a few critical paths. (b), the Optimal Traffic Tree, has a much shallower slope, indicating load is spread across many alternative routes. The x-axis shows betweenness values, and the y-axis gives their frequency. Networks with shallower slopes are more stable, efficient, and closer to the looped, adaptive behavior seen in Ficus systems (Barthelemy, 2011).
Allometric Scaling and Resource Optimization
Allometric Scaling Laws
In Ficus species, allometric scaling provides a guideline for understanding how structural and functional traits can evolve to maintain stability, efficiency, and adaptability. Allometry refers to how one biological dimension changes with another according to a power-law relationship.

Where the exponent β defines the scaling pattern (Fan et al., 2017). When β = 1, traits scale isometrically, meaning proportional growth; when β ≠ 1, traits grow disproportionately, showing some trade-offs in resource allocation.
Across 28 species of Ficus, leaf lamina area and mass coincide isometrically with stem area and mass (this is shown clearly in Fig. 4) (Fan et al., 2017). This suggests that as Ficus branches expand, investment in photosynthetic tissue remains proportional to support and transport tissue. However, petiole mass scales allometrically with lamina area, indicating that as leaves enlarge, additional biomass is allocated to the petiole to sustain mechanical support and hydraulic flow (Fan et al., 2017). These relationships reveal the balance between mechanical stability and energy acquisition, which is a central principle in Ficus evolution.

Fig. 4. Biplot of trait relationships based on multiple factor analysis (MFA) 11 stem/petiole (red) and 13 leaf traits (green) of 28 Ficus species. Some notable traits listed are Stem cross section area (SA), Vessel density (VD), Total leaf area (TLA), Saturated wood-water content (SWC), and Modulus of elasticity (MOE) (Fan et al., 2017).
Scaling relationships in Ficus also reveal strategic allocation patterns. Leaf number per stem mass (leafing intensity) decreases as leaf size increases, showing that trees with fewer, larger leaves use stems more intensively for support and transport. This adaptive scaling minimizes redundancy in leaf structure while maximizing the efficiency of carbon gain per stem investment. Furthermore, Ficus species vary widely in form, yet all maintain consistent allometric relationships that ensure energy balance and structural coherence. These findings confirm that scaling laws not only describe size relationships but also encapsulate functional design principles that have persisted throughout Ficus evolution (Fan et al., 2017).
Hydraulic Efficiency
Water transport efficiency lies at the core of Ficus physiology, dictating how trees sustain large canopies in tropical and subtropical climates. Hydraulic conductivity in Ficus stems scales from vessel diameter and fraction, but inversely with wood density and elastic modulus (Fan et al., 2017). This means species optimized for hydraulic performance often sacrifice mechanical stiffness. Large vessel diameters increase flow rate, yet they also heighten the risk of cavitation under water stress. The genus Ficus exemplifies how natural selection navigates this trade-off, achieving high water transport capacity without compromising resilience.
Vascular systems evolve toward fractal, space-filling designs that minimize resistance and energy loss (Savage et al., 2010). Ficus species mirror this pattern through their modular, highly redundant vessel networks, ensuring continuous water supply even if individual conduits fail. This redundancy allows rapid recovery after drought or mechanical injury, which is a crucial adaptation in fluctuating tropical environments.
In aerial species of Ficus, hydraulic efficiency is even more critical. Species such as F. benjamina and F. religiosa establish aerial roots that integrate into the main stem, forming a complex hydraulic grid. These roots function as additional water transport channels, enhancing both vertical and lateral conductance. The scaling of vessel elements within these roots follows a similar power-law relationship, linking diameter to root mass and length. By optimizing conduit geometry (Fig. 5), Ficus maintains steady hydraulic conductivity across growth stages, ensuring high photosynthetic productivity per biomass investment.

Fig. 5. Branching structures depicting the difference in internal network structure for Savage et al.’s ‘New model’ compared with the WBE model. Both models predict conduit taper, but the ‘New model’ also allows the number of conduits to increase and potentially fill a constant fraction of available wood area (Savage et al., 2010).
Mechanical Optimization
The mechanical structure of Ficus trees is a great example of optimization under competing hydraulic and gravitational constraints. While light, porous wood favors water transport; it reduces stiffness and strength. To counter this, Ficus species have evolved unique mechanical strategies that distribute stress efficiently. Their stems often feature dense peripheral wood and softer, water-rich cores, an arrangement that resists buckling while maintaining flexibility (Niklas & Spatz, 2006).
Many Ficus species also produce aerial and buttress roots that act as natural tension cables. In Ficus benghalensis, these roots extend from branches to the ground, transforming single-stemmed trees into multi-trunked colonies capable of spanning large areas. This structure redistributes mechanical load and increases wind resistance, which effectively lowers the mechanical stress per unit area of the stem. By spreading weight laterally rather than vertically, Ficus trees achieve large canopy spreads with minimal risk of toppling.
Mechanical scaling theory predicts that trees maintain a constant safety factor across size classes. Ficus follows this rule by adjusting wood density and stem geometry as it grows. Even as hydraulic efficiency declines with height, the slow but sure thickening of supportive tissues maintains an optimal balance between elasticity and rigidity. In essence, Ficus achieves mechanical homeostasis through a dynamic scaling process that uses structural reinforcement and physiological plasticity (McMahon & Kronauer, 1976).
Resource Distribution
Resource optimization integrates the physical and physiological aspects of Ficus design. Allometric relationships ensure that resource flows (like carbon, water, and nutrients) are distributed in proportion to structural demand. The near-isometric scaling of leaf and stem biomass indicates a coordinated allocation system, where photosynthetic and supportive tissues grow in tandem to sustain the tree's metabolic equilibrium (Fan et al., 2017).
Hydraulic and mechanical traits jointly shape this distribution of resources. High hydraulic conductivity enables intense leaf expansion and carbon fixation, while at the same time, mechanical reinforcement keeps that investment safe. The negative relationship between hydraulic efficiency and wood density implies that Ficus continuously adjusts its tissue composition to meet environmental pressures. In wetter habitats, low-density, high-conductivity wood is mostly found, and in drier regions, species favor denser wood with smaller vessels to prevent any unwanted cavitation (Fan et al., 2017). This variability in scaling demonstrates that resource allocation in Ficus is both genetically programmed and environmentally affected.
The branching architecture of Ficus also reflects efficient resource distribution. Fractal analysis of branching systems across tropical trees shows patterns that optimize both light interception and nutrient flow (Savage et al., 2010). Ficus crowns follow this idea, producing densely packed but organized canopies that balance exposure and shading. The result allows for consistent photosynthetic production. At the ecosystem level, resource optimization extends to many symbiotic relationships. Many Ficus species form relationships with fig wasps, which ensures year-round pollination. This reproductive strategy stabilizes carbon input and nutrient turnover, which in turn maintains the tree’s metabolic budget across seasons.
The study of scaling and resource optimization in Ficus reveals a finely tuned system of trade and compensation. Instead of following a single strict law, Ficus exhibits proportional patterns of investment between photosynthetic and supportive tissues, adjusts hydraulic efficiency through vessel redundancy, and strengthens mechanically through adaptive branching and root geometry. Together, these scaling patterns form an integrated growth strategy that supports large crowns, high productivity, and exceptional longevity, an evolved balance between structural cost and environmental demand.
Fractal Geometry of Ficus Crowns & Lindenmayer System Modeling
A fractal object with self-similarity shows that parts of an object look similar compared to the whole. Fractal patterns found in trees demonstrate approximate self-similarity, meaning that the branching patterns look similar but are not identical. Fractals show a set of repeated patterns or fragmented geometric shapes that are divided into smaller parts, similarly the tree branch looks like a miniature version of the tree, similar in pattern and form although not identical. The organization of branching patterns in trees, including Ficus, can be explained through fractal geometry which is molded with the Lindenmayer system (L-system).
The fractal growth the Ficus tree branches aims to generate a crown shape which enables the Ficus to better survive in its environment. The growth direction of the branches and the amount of foliage in each place in the tree crown is controlled by photomorphogenesis, the sensing of light, which forces a growth pattern which favors the highest collection of light while blocking light from competitors (Duchemin et al., 2018).
Lindenmayer Systems Modeling
L-systems are rule-based systems that can describe the natural branching patterns of trees. The L-system forms an object from an initial structure (axiom) and repeatedly replaces parts of it based on a set of rules called the production rules. Each round of replacement is known as an iteration. The more iterations we preform, the more complex the shape becomes, naturally forming a shape exhibiting fractal patterns (Hidayat et al., 2019).
The production rules used to model systems begin with the code Axiom (symbolized by ω)

where F represents the command “draw forward one segment” (segment 1 in Fig. 7). The branching pattern is formed using the production rule which defines how we will add new segments to existing ones.

Here, the symbol F, which creates the first branch, is replaced with two new branches: [ -F] indicates the modeling system to move forward (draw a segment) and rotate by the given angle to the left and [+F] draws a segment rotated to the right by the specific given angle. The square bracket [ symbol saves the current position while the bracket ] returns to the last saved position and angle. The formation of a branch using the product rule is shown below (Fig. 6). The angle of rotation parameter in L-systems controls the spread of branches, thus crown shape (Hidayat et al., 2019).

Figure 6: Fractal tree branch modeled with the L-system. In this system, the set angle of rotation is given as 𝛿 = 25 the system begins with Axiom ω : F and the production rule ω: F → [+F] [-F]. The first application of the production rule ω gives the pattern [+F] [-F] which creates branches 2 (associated with the [-F] rotation to the right) and branch 3 created from the [+F] command. The circled section represents what the branch looks like only with one application of the product rule (the first iteration) (Adapted from Hidayat et al., 2019).
Iteration rule cycles are represented by n, an integer that represents all real numbers. Where n=0 is the first cycle, meaning a simple branch. At each level of increasing n, the system grows by one level. For example, in the production rule:

Gives the results shown in the Fig. 7 with each iteration cycle n.
Table 1. Iteration cycles with their assocaited results following the product rule in equation 9.Each F is replaced by F[+F] [F-] in each step, creating a more complicated system at each level.
| Iteration (n) | Result |
|---|---|
| 0 | F |
| 1 | F[+F] [F-] |
| 2 | F[+F] [F-] [+F[+F] [F-]] [-F[+F] [F-]] |
An example of the complexity at increasing levels of iteration cycles are shown below (Fig. 8). (Hidayat et al., 2019).

Fig. 8. Fractal tree structure shown using L-system with 𝛿 = 25. With the production rule ω : FF[+F+FF] [-F-F] [+FF+F]. (Hidayat et al., 2019).
Trees, including the Ficus trees, develop fractal patterns to optimize their access to light and to occupy as much space as possible. For example, the branching pattern (above) exists in a 2-dimension plane, such that after a certainty amount of iteration cycles, the branches would overlap creating a less efficient system. However, to overcome this, tree can initiate new branches at a node that extend beyond the 2D plane and grow in the z axis (3D space).
To take the analysis of a branching system into 3D, we introduce three-dimensional vectors: H (heading) which represents the forward direction, L (left) which represents the lateral direction and U (up) which represents the vertical direction (Prusinkiewicz et al., 2019)
The following grammatical notations are introduced to the 3D L-system and are shown graphically below (Fig. 9):

Fig. 9. a) A graphical, 3-dimensional reprehension of Lindenmayer modeling with 3D L-system grammatical notation. b) an example of a branch formed in 3D space using L-system modeling with the fractal product rule F(2)[-F[-F]F]/(137.5)F(1.5)[-F]F. +/- = Turn left/right (around U axis), &/^ =Pitch down/pitch up (around L axis), \ / / = Roll left/roll right (around H axis) (Al-Rawi, 2022).
Fractal geometry patterns also arise in branching to ensure the efficiency of water flow in tree branches throughout all levels of branching. When a liquid flowing through tree branches encounters a sudden change in the size of the channel it flows through, such as when a branching point splits into several different smaller ones, there can be a backflow of the liquid. If the water does not flow smoothly, the tree wastes energy as turbulent waves resists the flow through the branches. Uneven and unproportional branching can cause inefficiencies in fluid transport and in nutrient distribution. To prevent a loss of energy in the tree, area-preserving branching ensures that fluid flow through the vascular system remains efficient across all levels of branching. A liquid will flow smoothly through a hierarchical network where the sum of the cross-sectional areas of smaller branches equals that of the parent branch. This design minimizes resistance and maintains a consistent flow of nutrients and water from trunk to leaves. Each successive branch decreases in radius by a constant factor √2, creating a self-similar, fractal structure that repeats throughout the canopy. This efficient geometric organization not only allows trees to distribute resources evenly but also helps regulate overlapping and spacing. The branches spread out to maximize coverage and minimize shading or crowding, ensuring optimal light capture and spatial balance. The branching pattern in plants is compared to the blood vessels of a mammalian heart which also form fractal patterns in their network (Fig. 10) (West, 2017, Chapter 9, pp.195-197).

Fig. 10. A comparison of mammalian artery and plant branch fractal patterns (West, 2017, Chapter 9, pp.195-197). .
Diffusion-Limited Aggregation (DLA) Modeling of Ficus Species
In Hong Kong's rugged terrain, an unexpected structural engineer stabilizes ancient stone retaining walls: the strangler fig (Fig. 11). This hemiepiphytic tree begins its life as a seed, sometimes deposited by a bird high in the crevice of a host tree or, in this case, a man-made stone structure. From there, it sends roots cascading downward, in a complex, searching pattern that can eventually envelop and consolidate its substrate (Jim, 2014).

Fig. 11. Strangler Fig root architecture on a stone wall in Hong Kong (Jim, 2014).
This growth is a biological form of reinforcement, and its fractal nature can be modeled by processes like Diffusion-Limited Aggregation (DLA). This model begins with a single stationary "seed" particle. New particles are then introduced and undergo a random walk (like Brownian motion) until they collide and stick to a growing cluster. This results in a dendritic structure (see Fig. 12 for the characteristic pattern) because the outermost branch tips are most likely to capture new particles, "shadowing" the inner regions from further growth. This growth instability is amplified by "tip-splitting," where a single tip divides to form new branches, producing a self-similar fractal pattern where the same branching motifs repeat at different scales (Amir et al., 2010).
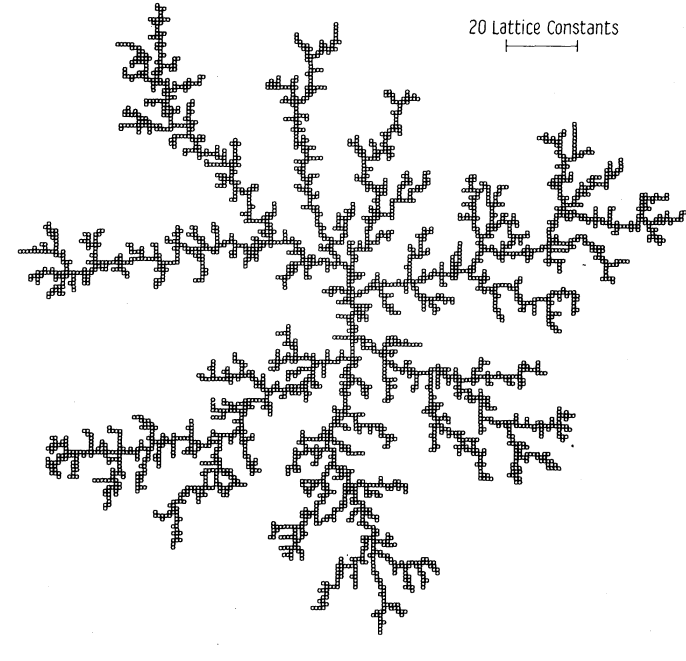
Fig. 12. Diffusion-limited aggregation (DLA) random aggregate of 3600 particles on a square lattice, showing the characteristic pattern (Adapted from Witten & Sander, 1981).
While DLA can effectively model the initial, exploratory growth of a strangler fig, the resulting structure is mechanically fragile. The full architectural complexity of Ficus species arises from secondary adaptations such as inosculation and aerial roots (Serrano Salazar et al., 2018). Inosculation, the natural fusion of adjacent roots and branches, creates a highly interconnected network within the trunk, providing exceptional mechanical stability. Simultaneously, aerial roots descend from branches to lignify into supportive "pseudo-trunks" upon reaching the ground. These pillars increase the tree's footprint and structural integrity, creating a collaborative system stabilized by multiple points of soil contact (Ludwig et al., 2019). Drawing inspiration from these biological strategies, Serrano Salazar and colleagues developed a biomimetic algorithm that augments a basic DLA model for constructing full-scale pipe-based structures. The "Rain Tree" installation (Fig. 13) exemplifies this approach, using standardized PVC bars and 3D-printed PLA knots to demonstrate the viability of this discrete, bio-inspired method for architectural assembly (Serrano Salazar et al., 2018).

Fig. 13. “Árbol de la lluvia” (Rain Tree) in front of the Faculty of Architecture at Medellín University. Biomimetic design inspired by trees, generated using a DLA-inspired algorithm (Serrano Salazar et al., 2018).
Their model was developed using a 3D Grasshopper visual programming tool. The algorithm begins by defining particles that originate at random positions on the upper face within a prism. These particles move downward at a constant velocity along a vertical trajectory. When a moving particle enters within a defined collision distance of a stationary (capturing) particle, it adheres, thereby extending the structure. Each captured particle then becomes a new capturing agent, further propagating the aggregation process (Serrano Salazar et al., 2018).
To simplify assembly and to keep the structure uniform, the system uses three types of knots – A, B, and C – which correspond to foundational (base of prism), bifurcating (fork between two branches), and connecting elements (inosculation and aerial roots), respectively (Fig. 14).

Fig. 14. Knot types used in the system: (A) foundational element (base of the prism), (B) bifurcating element (branch fork), and (C) the connecting element (inosculation and aerial roots) (Serrano Salazar et al., 2018).
Each bifurcation knot (type B) is associated with an aggregation ring – a conceptual circle derived from a cone whose vertex is the capturing particle and whose generatrix forms a fixed angle with the axis (Fig. 15). When a moving particle enters within the collision threshold of this ring, it is captured, and a new bar is generated. A symmetric mirror bar is also created, except in the case of type A knots, ensuring consistent bifurcation angles throughout the structure (Serrano Salazar et al., 2018).

Fig. 15. Geometric construction of type A and type B bifurcation knots. The diagrams illustrate how aggregation rings (dashed cones) are used to define the capture regions where new branches form. The vertex of each cone corresponds to the “capturing” particle, and its generatrix (length L) forms a fixed angle (β or δ) with the cone axis. When an approaching particle (open circle) enters within the collision threshold (≤ ε) of this cone, it becomes attached, creating a new bar (solid line). In a type A knot (top row), a single bar is generated upon capture. In contrast, a type B knot (bottom row) produces a symmetric twin bar, forming a bifurcation. This mechanism ensures that all bifurcations maintain consistent angular geometry throughout the structure (Serrano Salazar et al., 2018).
A key innovation in the algorithm is the incorporation of inosculation (bridges) and aerial roots, which introduces a stability mechanism. The geometric problem of connecting two non-adjacent bars via a bridge is solved by identifying a segment that forms the same angle with both parent bars. The distance (d) between the intersection planes and the segment is given by:
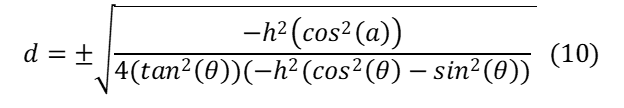
Where a is a fixed angle, and θ is the angle between the two bars. The figure below provides a sketch of the problem (Fig. 16).

Fig. 16. Geometric construction for bridge formation between non-adjacent bars. The diagram shows how the connecting segment (red) is defined to form the same angle (α) with both parent bars (black). The distance d between intersection planes and the segment depends on the bar angle θ, with h/2 = d·tan(θ). This setup underlies the algorithm’s modeling of inosculations and aerial root bridges (Serrano Salazar et al., 2018).
Only segments with lengths within a defined range are accepted, while those intersecting existing elements or terminating too close to existing knots are discarded. Similarly, aerial roots are generated by intersecting two conical surfaces: one centered on a branch and forming a fixed angle a, and another oriented vertically from the ground with angle β (Fig. 17). The intersection yields two symmetric segments, one of which is arbitrarily selected, provided its length falls within a specified valid range. This introduces new support points to the structure, enhancing its stability (Serrano Salazar et al., 2018).

Fig. 17. Generation of aerial roots through the intersection of two conical surfaces. The first cone (left) is centered on a branch and defined by angle α, while the second cone represents the vertical orientation from the ground with angle β. Their intersection (center) yields two symmetric candidate segments, one of which is selected if its length lies within the valid range (right) (Serrano Salazar et al., 2018).
To make sure the structure is physically possible, the algorithm includes a self-collision check. Any element that would intersect the ground or other parts is discarded. When multiple elements conflict at the same time, an incompatibility-counting algorithm removes the ones causing the most problems, ensuring the final structure has no overlaps. By repeatedly applying these rules, the algorithm builds a branched structure (Fig. 18) that grows more complex and stable, combining random growth with bio-inspired design (Serrano Salazar et al., 2018).

Fig. 18. Example of growth of the structure over 800 iterations (Serrano Salazar et al., 2018).
The management of Hong Kong's strangler figs is challenged by widespread misconceptions and inappropriate practices that compromise tree health. Unsympathetic repairs to retaining walls, such as using cement mortar to seal joints, block the micro-niches necessary for root growth, while aerial roots are often improperly cut. Construction, utility work, and misguided tree-care further damage the root systems, destabilizing the trees and negating their natural adaptations due to a lack of understanding of their mechanical value. Without dedicated conservation efforts, Hong Kong risks losing these iconic natural and cultural landmarks vital to urban biodiversity (Jim, 2014).
Perhaps a proactive approach to this issue could involve adapting a computational growth model, like the one by Serrano Salazar et al., to transform tree conservation. A specialized digital twin of a strangler fig would enable us to simulate its growth on a virtual stone wall and rapidly test interventions. Rather than waiting decades to observe a tree's response to a management change, we could model parameters like soil depth, irrigation, and joint designs to foresee outcomes almost instantly. This model-based approach provides a low-risk platform to virtually prototype support structures, determine the consequences of interventions, and discover effective ways to guide aerial roots – all before implementing any physical change.
Conclusion
The root and branch systems of Ficus trees embody the logic of graph theory, transforming biological structure into a living network optimized for flow, stability, and communication. Through both acyclic and cyclic configurations, Ficus integrates efficiency with resilience, forming loops that maintain transport even under stress. Its topology behaves like a self-correcting algorithm, continually adjusting pathways to sustain life and balance mechanical and hydraulic demands. In Ficus, allometric scaling and resource optimization represent an integration of biology, physics, and math. They have evolved to maintain hydraulic continuity, mechanical safety, and balanced resource distribution despite vast differences in size and habitat. From the vascular network’s fractal design to the coordinated scaling of leaf, stem, and root systems, every structural adjustment serves the same goal: maximizing efficiency per unit investment. These principles show how Ficus continues to be one of the most versatile and enduring plants in tropical ecosystems. The relationship between scaling laws and optimization not only explains its remarkable growth strategies but also the broader evolutionary ideas about how living systems adaptively manage constraints of energy, matter, and structure. Ficus trees such as the bayan tree form large crowns through the recursive growth of their branches, which follows a fractal geometry pattern. The self-similar patterns found throughout the crown and canopy are modeled by Lindenmayer systems which provide a mathematical model demonstrating that a fractal growth optimizes space, light capture and the efficient flow of liquids in Ficus trees. The Diffusion-Limited Aggregation model provides another useful framework for simulating the fractal root architecture of strangler figs, linking biological growth to computational design. By integrating mechanisms like inosculation and aerial roots, the model evolves from a fragile aggregation into a stable, adaptive structure. Applying such bio-inspired algorithms to conservation could help predict and guide fig growth, especially in areas like Hong Kong, supporting both ecological resilience and heritage preservation.
References
References
Al-Rawi, A. (2022). Generation of the Plants As a Self-Similarity Fractal In Three Dimensions Using Lindenmayer System. University of Anbar, 2(26), 88-94. https://doi.org/10.4206/aus.2019.n26.2.11.
Amir, S., Mohamed, N. S., & Hashim Ali, S. A. (2010). Simulation model of the fractal patterns in ionic conducting polymer films. Central European Journal of Physics, 8(1), 150-156. https://doi.org/10.2478/s11534-009-0036-6
Aumeeruddy-Thomas, Y., & Hossaert-McKey, M. (2024). Fig trees and humans: ficus ecology and mutualisms across cultures. Berghahn Books. https://search.ebscohost.com/login.aspx?direct=true&scope=site&db=nlebk&db=nlabk&AN=3636433
Barthelemy, M. (2011). Spatial networks. Physics Reports, 499(1–3), 1–101. https://doi.org/10.1016/j.physrep.2010.11.002
Brodribb, T. J., Skelton, R. P., Carriqui, M., Lucani, C. J., Bienaimé, D., & McAdam, S. A. M. (2023). Hydraulic design and drought tolerance in woody plants. Nature Ecology & Evolution, 7(9), 1383–1391. https://doi.org/10.1038/s41559-023-02180-z
Category: the great banyan. Wikimedia Commons. (n.d.). https://commons.wikimedia.org/wiki/Category:The_Great_Banyan
Duchemin, L., Eloy, C., Badel, E., & Moulia, B. (2018). Tree crowns grow into self-similar shapes controlled by gravity and light sensing. Journal of The Royal Society Interface, 15(142), 20170976. https://doi.org/10.1098/rsif.2017.0976
Fan, Z.-X., Sterck, F., Zhang, S.-B., Fu, P.-L., & Hao, G.-Y. (2017). Trade-off between stem hydraulic efficiency and mechanical strength affects leaf–stem allometry in 28 Ficus tree species. Frontiers in Plant Science, 8, 1619. https://doi.org/10.3389/fpls.2017.01619
Fromm, J., & Lautner, S. (2007). Electrical signals and their physiological significance in plants. Plant, Cell & Environment, 30(3), 249–257. https://doi.org/10.1111/j.1365-3040.2006.01614.x
Hidayat, E. W., Putra, I. K., Giriantari, I. A., & Sudarma, M. (2019). Visualization of a two-dimensional tree modeling using fractal based on L-System. IOP Conference Series: Materials Science and Engineering, 550(1), 012027. https://doi.org/10.1088/1757-899x/550/1/012027
Jim, C. Y. (2014). Ecology and conservation of strangler figs in urban wall habitats. Urban Ecosystems, 17(2), 405-426. https://doi.org/10.1007/s11252-013-0322-3
Katifori, E., Szöllősi, G. J., & Magnasco, M. O. (2010). Damage and fluctuations induce loops in optimal transport networks. Physical Review Letters, 104(4), 048704. https://doi.org/10.1103/PhysRevLett.104.048704
Li, S., Nie, Y., Zhou, X., & Zhang, X. (2017). Hydraulic architecture and adaptation of roots in tropical trees. Journal of Integrative Plant Biology, 59(9), 728–739. https://doi.org/10.1111/jipb.12534
Ludwig, F., Middleton, W., Gallenmüller, F., Rogers, P., & Speck, T. (2019). Living bridges using aerial roots of ficus elastica - an interdisciplinary perspective. Scientific reports, 9(1), 1-11. https://doi.org/10.1038/s41598-019-48652-w
McMahon, T. A., & Kronauer, R. E. (1976). Tree structures: Deducing the principle of mechanical design. Journal of Theoretical Biology, 59(2), 443–466. https://www.sciencedirect.com/science/article/pii/002251937690182X
Niklas, K. J., & Spatz, H.-C. (2006). Allometric theory and the mechanical stability of large trees. American Journal of Botany, 93(6), 824-828. https://doi.org/10.3732/ajb.93.6.824
Patrut, R. T., Garg, A., Patrut, A., Woodborne, S., Rakosy, L., Ratiu, I. A. (2023). Radiocarbon analysis of Indian banyan tree. Current Science 124(10):1175-1180. DOI: 10.18520/cs/v124/i10/1175-1180
Prusinkiewicz, P., Hammel, M., Hanan, J., & Mẽch, R. (1996). L-systems: From the theory to visual models of plants przem ysla W. https://algorithmicbotany.org/papers/l-sys.csiro96.pdf
Prusinkiewicz, P., & Lindenmayer, A. (1990). The algorithmic beauty of plants. Springer-Verlag. https://doi.org/10.1007/978-1-4613-8476-2
Robert, C. A. M., Himmighofen, P., McLaughlin, S., Cofer, T. M., Khan, S. A., Siffert, A., & Sasse, J. (2025). Environmental and biological drivers of root exudation. Annual Review of Plant Biology, 76, 317–339. https://doi.org/10.1146/annurev-arplant-083123-082752
Runions, A., Lane, B., & Prusinkiewicz, P. (2007). Modeling trees with a space colonization algorithm. ACM SIGGRAPH 2007 Sketches, Article 117. https://doi.org/10.1145/1278780.1278940
Sack, L., Dietrich, E. M., Streeter, C. M., Sanchez-Gomez, D., & Holbrook, N. M. (2008). Leaf hydraulic conductance and venation architecture in tropical rainforest trees. Proceedings of the National Academy of Sciences, 105(5), 1567–1572. https://doi.org/10.1073/pnas.0804294105
Savage, V. M., Donoghue, M. J., Mills, H. M., & Loreau, M. (2010). Hydraulic trade-offs and space-filling enable better fitness in tree vascular networks. Proceedings of the National Academy of Sciences, 107(52), 22769–22774. https://doi.org/10.1073/pnas.1012194108
Serrano Salazar, S., Carrasco Hortal, J., Morales Menárguez, F., Pablo, J., & Salazar, G. (2018). Cooperative Trees by Adding Inosculated and Discrete Definitions to a DLA Design. https://papers.cumincad.org/data/works/att/ecaade2018_393.pdf
Sharma, A., & Tiwari, S. (2017). Plant growth modeling using the L-system approach and its visualization. International Journal of Computer Applications, 160(4), 1–5. https://doi.org/10.5120/ijca2017913124
Walker, T. S., Bais, H. P., Grotewold, E., & Vivanco, J. M. (2003). Root exudation and rhizosphere biology. Plant Physiology, 132(1), 44–51. https://doi.org/10.1104/pp.102.019661
West, G. B. (2017). Scale: the universal laws of growth, innovation, sustainability, and the pace of life in organisms, cities, economies, and companies. Penguin Press. http://search.ebscohost.com/login.aspx?direct=true&scope=site&db=nlebk&…
Witten, T. A., & Sander, L. M. (1981). Diffusion-Limited Aggregation, a Kinetic Critical Phenomenon. Physical Review Letters, 47(19), 1400-1403. https://doi.org/10.1103/PhysRevLett.47.1400
Zwieniecki, M. A., Melcher, P. J., & Holbrook, N. M. (2002). Hydraulic design of leaves: Efficiency and safety of the water transport system in plants. Plant, Cell & Environment, 25(10), 1445–1453. https://doi.org/10.1046/j.1365-3040.2002.00917.x