
Table of Contents
Keywords: Mathematical modelling, leaf area, pipe model theory, finite element method (FEM), stress distribution, chestnut tree hub, biotic-abiotic-movement (BAM) model.
Abstract
Chestnut trees (Castanea) reveal complex biological and ecological patterns that can be analyzed through mathematical and computational modelling. This paper explores different modelling techniques used to better understand and predict chestnut species’ behavior. Models based on linear relationships, such as the Pipe Model, allow for estimations of leaf area, as well as explaining their variability within an individual. Chestnut’s shell breaking mechanism can be simulated using Finite Element Modelling (FEM), revealing how birds, like woodpeckers, reposition chestnuts in their beak to maximize efficiency, without damaging their beak. Additionally, chestnut trees, which are a dominant species in a certain region, can be represented through scale-free networks. Chestnuts with large crowns act as network hubs and follow the power-law distribution to a certain extent. This was seen during the chestnut blight in the 1900s, where their attack had destabilized the ecosystem, which led to fluctuations in the rodent and rattlesnake reproductive cycles. Finally, the Biotic-Abiotic-Movement (BAM) framework helps better understand and predict chestnut species distribution across the globe by identifying locations where biotic and abiotic conditions promote growth and survival of chestnut trees.
Introduction
Chestnut trees, belonging to the genus Castanea, are part of the Fagaceae family (Pinto et al., 2020). This family is mostly a monoecious group of plant that have simple leaves, small unisexual flowers, and nuts enclosed in a valved cupule (Fig. 1) (Simpson, 2010).

Fig. 1. Chestnuts from different Castanea species inside a valved cupule, an outer shell with spikes that surrounds and protects the nut (Massantini et al., 2021).
Chestnut production has gradually increased over the years because of their durable wood and edible fruit. Their cultivation dates to the ancient Greece for the same reasons. Today, the majority of chestnut are grown across a wide range of climates due their high generic diversity (Massantini et al., 2021).
(see Chestnut Physics and Chestnut Chemistry for more background information)
Computational modelling allows researchers to study complex biological systems. These models are used to test hypotheses, provide new insights, deepen understanding, and explore how different factors influence one another. They do not replace experiments, but are used to demonstrate whether the proposed mechanism can lead to an observed outcome (Brodland, 2015). Another approach, mathematical modelling, uses mathematical concepts to represent the relationship between variables and parameters (Green, 1992). In other words, modelling is used to replicate the behavior of complex systems to improve understanding and to predict their behaviour (Hardman & Ross, 2006).
In this essay, both modelling techniques are applied to have a better understanding of chestnut’s crown structure, shell shape, and its distribution in the world. By applying these models, biological observations, such as chestnut’s morphology, can be linked to mechanical and ecological functions.
Seed-Breaking Mechanism Modelled by FEM
Small mammals and birds play a critical role in the growth of the chestnut population through their mutualistic relationship with the tree. The lack of tannins in the chestnut creates a palatable taste, attracting animals near the tree to pick the fallen nuts off the ground and carry them to neighbouring areas. When a mammal buries a nut or a bird drops it while in flight, the nut can germinate and grow in a new region. Birds play a vital role in this distribution mechanism. Many species, such as woodpeckers and blue jays, prefer chestnuts to other nuts because the smaller, flattened shape of the chestnut shell makes it easier to hold. However, the convenience of retrieving and transporting the chestnut is insignificant if it is too difficult to break it open and retrieve the edible kernel (Wright et al., 2022). (see Chestnut Physics for a discussion on mutualism)
Using finite element analysis, Yang and Qi conducted a study to determine the simplest method for opening a chestnut shell (Qi & Yang, 2021). The finite element method (FEM) is a numerical technique used to simply complex problems, frequently modelled by partial differential equations, to solve for approximate solutions. These simple elements can be triangles, tetrahedra, or other common shapes. The method is often used in engineering to analyze how irregular structures respond to forces, because the simpler elements can be analyzed by classical laws of physics. Since the chestnut shell has a non-uniform curvature and varying thickness, FEM helps predict where cracks will occur (El-Amin, 2023).
A solid model of the chestnut was created using Ansys software, a simulation software used to analyze how structures will respond to forces without having a physical prototype. The shape of the chestnut is irregular and can generally be approximated as a spherical shape, a hemispherical shape, or a pancake shape. As more than 80% of chestnuts are hemispherical with a pointed tip along the circumference of the circle (Fig. 2), this shape was chosen for the model (Yuan et al., 2013). The chestnut model was analyzed on a Cartesian plane (Fig. 3), where the x-axis pointed from one side of the flat face to the other, the y-axis pointed along the sharp tip of the chestnut, and the z-axis pointed from front to back (Qi & Yang, 2021).

Fig. 2. Pile of chestnuts with the most common hemispherical shape. The chestnuts have a flat face on one side and a curved surface on the other. The circumference of the flat face is called the shell edge. The shape differs from a perfect hemisphere by its sharp tip, where the chestnut attaches to the tree. The chestnuts grow from the tree in a burr, shown at the top of the picture, which contains up to three chestnuts and is much easier to open than the chestnut itself (Vliet, 2004).

Fig. 3. Diagram of the chestnut model. The selected shape was a smooth hemisphere with a sharp tip at the bottom. A) Aerial view of chestnut model, with the flat face resting on the surface. The x-axis of the chestnut is horizontal on the flat face. The y-axis pointed from the top of the chestnut down to the sharp tip. B) Side view of the chestnut model. The z-axis was chosen to point from the flat face at the front to the rounded curve along the back. The x-y plane was the flat face of the chestnut (Qi & Yang, 2021).
The Ansys model was based on the average physical parameters, specifically the elastic modulus and Poisson’s ratio, and geometric dimensions of 100 Castanea mollissima samples, a type of Chinese chestnut (Qi & Yang, 2021). The elastic modulus measures the stress required to deform a material, in which a higher modulus indicates a stiffer material. The experimental results for this parameter in the X, Y, and Z directions were 900 MPa, 680 MPa, and 1200 MPa, respectively. Since the shell is mainly composed of cellulose and hemicellulose, which resist deformation under stress, these moduli are relatively high, with the z-direction being the stiffest. Poisson’s ratio (ν) is a dimensionless property describing a material’s tendency to deform in directions perpendicular to the applied force. It is calculated by the negative ratio of transverse strain to axial strain, where transverse and axial are the two directions perpendicular to the applied force, as seen in Equation 1 (Belyadi et al., 2017):

For example, if the force was applied downwards in the z-direction, the transverse strain would be measured along the x-axis and the axial strain would be measured along the y-axis. A higher Poisson’s ratio means it has a large deformation perpendicular to the applied force (Belyadi et al., 2017). It is commonly between 0 and 0.5 for most materials, with the chestnut shell having a measured ratio of 0.30 in all three directions. This means the ideal breaking mechanism will primarily depend on elastic modulus, as the Poisson’s ratio is uniform across the shell (Qi & Yang, 2021).
The breaking mechanism was tested in each direction using the Ansys model to determine the optimal method for opening the chestnut. To test the x-direction, a 500 N load was applied to one side (Fig. 4). The shell deformed inward until it cracked cleanly in the y-direction. The highest stress occurred around the area where the load was applied and along the y-z plane (Fig. 5). This occurred because the chestnut’s natural fibres ran parallel to the y-axis and the stress spread evenly across the grain, eventually creating a clean crack between fibres once the stress became strong enough. To test the cracking in the y-direction, the bottom tip was constrained, and a downward force of 500 N was applied to the top of the chestnut. The top compressed inward, and the stress ran down along the fibres, intersecting at the sharp tip. Since the tip is thin and constrained, the strain is concentrated at the bottom, and the tip cracked first. This created small, irregular cracks shooting upwards from the bottom, which is suboptimal for opening the nut. The z-direction was tested by constraining the flat face (the x-y plane) and applying the force from the back of the shell (the center of the round side of the hemisphere). The flatter surface created a larger contact area, and the stress spread evenly along the flat face, resisting deformation until the stress grew too high and an abrupt crack formed. This was expected due to the higher elastic modulus in the z-direction. The ideal mechanism for cracking the shell is by applying a force to the side (in the x-direction), which creates a clean crack along the grain of the chestnut. The other directions are both inefficient, as the y-direction only broke at the tip, and the z-direction created an abrupt, unpleasant crack (Qi & Yang, 2021).

Fig. 4. To test the breaking mechanism in the x-direction, a 500 N force is applied to one side of the chestnut, parallel to the x-axis (Adapted from Qi & Yang, 2021).

Fig. 5. Nephogram of stress distribution in the chestnut. Since the chestnut is symmetrical, half of the hemisphere is shown. A) Nephogram of stress after a force is applied in the x-direction. The 500 N force is applied to the side of the chestnut, called the contact area (top right), and the greatest stress is seen in the contact area and at the center of the chestnut along the y-z plane. The stress concentrates along the edges of the plane, parallel to the fibers, and a clean crack forms between the fibers in the y-direction. B) Nephogram of stress after a force is applied in the y-direction. The greatest stress occurs at the contact area, but it also concentrates at the sharp tip at the bottom. Since the tip is thin and constrained, it cracks first. C) Nephogram of stress after a force is applied in the z-direction. The greatest stress occurs at the contact area and at the flat face (x-y plane). The stress is evenly distributed and creates an abrupt, irregular crack in the flat surface (Adapted from Qi & Yang, 2021).
An efficient mechanism for opening the shell is vital to the mutualistic relationship between birds and the chestnut tree, as the nut can only germinate in new regions if the animal is willing to retrieve the chestnut with certainty that it can access the edible kernel inside. Woodpeckers, a known consumer of American chestnuts, will reposition shells into an ideal position before trying to open them with their beaks. They have evolved this behaviour to increase efficiency and protect their beaks. By breaking the chestnut from side to side, the woodpeckers can easily retrieve the edible kernel in one piece, increasing the likelihood that the birds will select a chestnut over another seed or nut in the forest (Yi et al., 2014).
Mathematical Modelling of Crown Structure and Growth in Chestnut
The architecture and growth dynamics of the chestnut crown can be quantitatively described through a series of mathematical models that relate key structural and physiological variables. Trees have evolved to express a range of phenotypic characteristics and behaviours, allowing them to succeed under a range of environmental conditions. Models aid in studying and understanding aspects such as resource allocation and growth patterns for scientific, commercial and preservation purposes, but the multitude of characteristics a given chestnut tree can display means that simpler models, often built under ideal conditions, are unable to provide a general reproduction applicable to most individuals of a given species.
Leaf Area Estimation
Leaf area is an important characteristic correlated to physical and metabolic factors of chestnut trees, including, but not limited to, photosynthetic capacity (see Chestnut Chemistry). Chestnut trees adjust their leaf dimensions according to the amount of sunlight they receive. In well-lit environments, leaves are larger and thicker due to the abundance of energy. Even though leaf area changes from leaf to leaf, they have a growth pattern that can be estimated by Equation 2 (Serdar & Demirsoy, 2006):

Where AL is the leaf area (cm2), L is the leaf length (cm), and W is the leaf width (cm) measured at the midpoint of the lamina (Fig. 6).

Fig. 6. Chestnut leaf displaying the Width (W) and Length (L) measurements used to estimate leaf area (Serdar & Demirsoy, 2006).
Leaf area is an important indicator of the plant’s nutrition and is directly related to its need to be connected to other parts of the tree, as described by the Pipe Model.
The Pipe Model
According to the pipe model theory (PMT), a fixed quantity of leaves is supplied by a corresponding section of non-photosynthetic tissue that has a uniform cross-sectional area. The cross-sectional area of the sapwood (AS) in a tree’s stem is proportional to the cumulative leaf area (AL) it supports. This concept views each unit of leaves as being connected to the stem by a "pipe" of constant cross-sectional area, which serves as a functional link for transport and support (Shinozaki et al., 1964).
Chestnuts tend to follow this postulate within a single branch, exhibiting a strong linear correlation; however, they show a significant deviation from the strict pipe model when considering the entire tree. The AL:AS ratio was found to decrease with increasing branch height, which is a necessary sacrifice the tree has to make due to increased gravitational pull on the sap as the xylems stretch further away from the root. A generalized linear mixed model identified branch height as the main explanatory variable for this intra-tree variability. The most parsimonious model describing this relationship is given by Equation 3 (Gehring et al., 2015):
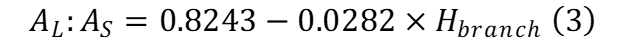
Where Hbranch is the height of the branch insertion in meters. This indicates that for every 10-meter increase in height, the AL:AS ratio decreases by approximately 0.282 units. To enable comparisons between trees without the confounding effect of sampling height, the concept of AL:AS (ground), the theoretical ratio at ground level can be calculated with Equation 4:

This is observed as a consequence of resource optimization. The more light the leaves have access to, the more energy they can produce by themselves, and the less they need to rely on getting energy from other parts of the plant. For this reason, not only do leaves at the top have a smaller area, but they grow more massive with their increased photosynthetic capabilities, and the tree can grow to great heights without needing to divert much of its energy to far-away tips (Joesting et al., 2009).
Adaptation of Chestnut Trees to Their Ecosystems
A Hub in a Network
American chestnuts, a historical species in North America, once played a major biological role in forests, as they used to dominate 80 million hectares from Maine to Mississippi (Fei et al., 2012). As a dominant tree species with a positive neighborhood effect, they helped establish a dynamic equilibrium within their ecosystems, a constant dance balancing the structural arrangement of the forest, species composition and species interaction within a given disturbance range (Frelich, 2016). Chestnut trees exert a positive influence on their environments through multiple pathways: by producing nutrient-rich nuts, a valuable energy source for birds and mammals, by developing a dense canopy that provides habitat for wildlife and by growing deep roots that maintain soil structure and fertility (Kroll, 2023). As a foundation species, the chestnut tree provides physical structure to its ecosystem, shaping and maintaining niches and interactions, in contrast to a keystone species, which regulates biodiversity through a disproportionate impact relative to its abundance (Davila, 2025).
Recent studies have applied the mathematical concept of networks to tropical rainforests, revealing that dominant plant species can exhibit scale-free interactions within local clusters (Ball, 2024). Scale-free networks are characterized by a few nodes with high connectivity (hubs) and many nodes with low connectivity (Beiler et al., 2010). This framework can reasonably be extrapolated to the role of American chestnuts within their forest communities, modelling the tree as a hub, and its multiple interactions with other species as edges. Characterizing chestnut trees as hubs is supported by the observation that trees with larger crown areas tend to have larger interaction zones (Schmid et al., 2020). Scale-free networks usually obey a power law distribution (Franceschet, n.d.), as seen in equation 5:

Where k represents the number of edges connected to a node, P(k) represents the probability of a randomly chosen node to have a degree k, and y is a constant parameter of the distribution.
However, natural systems rarely obey theoretical principles perfectly. Forest networks deviate from this idealized law. Analyses of forest networks revealed that node degree is better summarized by this equation (Schmid et al., 2020):

Where <k> is the average number of species a tree connects to, ki is the number of edges connected to a node i, N is the number of nodes in the network, and E is the number of edges in the network.
This relationship imposes a natural limit N to the series, reflecting the total number of nodes in the network, while the factor of two accounts for the concept of undirected networks, in which species have mutual interactions (Schmid et al., 2020) (Fig. 7). Although this equation does not explicitly describe the distribution of nodes by their connectivity, it implies that the system must contain a few highly connected nodes and many low-connected ones with low connectivity to maintain a constant average degree.

Fig. 7. Scale-free network model. The American chestnut, a dominant species, can be modelled as a hub (grey node), as it maintains multiple interactions with species in its surrounding (Seo et al., 2013).
Self-organization of an ecosystem around these scale-free mechanisms could enhance its robustness (Ball, 2024). Indeed, the heterogeneous architecture characteristic of scale-free networks enables dynamical robustness, defined as the capacity of a system to maintain a level of structural integrity and functioning under deliberate attacks, which target hubs, and random attacks. Scale-free networks are particularly resistant to random attacks, as most nodes have low connections, but are deeply affected by targeted attacks, as hubs maintain disproportionately a lot of connectivity (Cai, 2021).
According to this model, chestnut trees could benefit from the robustness of the system, as random natural perturbations are less likely to strongly affect the tree’s surrounding community. By maintaining stable dynamics within a cluster, the chestnut tree can rely on consistent nutrient cycling and symbiotic partners. Furthermore, numerically dominant species can influence the establishment of new species while ensuring their own survival, which represents an important competitive advantage (Gilbert et al., 2009). For instance, with its large crown area and its dense distribution, chestnut trees can regulate the amount of light passing through their canopies, creating the partially shaded environment their seedlings need to establish effectively (Government of Canada, 2018). Moreover, by being able to have a dense distribution, the species maximizes the availability of compatible chestnut trees for reproduction (Bickerton, 2019).
As mentioned above, scale-free networks are particularly vulnerable to targeted attacks, which can profoundly impact ecosystem stability. In the 1900s, when the causal agent of the chestnut blight, Cryphonectria parasitica, nearly eradicated American chestnuts, key connections maintained by this hub were disrupted. In the past few years, biologists have observed irregular birth rates in timber rattlesnakes, a species with energetically demanding reproductive cycles spaced across several years. Investigations into this irregularity revealed that the disappearance of many American chestnuts was indirectly responsible. Timber rattlesnakes typically feed on mice or other rodents, which themselves rely on nuts for food. American chestnuts historically produced large annual crops, supporting a relatively stable population of rodents. However, following the blight, rodents became dependent on the periodic pulses of crops produced by oaks, beeches or hickories, causing their population to fluctuate dramatically from year to year. Consequently, timber rattlesnakes have reduced their reproductive cycles, as they don’t have enough energy to maintain their previous rhythm, further amplifying the central role of chestnut trees among their ecosystems (Briggs, 2024).
Distribution Across the World
The spatial distribution of chestnut trees can be described mathematically as a function of biotic factors (B), abiotic factors (A) and movement factors (M). Biotic factors describe interactions with living organisms, abiotic factors refer to non-living environmental conditions, and movement factors highlight the tree’s opportunity to spread to new locations (Fei et al., 2012). Biologists use mainly the Biotic-Abiotic-Movement (BAM) framework to represent a species’ area of distribution. The niche occupied by the species corresponds to the intersection of these three factors (Fig. 8) (Soberón & Osorio-Olvera, 2023):


Fig. 8. Illustration of a BAM framework. The cross-hatched area, situated at the intersection of biotic factors, abiotic factors and movement factors, represents an actual area occupied by the species. The dotted area is situated at the intersection of only 2 factors, therefore representing a potentially habitable area (Soberón & Osorio-Olvera, 2023).
When projecting a geographical region through time, this theoretical principle can be used to create a realistic framework based on dispersal capacities and historical initial conditions describing the area of distribution of species j, as modelled by this general model (Soberón & Osorio-Olvera, 2023):

This function enables researchers to represent a geographical distribution of species over time, modelled by a grid of n cells forming a geographic plane. Typically, columns correspond to latitude coordinates, while rows correspond to longitude coordinates. A binary scheme is used; each cell indicates “0” if the area is unsuitable or “1” if the area is suitable.
In this expression, Gj(t+1) and Gj(t) are vectors of binary values, indicating with a “0” or a “1” if a cell is occupied or not. The argument (t+1) denotes the subsequent time step, illustrating how occupied areas can dynamically evolve depending on biotic, abiotic and movement factors. If, over time, any matrix equals 0, the region can no longer be occupied by the species, further emphasizing the correlation between the three factors determining spatial distribution. Bj(t) and Aj(t)are diagonal matrices, where a diagonal value of “1” denotes, respectively, a favorable biotic and abiotic environment for the species j, while a value of “0” denotes unsuitable conditions. Mj is an adjacency matrix n x n expressing the potential dispersal between cells, depending on the theoretical capacity of the species j to colonize adjacent areas. This matrix remains constant over time, as it reflects the fixed special configuration of landscapes and the dispersal ability of species (Fig. 9) (Soberón & Osorio-Olvera, 2023).

Fig. 9. Application of the function used to model a geographical region through time to a simplified hypothetical scenario. A) Current distribution of a hypothetical species established in Canada. The species occupied the areas delimited by the cells, from left to right, 1 and 5. B) Predicted distribution of a hypothetical species at time t. The species now occupies the areas delimited by the cells, from left to right, 1, 2, 5 and 8. C) Matrices used to project the distribution of the hypothetical species at time t. Each matrix is labelled with cx, indicating what rows and columns refer to (Camille Lebourg’s own artwork).
While a habitable niche must satisfy all three factors, climatic variables, a key element of abiotic factors, are considered first-order constraints, as they define the border area where a species can survive. These climatic parameters can be divided into three main classes: thermal variables, which limit growth through growing-season warmth and winter coldness; moisture variables, which describe the spatial and temporal availability of water through precipitation and moisture; and variability indices, which define temperature fluctuations in a given time (Fei et al., 2012).
By analyzing the occupied area of each chestnut species in relation to these parameters, it has been found that chestnut species share similar geographic distributions and climatic limits, growing in moist and mild forests at comparable longitudinal spans and distances from coastlines. Specific-species design solutions enable chestnut trees to persist within their specific environments, exhibiting resistance to distinct thermal and moisture gradients. For instance, European chestnuts tolerate colder and drier regions, as the Mediterranean Sea acts as a dispersal barrier, restricting their area of distribution to higher latitudes. In contrast, Japanese chestnut occupies a region with higher moisture availability, reflecting the abundant precipitation characteristic of Japanese islands (Fig. 10) (Fei et al., 2012).

Fig. 10. Graphical representation of the primary distribution of different species of chestnut trees, highlighting their tolerance to thermal climate and moisture. The horizontal axis indicates the thermal climate gradient, from cold to warm. The vertical axis indicates the moisture gradient from wet to dry (Fei et al., 2012).
Furthermore, the global distribution of chestnut trees across the world is not random; it reflects a selective occupation of environments that maximize their growth and survival (Fig. 11). The suitability of a site for chestnut trees is influenced by soil properties. Optimal growth occurs in well-drained soils with a pH between 5.5 and 6.5. More acidic soils can burn young shoots and leaves, compromising long-term survival, while more basic soils limit growth by their poor nutrient quality. Moreover, effective soil drainage ensures the renewal of essential nutrients (Fulbright, 2012).

Fig. 11 Global distribution of chestnut trees, which are found in regions with favorable soils and pH, as shown across three maps. A) Distribution of chestnut species across the world. American, European and Japanese chestnuts are distributed approximately from 30 to 50 °N, while Chinese chestnuts are distributed approximately from 15 to 40 °N (Fei et al., 2012). B) Soil pH across the world. Chestnut trees grow in soil with a pH between 5.5 and 6.5. In this global map, it corresponds to red-purple pixels (Cohen, 2016). C) Soil distribution across the world. Chestnut trees grow in well-drained soil, corresponding to sandy loam (number 2, brown) or loam soils (number 4, light pink) (Koirala, n.d.).
Impacts of Climate Change
Climate is an ever-changing natural condition whose mutability has increased exponentially with human activity since the Industrial Revolution. Chestnut trees have spread around the world and settled in areas where the established BAM framework factors are optimal, meaning the current-day chestnuts have built their survival toolkit upon design solutions for current-day challenges. Climate change is violently reshaping this map, especially through major changes in abiotic factors, pushing the species’ optimization to their limits. To illustrate, sweet chestnut trees have optimal living parameters that include: an annual temperature mean of 8-15 °C, yearly precipitation of 600-1600 mm, and chilling accumulation of above 90 chilling portions per winter for proper budburst, flowering, fruit set, and maturation. They are unable to withstand minimum temperatures below -16 °C, suffer thermoinhibition above 32 °C, and are severely constrained by droughts longer than two months. These abiotic factors are first-order constraints, and with projections for the Mediterranean basin indicating warmer temperatures, longer and more frequent droughts (Fig. 12), and reduced winter chilling, the design solutions chestnuts currently employ will soon become maladaptive. This increased environmental pressure could catalyze either the rise of new breeds more tolerant to surging environmental parameters or their extinction (Freitas et al., 2021).

Fig. 12. Projected drought frequency (top row) and drought intensity (bottom row) for the period 2021-2060 under the worst shared socioeconomic pathways under a study by Essa (adapted from Essa et al., 2023).
It is important to highlight that the optimal BAM framework for chestnut trees’ survivability is unlikely to disappear, but it will shift geographically towards the north, due to areas currently within the optimal temperature range becoming too hot and areas too cold for chestnut growth now attaining ideal temperatures. For the American chestnut, Figure 13 displays some high-emission scenarios of up to 100% catastrophic loss of suitable habitat, accompanied by a northeastern range shift of 476.9 km in the BAM framework (Adeyemo & Granger, 2023).

Fig. 13 American chestnut habitat suitability model and multiple predictions of habitat range shift based on different high-emission models and scenarios (Adeyemo & Granger, 2023).
Conclusion
The chestnut trees’ leaf growth follows patterns to maximize resource distribution and energetic equilibrium. Leaf area distribution patterns can be reliably approximated using linear parameters of length and width. The ratio of leaf area to sap area remains constant within a single branch, but linearly decreases as the branch’s height increases, due to the distance from the roots and light availability.
Chestnut trees show impressive integration of mechanical adaptation and ecological function. Finite element modelling (FEM) was used to examine how chestnut’s irregular, non-uniform curvature and variable thickness shape responds to forces applied in different directions. The shell was seen to break cleanly when force is applied in the x-direction due to the alignment of the cellulose and hemicellulose fibers. When force is applied parallel to these fibers, the shell resists stress and cracks irregularly and abruptly. Woodpeckers appear to understand this mechanism when breaking the nut. They reposition the chestnut in their beaks to apply pressure from the sides of the chestnut, producing a clean cut along the grains without damaging their beaks. This illustrates the mutualistic relationship of chestnut trees and seed-hoarders that support seed dispersal.
Chestnut trees also have an important role in their environment by producing nutrient-rich nuts for birds and rodents, forming a dense canopy that provides shelter for wildlife, and developing deep roots that maintain soil fertility and structure. In areas where they are dominant, chestnuts with higher crowns act as hubs in scale-free networks. That means that disturbances targeting these hubs have devastating effects on the ecosystem. For instance, in the 1900s, the chestnut blight impacted several chestnut trees, which triggered cascading events on the rodent and rattlesnake population.
BAM modelling and matrix representation have also helped researchers understand and predict chestnut’s species distribution by identifying favourable and unsuitable biotic and abiotic conditions. Their global distribution is not random, but selective to favourable environments that maximize their growth and survival. Although chestnut species grow in similar mild and moist forest regions at comparable distances from the coastline, each has evolved unique design solutions to persist in environments with different thermal and moisture gradients. For example, European chestnuts tolerate colder and drier regions, while Japanese chestnuts are well adapted to regions with high moisture. Unfortunately, climate change is altering the current BAM framework to the point where up to 100% of the habitats of some chestnut species may be lost, due mainly to abiotic factor shifts such as rising temperatures.
Overall, computational and mathematical modelling helps deepen the understanding of chestnut tree species.
References
References
Ball, P. (2024). Uncovering Networks in Rainforest Plants. Physics, 17. https://doi.org/10.1103/Physics.17.68
Beiler, K. J., Durall, D. M., Simard, S. W., Maxwell, S. A., & Kretzer, A. M. (2010). Architecture of the Wood-Wide Web: Rhizopogon spp. Genets Link Multiple Douglas-Fir Cohorts. The New Phytologist, 185(2), 543-553.
Belyadi, H., Fathi, E., & Belyadi, F. (2017). Chapter Thirteen - Rock Mechanical Properties and In Situ Stresses. In H. Belyadi, E. Fathi, & F. Belyadi (Eds.), Hydraulic Fracturing in Unconventional Reservoirs (pp. 207-224). Gulf Professional Publishing. https://doi.org/https://doi.org/10.1016/B978-0-12-849871-2.00013-7
Bickerton, H., McConnel, A., Holmes, K., Archambault, M.C., Voisin, L., Mannion, J., Smith, M., Laurent, K., deCatanzaro, R., Dunn, L., Brondex, V., Brownell, V., Wheeldon, A., Snyder, E., Collins, M., Jacobs, C. (2019). Recovery strategy for the American chestnut (Castanea dentata) in Canada. Environment and Climate Change Canada. http://epe.lac-bac.gc.ca/100/201/301/weekly_acquisitions_list-ef/2019/1…
Briggs, K. (2024). How the Loss of American Chestnuts Impacts Timber Rattlesnakes Today. https://www.oriannesociety.org/faces-of-the-forest/loss-of-american-che…
Brodland, G. W. (2015). How computational models can help unlock biological systems. Seminars in Cell & Developmental Biology, 47-48, 62-73. https://doi.org/https://doi.org/10.1016/j.semcdb.2015.07.001
Cai, M., Liu, J., Cui, Y. (2021). Network robustness analysis based on maximum flow. Frontiers in Physics, 9. https://doi.org/https://doi.org/10.3389/fphy.2021.792410
Cohen, J. (2016). Researchers create global map of soil pH and illuminate how it changes between wet and dry climates. https://phys.org/news/2016-12-global-soil-ph-illuminate-climates.html
Davila, C. M. (2025). Foundation Species: Nature's Hidden Architects Shaping Life Itself. https://www.wildlifenomads.com/blog/what-is-a-foundation-species/
El-Amin, M. F. (2023). Introduction. In M. F. El-Amin (Ed.), Numerical Modeling of Nanoparticle Transport in Porous Media (pp. xix-lx). Elsevier. https://doi.org/https://doi.org/10.1016/B978-0-323-90511-4.00005-8
Fei, S., Liang, L., Paillet, F. L., Steiner, K. C., Fang, J., Shen, Z., Wang, Z., & Hebard, F. V. (2012). Modelling chestnut biogeography for American chestnut restoration. Diversity and Distributions, 18(8), 754-768. https://doi.org/10.1111/j.1472-4642.2012.00886.x
Franceschet, M. (n.d.). Power laws and scale-free networks. Università degli Studi di Udine.
Frelich, L. (2016). Forest dynamics. F1000Res, 5. https://doi.org/10.12688/f1000research.7412.1
Fulbright, D., Lizotte, E. . (2012). Should I Be Growing Chestnuts? Tips for success Mechigan State University. https://www.canr.msu.edu/uploads/236/76562/Chestnut_growing_requirement…
Gilbert, B., Turkington, R., Srivastava, Diane S., Associate Editor: Oswald, J. S., & Editor: Donald, L. D. (2009). Dominant Species and Diversity: Linking Relative Abundance to Controls of Species Establishment. The American Naturalist, 174(6), 850-862. https://doi.org/10.1086/647903
Green, M. H. (1992). Introduction to Modeling1,2. The Journal of Nutrition, 122, 690-694. https://doi.org/https://doi.org/10.1093/jn/122.suppl_3.690
Hardman, J. G., & Ross, J. J. (2006). Modelling: a core technique in anaesthesia and critical care research. BJA: British Journal of Anaesthesia, 97(5), 589-592. https://doi.org/10.1093/bja/ael272
Koirala, S. (n.d.). Soil Texture Map. University of Tokyo. https://hydro.iis.u-tokyo.ac.jp/~sujan/research/gswp3/soil-texture-map…
Kroll, J. (2023). The Benefits of Planting Chinese Chestnut Trees for Wildlife. https://wildtree.co/blog/the-benefits-of-planting-chinese-chestnut-tree…
Qi, Y., & Yang, X. (2021). Study on breaking mechanism of chestnut shell based on finite element analysis. Journal of Physics: Conference Series, 1865, 032001. https://doi.org/10.1088/1742-6596/1865/3/032001
Schmid, J. S., Taubert, F., Wiegand, T., Sun, I. F., & Huth, A. (2020). Network science applied to forest megaplots: tropical tree species coexist in small-world networks. Sci Rep, 10(1), 13198. https://doi.org/10.1038/s41598-020-70052-8
Seo, H., Kim, W., Lee, J., & Youn, B. (2013). Network-based approaches for anticancer therapy (Review). International journal of oncology, 43(6), 1737-1744. https://doi.org/10.3892/ijo.2013.2114
Shinozaki, K., Yoda, K., Hozumi, K., & Kira, T. (1964). A quantitative analysis of plant form-the pipe model theory: II. Further evidence of the theory and its application in forest ecology. Japanese journal of ecology, 14(4), 133-139.
Soberón, J., & Osorio-Olvera, L. (2023). A dynamic theory of the area of distribution. Journal of Biogeography, 50(6), 1037-1048. https://doi.org/10.1111/jbi.14587
Vliet, T. V. (2004). American Chestnut.
Wright, J. R., Matthews, S. N., Pinchot, C. C., & Tonra, C. M. (2022). Preferences of avian seed-hoarders in advance of potential American chestnut reintroduction. Forest Ecology and Management, 511, 120133. https://doi.org/https://doi.org/10.1016/j.foreco.2022.120133
Yi, X., Steele, M. A., & Shen, Z. (2014). Manipulation of walnuts to facilitate opening by the great spotted woodpecker (Picoides major): is it tool use? Animal Cognition, 17(1), 157-161. https://doi.org/10.1007/s10071-013-0695-y
Yuan, Y., Zhao, Z., Xu, Y., Dang, X. a., Yang, L., Zhang, C., & Yuan, Y. (2013). Heat–Mass Transfer Coupled with Stress–Strain Model and Simulation for Vacuum Shelling of Chestnuts. Drying Technology, 31(5), 527-534. https://doi.org/10.1080/07373937.2012.745090
Government of Canada. (2018). American chestnut (Castanea dentata) COSEWIC assessment and status report: chapter 8. Environment and Climate Change Canada (ECCC). Retrieved from https://www.canada.ca/en/environment-climate-change/services/species-risk-public-registry/cosewic-assessments-status-reports/american-chestnut/chapter-8.html
Massantini, R., Moscetti, R., & Frangipane, M. T. (2021). Evaluating progress of chestnut quality: A review of recent developments. Trends in Food Science & Technology, 113, 245-254. https://doi.org/https://doi.org/10.1016/j.tifs.2021.04.036
Pinto, D., Braga, N., Silva, A. M., Costa, P., Delerue-Matos, C., & Rodrigues, F. (2020). Chapter 6 - Chestnut. In C. M. Galanakis (Ed.), Valorization of Fruit Processing By-products (pp. 127-144). Academic Press. https://doi.org/https://doi.org/10.1016/B978-0-12-817106-6.00006-X
Simpson, M. G. (2010). 8 - Diversity and Classification of Flowering Plants: Eudicots. In M. G. Simpson (Ed.), Plant Systematics (Second Edition) (pp. 275-448). Academic Press. https://doi.org/https://doi.org/10.1016/B978-0-12-374380-0.50008-7