Table of Contents
Keywords: xylem, phloem, hydraulic efficiency, hydraulic safety, pinecone, needles, samara, autorotation, sound attenuation, hydro-actuation
Abstract
From a physical perspective, the pine tree’s very design embodies resilience. Pines are among the few trees to not only survive the winter, but flourish in it. This paper presents a detailed analysis on the various biophysical properties of the Pinus that allow it to endure such challenges. From their seeds and cones to their interior and exterior structure, pine trees have developed many adaptations allowing them to thrive in their environment. Inside the pine, the fluidics of sap and resin allow the tree to survive dry climates and insect attacks. Characteristics in the structure of pine needles and the mechanics of pinecones have also been shown to aid in managing both humid and dry climates. A multitude of trees separate nutrient and water delivering tasks between the xylem and the phloem, as does the pine tree. By developing a nutrient delivery process unique to pine needles, the pine tree presents efficient solutions to the harsher climates it inhabits (Tapping into Health: Unlocking the Mysteries of Tree Sap and its Remarkable Uses, 2025). Mechanisms in pinecones control when pine seeds are released for dispersal based on the environmental conditions. The aerodynamic properties of pine seeds allow for efficient seed propagation via wind dispersal. Sound attenuation properties of pine forests can also create a better environment for wildlife, which in turn contributes to the survival of the forest.
Introduction
Historically, Pinus appeared around 150 mega-annum, during the Mesozoic Era, and spread across the northern continent during the Crustacean period. By the mid-Crustacean period, the pine ancestor diverged into two lineages of genus: Strobus (Haploxylon) and Pinus (Diploxylon) (Keeley, 2012). Haploxylon, or soft pines, have needles in bundles of five or four, little resin, and stalked cones. Their timber is soft, with close-grained wood. Diploxylon, or hard pines, typically have needles in bundles of two or three, large amounts of resin, and cone scales with prickles. Their timber is harder, with coarse-grained wood that are darker colours (“Pines”, 2025). Versatile conifers, pine trees are the most widespread type of conifer across the globe. Figure 1 showcases a few remarkable types of pines, native to different areas of the northern temperate region.

Fig. 1. a) The sugar pine, or Pinus lambertiana, is the tallest known pine of the diploxylon lineage, native to North America (adapted from “Pinus lambertiana”, 2025). b) The gnarly bristlecone pine, or Pinus longaeva, is an extremely long-living pine restricted to mountaintops. A haploxylon, bristlecones are native to North America (adapted from “Pines”, 2025). c) The scotch pine, or Pinus sylvestris, is the widest dispersed pine of Eurasia. A diploxylon, it is native to northern Europe (adapted from “Pines”, 2025). d) The Austrian pine, or Pinus nigra, is widely cultivated as an ornamental. A diploxylon, it is native to Europe and western Asia (adapted from “Pinus nigra”, 2025).
In the Strobus lineage, most species are situated in alpine or desertic environments with extreme heat or extreme cold conditions. For the subgenus Pinus, forest fires are a common threat since their high resin content increasing their susceptibility to combustion. The Strobus lineage, however, develop their densely packed needles and thin barks from their distribution in ecosystems where fires are not a regular feature. On the other hand, the Pinus lineage, which incorporates most pine trees, develop higher canopies and thicker barks to adapt to fire regimes common to their ecosystems. Reproduction is often delayed until fires expose mineral soil, rich in nutrient for potential seedlings (Keeley, 2012). The Mesozoic period’s active fire occurrences support the pine tree’s adaptive evolution to different fire regimes in addition to adaption to geology and climate.
Fluidic Properties of Pine Trees
Hydration and Nutrient Transport
The pine tree’s ability to survive in harsh conditions is largely dependant on the plant’s hydration and transport of nutrition through its internal structures. A pine tree’s roots absorb water and nutrients from the soil and simple sugars from its needles, both of which are then spread throughout the tree (Spengler, 2023). The sugars are transformed from sunlight, water, and carbon dioxide as the plant undergoes photosynthesis. These nutrients and sugars are carried by a viscous liquid, sap, crucial to the survival of the tree, supporting its growth and metabolism (Spengler, 2023). It transports hormones throughout the plant, controlling development and reactions to external stimuli (Penrose, 2018). Additionally, without sap hydrating the tree, it would wilt and become susceptible to diseases and pests. Sap, which is mostly composed of water, carries its sugars as if flows through the phloem and xylem (Penrose, 2018).
The phloem is the fibrous tissue under the bark that carries the sugars from the leaves down the tree (Petruzzello, 2025). However, this process in pine trees is different from that of broadleaf trees. The phloem is composed of specialized cells, forming the sieve tube and parenchyma structures. The sieve tubes have perforations in the walls that provide the main channels for the substances that travel through the tree (Petruzzello, 2025). In broadleaf trees, the sieve tubes would begin at the leaf but for pine needles, the arrangement of the veins poses a problem since the transport of sugar will stagnate at the tip (Bohr, 2023). So, the sieve cells start at different points along the needle, as seen in Figure 2, while transfusion tissue, illustrated in Figure 3, directs the sugars to the correct tube. This tissue is composed of a complex interdigitated network of sugar and water-carrying cells. Transfusion tissue is unique to conifers, explaining how pine trees are so resilient in the face of harsh dry and cold conditions. Found at the end of the sieve tubes are the parenchyma cells, thin-walled unspecialized cells, to facilitate the flow of sugars (Bohr, 2023).

Fig. 2. An image of the sieve cells along bark of Pinus Strobus (Mauseth, 2001)

Fig. 3. A cross-sectional diagram of the pine needle, illustrating the xylem, phloem, and transfusion tissue (Own work by Amanda Kawwas, 2025).
The xylem is the porous tissue in the tree’s vascular system, transporting water and dissolved minerals from the roots up the tree (Wagner et al., 2023). The water travelling through the xylem ensures that the entire tree receives the necessary moisture for growth and survival. It consists of a variety of specialized water-conducting cells known as tracheary elements. One of the tracheary elements that water passes through is the tracheid, portrayed in Figure 4. Subsequently, the water is filtered by the pit membranes, preventing the passage of air bubbles. This structure is crucial to the plant’s survival as the presence of an embolism could disrupt the flow of water through the tree, blocking the water-conducting elements of the plant. The parenchyma cells found in the xylem tissue allow for the storage of various substances (Wagner et al., 2023).

Fig. 4. Secondary xylem tracheids with circular bordered pits, composed of pit membrane in Pinus species. Bar=50 μm (Elsevier, 2009)
The cellular makeup and function of the xylem enable the structure’s filtering properties (Petruzzello, 2025). Since it is made up of tiny pores, it can trap chemicals and microbes that flow through it, similar to the function of dialysis machines. It can remove over 99 percent of the bacteria in the sap flowing through it (Tetro, 2014). This helps the tree avoid bacterial infections, some of which can cause plant death in the span of a few days (Yadeta & J. Thomma, 2013).
Pine Resin: A Defense Mechanism
A common misconception about pine trees is that sap and pine resin are the same substance (Vázquez-González et al., 2020). Resin is thicker than sap, secreted by resin ducts, tubular structures that produce the resin, when a tree is injured to protect and heal the wound. There are different kinds of resin ducts found in both the xylem and the phloem, some of which are even connected to one another, creating a complex network that ensures an abundance of resin (Vázquez-González et al., 2020). In western North America, there have been various mountain pine beetle outbreaks responsible for the killing of millions of acres of pine forests (Zhao & Erbilgin, 2019). To survive such conditions, the pine trees developed larger, but fewer, resin ducts (Zhao & Erbilgin, 2019. Research has shown that the enlargement of the resin ducts is a crucial defence mechanism in pine survival against future beetle attacks (Zhao & Erbilgin, 2019).
Hydraulic Behavior in Droughts
Decreased moisture in the soil reduces water transport, photosynthetic rates, and carbon uptake, weakening the tree. The xylem hydraulic structure influences the physiological responses to such extreme environmental conditions, determining the pine trees’ plasticity under water-limited conditions (Guérin et al., 2020).
The optimization of water transport, or hydraulic efficiency, positively correlates the xylem’s cellular makeup to the growth rate of the tree (Ziaco et al., 2023). The xylem’s conduit size determines the amount of water able to flow through the stem, affecting the tree’s hydration during cell formation (Zhao et al., 2021). Thus, primary growth, or the height of the tree, increases exponentially with conduit size. Similarly, a more efficient xylem is associated with larger secondary growth, observed in the tree-ring area, also known as the basal area increment. Anatomical traits that promote efficiency like enlarged tracheid lumen area are found in pine trees, explaining their ability to grow so tall under less favorable conditions.
Pine trees have a natural efficiency-safety trade off, balancing facilitating effective water transport and preventing xylem implosion. Resistance to implosion under highly negative pressures, experienced during droughts or extreme cold, is determined by the thickness of the cell walls relative to conduit size. In straining environments, hydraulic safety is prioritized in xylems, resulting in reduced radial growth. Regardless of the trade off, efficiency can overpower safety in determining stem growth, even in water-limited conditions (Ziaco et al., 2023). Such water-retaining characteristics are found not only within the internal wood anatomy but also in external structures like pine needles.
Mechanical Structure of Pine Needles and Cones
Pine Needles In Different Climates
Needles in the subgenus of Pinus are adapted to the rainfall and wet climates that pine trees are situated in. These needles prominently exhibit abilities for moisture equilibrium and resistance to raindrop impact.
The structure of the pine needle is semi-conical, the apex angle of the tip of the needle decreasing towards the base direction, with a wedge-shaped cross-section (Lebanoff & Dickerson, 2020). Pits and grooves arrange linearly along the body of the needle. Wan et al. tested Pinus tabuliformis needles’ water collection abilities by first placing a small droplet on the apex angle of the needle to imitate condensation of fog and observing the behaviour of its movements along the body (Wan et al., 2019). The initial droplet at the apex angle moves towards the root of the needle, coalescing with other smaller droplets along the needle, due to Laplace pressure, expressed by the equation:

Where is the local radius of the needle, is the droplet radius, are the local radii of the needle on either side of the water droplet, is the surface tension of water, and is the incremental radius of the needle. Additionally, it was found that as droplets approach the root of the needle, the surface becomes more hydrophilic. This movement down the body of the needle is discrete (Wan et al., 2019) and is attributed to a “pinning effect”. As shown in Figure 5, as droplets gather, the force increases to a point that overcomes this pinning effect, due to combined influences of the Laplace pressure, surface wettability, and the surface tension of water along the channeling grooves. At a mist flow of 1.2 m/s, the pine needle can collect 1.2 ml of water per ten minutes (Wan et al., 2019).

Fig. 5. (a-b) In situ optical microscopic observation of the directional water collection on the pine needle placed at 0° and 90°. (c) The water droplets could spread from the tip to the root of the pine needle. (d) The shape gradient rise the Laplace pressure at the two opposite sides of the droplet. Scale bars, 500 μm (Wan et al., 2019).
The Chinese red pine, or Pinus tabuliformis, the subject of Wan et al.’s study, is a pine of the subgenus Pinus, commonly found in northern China. This type of pine prefers dry, sunny, hills and slopes (Farjon, 2013). Due to its ecology, this pine has developed its needles to adapt to conditions such as lower temperatures and water depletion (Zhang, 2010; Liu, 2012, as cited in Zhang et al. 2017). The Chinese red pine’s needles, consequently, perform well in gathering moisture in its dryer habitat. Another similar study on needle shapes by Lebanoff & Dickerson observes the longleaf pine (Pinus palustris), a pine that prefers the opposite extreme in habitat: bio-diversified forests prone to fire (Lebanoff & Dickerson, 2020).
The needles of the longleaf pine present a wedge-up orientation that performs well in splitting impacting water drops, minimising resultant forces acting on the needle and the soil underneath. Less prone to mass capture, this specific pine appears to be rejecting the accumulation of moisture from rain (Lebanoff & Dickerson, 2020). Of the Pinus variety as well, longleaf pines are dependent on fire to eliminate habitat competition and to expose mineral-rich soils. Their environment is rich in biodiversity, the longleaf pine’s long needles protecting the ecosystem on the ground by reducing the kinetic energy of raindrops (Lebanoff & Dickerson, 2020).
Hygroscopic Movement of Pinecones
The scales of pinecones are composed of dead cells, intricate geometrical structures that undergoes conformational changes during hydration. The mechanism of reversible deformation in pinecones serves to increase the survivability of the pine through efficient seed dispersal (Quan et al., 2021). The current general understanding of the bilayer structure of individual scales of the cone describes its cellular structure as the sclereid layer and the sclerenchyma layer. The sclerenchyma layer is the upper, rigid, layer of scales, consisting of densely packed fibers. The sclereid layer, a more porous and flexible layer, is situated under the sclerenchyma layer. This layer consists of two sub-layers: a more porous layer sandwiched between the sclerenchyma and the second sub-layer, a denser sclereid layer (Quan et al., 2021).
Song et al. conducted a tracking experiment on pinecones studying their hygroscopic driven movements. The study separates the macroscopic scale structure into three layers: bract scales (corresponding to the sclerenchyma layer), fibers (flexible sclereid layer), and inner lignified structure (rigid sclereid layer) (Song et al., 2019). The resulting structural change is induced by water droplets reaching the inner scales. As Figure 6 shows, only a small deformation occurs on a small section on the root of the scale attached to the midrib of the cone, the movement otherwise only amplified by the body of the scale (Reyssat & Mahadevan, 2009).

Fig. 6. Cone scale in its wet (a) and dry (b) states, where θ is the angular position of the scale, the dry state being chosen as a reference (θ = 0°) (adapted from Reyssat & Mahadevan, 2009).
Song et al.’s study confirms that the three layers of scale structure prevent water droplets from flowing directly into the center of the cone and direct the water into scales as a higher priority destination. Smaller pores line the exterior bract scales, while larger pores line the middle layer. However, microfibrils in the bract scales vary in angles and have inconsistent orientations, whereas microfibrils in the sclereid demonstrate uniform orientation. Water is absorbed first between bract scales and fibers, driven by the preferential flow phenomenon, where water prioritises the channel that is the most thermodynamically favorable (Brindt et al., 2023). Figure 7 details the pathway water follows into the center of the pinecone, directed by the upward pointing angle of the bract scales. The water between these two layers then spreads, quickly saturating surface areas. The wetted scale areas have water filling up pores of the bract and fibers that are otherwise filled with air when dry, thus inducing morphology changes with incident swelling. Specifically, length and breadth of wet scales increase by 3.0% and 5.5% respectively in comparison to their dry state (Song et al., 2015).
The inconsistent orientation of fibers and pores of the sclerenchyma and sclereid scale layers causes a mismatch in swelling when pores are hydrated. The bending of each individual scales arises from the strain, as water is directed towards the pores of bract scales and fibers. These results demonstrate the pine’s efficient motion in structural changes, minimizing both the amount of water and time used.

Fig. 7. Schematic diagram of a pinecone indicates the route of water transport. 1) The droplet reaches the center of the pinecones 2) Water is absorbed by the bract scales and spreads into the scales and fibers. 3-1) Most water is transported to the inner scales. 3-2) A small amount of water spreads to the fibers 4) The water in scales eventually causes the structural transformation (adapted from Song et al., 2015).
Porous materials of the scales are further explored in an experiment by Quan et al. The study, which used pinecones from Torrey pines (Pinus torreyana), discovered that scale flexure is not driven solely by differential expansion between the two fiber types, as previously thought (Harlow et al. 1964 as cited by Quan et al., 2021). Quan et al. observed longitudinal alignment of sclerenchyma fibers with the sclereid fibers in a cross section of a scale. Both types of layers have pores gradually become less dense in the same direction, as the thickness of the base thins out towards the tip. Pores become larger closer to the heart of the cone, or the side of the scales closer to its root. The porosity gradient is found to contribute significantly to the efficient swelling of scales while bending, directly responsible for directing water to inner layers with larger pores as Song et al. previously found (Quand et al. 2021). Between the outer bract layer (sclerenchyma) and inner fibers (inner sclereid), porous parts of the sclereid cells act as a cushion that eases the mechanical strain whilst scales bend. As the inner, more swellable, layers expand due to outside moisture, the outer, less swellable layer, resists it, causing the entire cone to curl inwardly. Thus, pinecone hydro-actuation depends not only on morphological expansion from water-filled pores, but also on the internal porosity gradient that eases this swelling and ensures reversibility.
Pinecone hydration-actuation is a classic example of effective seed dispersal dependent on convenient environmental conditions. During Quan et al.’s study, some collected Torrey pinecones are found to still contain seeds even when scales are open, concluding that seeds may be gradually released over several cycles of actuation (Quan et al., 2021). The gradient porous structure of the scales ensures reversibility and toughness of bending sites, essential elements to allow multiple cycles of seed dispersal. By extending the seed dispersal period and separating it into cycles, there is an increased chance for the offspring to survive (Quan et al., 2021).
Kinetics in Pine Seed Propagation
Autorotation in Wind-Dispersed Pine Seeds
The scattering of pine seeds occurs in a variety of ways but most commonly by wind dispersion. The main adaptation for this mechanism is the development of winged seeds. Winged pine seeds tend to have a flattened shape to increase its aerodynamic abilities (Vander Wall, 2023). Other structural characteristics of winged seeds, including those of pines, are revealed by a study conducted by Yasuda and Azuma (1997). They consist of a concave bend upwards near where the wing attaches to the seed, a greater thickness on the leading edge, the side of the wing that hits the air first as it rotates and a centre of gravity near the leading edge and the inner part of the seed. Figure 8 shows these characteristics.

Fig. 8. (a) View from above of a pine samara wing where CG is the approximated location of the seed’s centre of gravity. (b) View of cross-section which shows the difference in thickness of the leading edge in comparison to the rest of the samara wing and the upwards concave bend near where the seed and wing meet (Own work by Aisha-Mae Garing-Patel, 2025).
Specifically referred to as samara, these winged seeds autorotate as they fall, lowering their speed of descent to remain airborne as long as possible (Minami & Azuma, 2003). After their release, pine seeds, like other auto-rotating seeds, do not immediately start to rotate but begin shortly after. This autorotation mechanism leads to the lifting force applied on the samara to balance out with its gravitational force (Azuma & Yasuda, 1989), reducing its constant descent velocity (Vander Wall, 2023), also known as a terminal velocity. Azuma and Yasuda (1989) explain that the steady rate of descent occurs along with a constant speed of rotation of the samara and a constant coning angle. The coning angle of a rotating seed, the angle between the horizontal axis and the span axis shown in Figure 9. The span axis is the axis on which the samara lays in the orientation of its wingtip to its seed.

Fig. 9. Demonstration of certain flight variables found in rotating samaras, where CG is the centre of gravity is the radius of the seed from its centre of gravity to the tip of the wing, is the coning angle, is the thrust produced by the samara’s rotation and the flight path plane is the plane along the span axis in which the samara lays (adapted from Jung & Rezgui, 2024).
The analysis of this steady aerial travel (Azuma & Yasuda, 1989) was conducted by the blade element momentum theory (BEM), which includes two theoretical concepts: the blade element theory, a simple theoretical model often used in the aerodynamic modelling of propellers that considers rotating seed’s wing as individual elements, and the momentum theory, which considers the rotating samara as a rotor disk (Jung & Rezgui, 2023). This means that there must be conservation of momentum, a balance between the thrust and the weight of the seed and a net torque of 0 Nm. These relationships can be analyzed using the following equations:


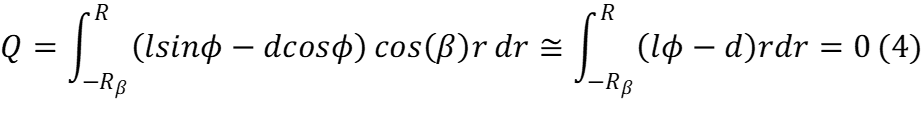
where is thrust (N), 𝜌 is air density (kg/m3), is the area of the imagined disk formed by the rotation of the samara (m2), is the induced velocity which is positive downwards (m/s), is the rate of descent (m/s), is gravitational force Fg, also known as the weight of seed (N) where is its mass (kg) and is the gravitational acceleration (m/s2), is the spanwise lift distribution (N/m), is the spanwise drag distribution (N/m) and is net torque (Nm). Figure 10 illustrates both the inflow angle (𝜙) and the coning angle (𝛽) (Azuma & Yasuda, 1989) noting that inflow angle (𝜙) refers to the angle at which the wind hits the seed during its descent in relation to its plane of rotation (Jung & Rezgui, 2024).

Fig. 10. A visual representation of a winged samara and the variables affecting their autorotation. (a) Dimensional view, where is the radius of the seed from its centre of gravity to the tip of the wing, is the radius of the seed from its centre of gravity to the tip of the seed, is the total length from the wing tip to the seed end of the samara and 𝛽 is the coning angle or flapping angle. (b) Distance view, where 𝜙 is the inflow angle. (adapted from Azuma & Yasuda, 1989).
Furthermore, Jung and Rezgui (2023) explain that another factor plays a role in slowing the descent of samara, that being the leading-edge vortex (LEV) observed in samaras in a study conducted by Lentink et al. (Jung & Rezgui, 2023; Lentink et al. 2009). This mechanism involves the presence of a tornado-like motion above the wing of the seed lowering the air pressure to improve flight performance by increasing lift (Jung & Rezgui, 2023). Figure 11 shows how the air hitting the samara results in the LEV above the wing near its centre of gravity increasing air circulation in that region.

Fig. 11. A horizontal view of a rotating samara showing the leading-edge vortex (adapted from Rezgui et al., 2020).
The autorotation and steady flight of pine seeds, enhanced by the LEV phenomenon, provides three distinct reproductive advantages. First, it decreases competition among seedlings by dispersing them further apart (Nathan et al., 2000). Second, seeds located farther from the parent tree are less likely to be detected by predators (Vander Wall, 2023). Finally, it allows new populations to colonize unoccupied territories.
Environments where crown fires commonly occur are home to types of pines known as fire-embracers (Keeley, 20212). These pines increase the intensity surrounding fires burning down more of the tree canopies to later release their seeds in one pulse. An example of fire-embracer is the Pinus halepensis (Keeley, 2012). As a species of pine with winged samara (Vander Wall, 2023), P. halepensis’ seeds, when released post-fire, can settle in newly cleared territories (Keeley, 2012) further from their parent and from one another due to their lower descent velocity.
Sound Propagation in Pine Forests
Physical Mechanisms of Sound Propagation
In pine forests, sound waves propagate through a heterogeneous environment. Obstacles such as ground irregularity, tree trunks, branches and needles cause diffraction, reflection and scattering of sound waves, which transforms coherent sound into incoherent sound (Tarrero et al., 2008). This conversion occurs because scattered waves return with varying phases, reducing coherence and, in many cases, producing destructive interference that leads to attenuation (Huisman & Attenborough, 1991; Roberts, 2003).
Scattering caused by tree trunks predominantly influences frequencies above 400 Hz, whereas canopy scattering primarily impacts the attenuation in upwind cases. Figure 12 illustrates these cumulative interactions (Swearingen & White, 2007).

Fig. 12. Cumulative contributions of components, upwind case. In each graph, (—) is a homogeneous atmosphere with forest ground impedance. (--) adds the upwind forest profile, (-⋅) adds trunk scattering, and (⋅⋅⋅) adds canopy scattering. The source receiver distance is 315 m. For each parameter, a great transmission loss TL can be observed (Swearingen & White, 2007).
The following model calculates the complete attenuation induced by pine trunk scattering:

The complete attenuation caused by scattering As is calculated by determining the direct field’s energy Ed , the reverberant field’s energy Er and the free field’s energy Ef. In addition, the ground surface of pine forests is another crucial element that influences sound attenuation. The coarseness of the floor becomes an obstacle to noise propagation in the same way as trunks do, mainly for medium- and high-frequency ranges. Here, the same interference mechanism explains the additional loss of coherence, which, combined with trunk scattering, produces a more important effect (Huisman & Attenborough, 1991; Tarrero et al., 2008).
Tree Density, Trunk Diameter and Basal Areas
A proposed model to analyze the sound pressure levels of pine forests is the Nord 2000 model, which can be corrected to account for the effects of trees on sound waves:

The sound pressure level L(r) measured by the receiver accounts for the influence of numerous variables: Lw is the sound pressure level for a certain frequency range, r is the distance, K(z) is the ground effect, Ae(r) is the scattering effect and AA is the sound absorption caused by the atmosphere (Kragh et al., 2002; Trimpop & Mann, 2014). The scattering term Ae(r) is given by the following equation:

This former expression considers the geometrical divergence and scattering ΔL , the corrected height of the scatterers h' , their absorption coefficients α , the corrected distance that accounts for obstacles in the scattering zone r' , the gap between the emitting source and the receiver r and nQ , which is associated with the scattering caused by the pine trees:

This scattering factor depends on both tree density n'' and the mean diameter of the pine trunks d . Since attenuation is related to scattering, both variables directly influence sound propagation. Thus, augmenting tree density or trunk diameter, whether separately or in combination, leads to an increase in sound damping (Tarrero et al., 2008). Figure 13 illustrates this near-linear relationship between sound attenuation and the reduction of tree density in a pine forest (Trimpop & Mann, 2014).

Fig. 13. Attenuation coefficients of sound Klin for a reduced density of pine trees in a forest at different frequencies. A near-linear relationship is observed between the attenuation coefficients and the stock density, which demonstrates the effect of an increase in stock density on sound attenuation (Trimpop & Mann, 2014).
Another significant parameter is the basal area, which refers to the area at breast height of the cross-section of a single tree per hectare. This parameter allows for a more accurate comparison of sound attenuation in forests composed of pine trees with inconsistent trunk diameters and heights (Elledge & Barlow, 2018; Trimpop & Mann, 2014). For frequencies below 1 kHz, thicker trunks enhance attenuation, which is consistent with the initial theory. Interestingly, the predicted effect is inverted for frequencies above 1 kHz. Beyond this value, forests consisting of trees having slimmer stems demonstrate a higher attenuation coefficient. Noticeably, pine stands having basal areas of less than 15 m2/ha seem to have an insignificant effect on the propagation of acoustic waves regardless of frequency, but most pine forests’ basal areas exceed this threshold. Hence, greater attenuation coefficients can be anticipated from these forests (Trimpop & Mann, 2014).
Anthropogenic noise harmfully impacts wildlife by reducing their ability to detect crucial sounds, disrupting their reproductive processes and altering predator-prey dynamics. These disturbances increase stress levels in animals who rely heavily on acoustic signals for communication, leading to behavioural changes, lower habitat quality and detrimental physiological impacts (Francis et al., 2009; Shannon et al., 2016). Through their noise reduction properties, pine forests can help counteract these harmful effects by creating a more favourable habitat for wildlife. In turn, fauna can benefit pine forests by dispersing pinecones, which increases tree population, and by enriching the soil with nitrogen and phosphorus through their fecal deposits (Furiness et al., 2011; Rehling et al., 2023).
Furthermore, pine forests can be used to insulate noisy places. To evaluate how a pine forest could serve as natural acoustic for a small airport, attenuation can be calculated using Eq. (7) and Eq. (8). A representative pine stand with a density of 500 trees/ha can be assumed (n'' = 0.05 trees/m2) along with a mean trunk diameter of 0.23 m, measured from a Montréal pine tree (Zenner & Peck, 2009). A correction term of 3 dB is included to account for divergence and scattering (Huisman & Attenborough, 1991). Using these parameters in Eq. (7) and Eq. (8), the forest attenuates approximately 22.28 dB of sound across a 100 m distance. Aircraft take-off levels at airports can reach 130 dB (How loud is too loud?, 2025), while noise guidelines recommend keeping exposure below 70 dB (Canada, 2024). To achieve this 40 dB reduction, a forest width of about 180 m is required. Assuming a small regional airport length of roughly 3,500 m, the surrounding forest area can be estimated as:

Hence, a 0.63 km² belt of pine forest would be sufficient to reduce airport noise to safe levels for nearby communities.
Sound Paths in Pine Forests
Sound waves can propagate through different paths in pine forests (Figure 14). These paths are often curved lines rather than straight ones because of wind and temperature gradients.

Fig. 14. Possible sound propagation paths in a pine forest: a direct path goes straightly from the emitter to the receptor, another is reflected by the ground and one goes above the canopy (Trimpop & Mann, 2014).
The sound perceived by the receptor is the sum of contributions from all sound paths. The forest’s attenuation can be calculated by the following expression, which accounts for the geometry of the forest, such as sound path length and diffraction near the edges (Trimpop & Mann, 2014):

The attenuation coefficient Aforest depends on the minimal attenuation AISO9612,min , the direct sound path dforest,direct , the sound path above the canopy dforest,diffraction and the attenuation for the direct sound path and the path above the canopy Klin,v and Klin,w , respectively (Trimpop & Mann, 2014). Whilst sound damping has a more important effect for longer distances, it is negligible for path lengths that are shorter than 40 m2 (Swearingen & White, 2007; Tarrero et al., 2008).
Sound Absorption Properties of Pinecones
Pinecones display incredible acoustic absorption capabilities due to their coarse, fibro-granular surfaces and the fine powder laying on their surface, which helps scatter incident acoustic waves. A simple way to quantify pinecones’ absorption properties is by measuring their Noise Reduction Coefficient (NRC). The following equation allows for these calculations (Jang & Kang, 2023):

The NRC corresponds to the average of the absorption coefficients α250, α500, α1000, and α2500 at frequencies of 250 Hz, 500 Hz, 1000 Hz and 2000 Hz respectively.
For each measured height of pinecone particle (Figure 15), different tendencies can be observed. Indeed, higher pinecone particles have optimal absorption at lower frequencies. For example, a 4 cm-high particle had the best sound absorption coefficient of 0.994 at 1100 Hz, whilst the 10 cm-high pinecone particles obtained their highest absorption coefficient of 0.992 at 384 Hz. Additionally, greater heights of these particles lead to a general increase of their NRC. Jang and Kang’s study of sound absorption of pinecones demonstrated that a 10 cm-high pinecone particle could absorb over 60 % of day-to-day environmental noise for frequencies ranging between 250 and 6400 Hz. Nonetheless, even the thinner cone particles absorbed a considerable amount sound energy (Jang & Kang, 2023).

Fig. 15 Example of an impedance tube used to determine the NRC of pinecone particles. Impedance tubes can be filled with pinecone particles of heights varying between 4 and 10 cm (Jang & Kang, 2023).
These sound absorption properties of pinecones can be used for various applications, notably as acoustic panels for noise reduction. However, adhesives such as glue could not be used to manufacture such panels, since the sound damping capabilities of pinecones come from their irregular and coarse surface. Thus, pinecone particles could not be significantly modified in order to preserve these abilities (Jang & Kang, 2023).
Conclusion
In conclusion, the pine tree exemplifies how biological systems embody fundamental physical principles to ensure survival and adaptation. Since the Mezoic era, pine trees’ two subgenera develop unique solutions to their distinctive environments. The more common and widespread genus, the Pinus, presents a variety of trees with vastly different techniques to exist efficiently within their ecosystems. In the pine’s vascular system, the hydraulic balance between efficiency and safety allows the tree to thrive under both dry and freezing conditions. With the xylem filtering sap, preventing bacterial infections, and the resin ducts, creating a defense mechanism against beetle attacks, the fluidics of the pine allows the tree to resist environmental stressors. Needles vary in length and structure in extreme environments that the Pinus gravitate towards. In fire-prone forests, the pine’s needles adapt a wedge-up orientation to avoid retention of rain and moisture, protecting the soil and fauna beneath the tree from high impact forces. On drier and sunnier slopes, the pine’s needles adjust into intricate channels with uniform grooves to capture every bit of moisture in the air and fog. Pinus pinecones, similarly, adjust to environmental factors to optimise seed dispersal. Without hydration-actuation, cones would release seed in wet, humid, conditions, leading to short-range dispersal despite the favourable shapes of pine seeds (Song et al., 2017). The auto-rotational mechanism and presence of a LEV in pine samaras enable further seed propagation via wind dispersal allowing pine seeds to avoid interspecies competition, evade potential predators and populate unoccupied land further from their parent. For instance, in fire-prone environments, pine seeds can disperse further post-fire and populate a greater area of newly cleared land. The acoustic properties of pine trees allow for a better environment for wildlife, which in turn can contribute to its longevity. Altogether, the pine’s fluidics, biomechanics, kinetics, and acoustics contribute to its resilience, demonstrating how the principles of physics can be modeled within one of nature’s most enduring trees.
References
References
Aljos, F., & Eckenwalder, J. E. Pinus - Pine description. In Conifers Garden. https://conifersgarden.com/encyclopedia/pinus
Azuma, A., & Yasuda, K. (1989). Flight performance of rotary seeds. Journal of Theoretical Biology, 138(1), 23-53. https://doi.org/10.1016/S0022-5193(89)80176-6
Bohr, T. (2023). Sap flow and sugar transport in a pine needle: how to deal with an adverse environment. APS March Meeting Abstracts, 2023, Y14.001. https://ui.adsabs.harvard.edu/abs/2023APS.MARY14001B/abstract
Brindt, N., Parlange, J.-Y., & Steenhuis, T. S. (2023). Unstable preferential flow in porous media. In M. J. Goss & M. Oliver (Eds.), Encyclopedia of Soils in the Environment (Second Edition ed., pp. 314-320): Academic Press.
Elsevier. (2009). Pinus sp. secondary xylem tracheids with circular bordered pits (Extant). Bar=50 μm. [Image]. In Science Direct. https://www.sciencedirect.com/science/article/abs/pii/B9780123739728000073.
Elledge, J., & Barlow, B. (2018). Basal Area: A Measure Made for Management. Alabama Cooperative Extension System. https://www.aces.edu/blog/topics/forestry/basal-area-a-measure-made-for-management/.
Farjon, A. (2013). Pinus tabuliformis. The IUCN Red List of Threatened Species. https://doi.org/https://dx.doi.org/10.2305/IUCN.UK.2013-1.RLTS.T42419A2978916.en.
Freidah, J. (2014). Microfluidics and nanofluidics research address global challenges. MIT News. https://news.mit.edu/2014/micro-and-nanofluidics-research-address-global-challenges
Guérin, M., von Arx, G., Martin-Benito, D., Andreu-Hayles, L., Griffin, K. L., McDowell, N. G., Pockman, W., & Gentine, P. (2020). Distinct xylem responses to acute vs prolonged drought in pine trees. Tree Physiology, 40(5), 605–620. https://doi.org/10.1093/treephys/tpz144
Huisman, W. H. T., & Attenborough, K. (1991). Reverberation and attenuation in a pine forest. The Journal of the Acoustical Society of America, 90(5), 2664–2677. https://doi.org/https://doi.org/10.1121/1.401861
Jang, E. S., & Kang, C. W. (2023). Investigation of sound absorption capability of pine (Pinus densiflora) cone particles. Journal of Wood Science, 69(1). https://doi.org/https://doi.org/10.1186/s10086-022-02075-w
Johnson, C. Y. (2016). Pine tree’s tissue for moving sap holds promise as water filter. The Boston Globe. https://www.bostonglobe.com/metro/2014/03/09/mit-engineers-test-low-tech-water-filter-inspired-nature/fpq416KF2TQ3IpRSZk8pML/story.html
Jung, B. K., & Rezgui, D. (2023). Sectional Leading Edge Vortex Lift and Drag Coefficients of Autorotating Samaras. Aerospace, 10(5), 414. https://www.mdpi.com/2226-4310/10/5/414
Jung, B. K., & Rezgui, D. (2024). Experimental study into the effects of pitch and coning angles on the flight performance of the natural samara. Royal Society Open Science, 11(9). https://doi.org/10.1098/rsos.240758
Keeley, J. E. (2012). Ecology and evolution of pine life histories. Annals of Forest Science, 69(4), 445-453. https://doi.org/10.1007/s13595-012-0201-8
Lebanoff, A. P., & Dickerson, A. K. (2020). Drop impact onto pine needle fibers with non-circular cross section. Physics of Fluids, 32(9), 092113. https://doi.org/10.1063/5.0019310.
Lentink, D., Dickson, W. B., Leeuwen, J. L. v., & Dickinson, M. H. (2009). Leading-Edge Vortices Elevate Lift of Autorotating Plant Seeds. Science, 324(5933), 1438-1440. https://doi.org/10.1126/science.1174196
Mauseth, J. (2001). Longitudinal section of pine bark (Pinus strobus) [Image]. In School of Biological Sciences. http://www.sbs.utexas.edu/mauseth/weblab/
Minami, S., & Azuma, A. (2003). Various flying modes of wind-dispersal seeds. Journal of Theoretical Biology, 225(1), 1-14. https://doi.org/10.1016/S0022-5193(03)00216-9
Penrose, N. (2018). What Time of Year Do Pine Trees Drip Sap? https://bigtreesupply.com/blog/what-time-of-year-do-pine-trees-drip-sap/
Petruzzello, M. (2016). Xylem | plant tissue. In Encyclopædia Britannica.
https://www.britannica.com/science/xylem
Popolizio, T. (2024, October 7). Transport of Food in Plants. Pressbooks.pub; ROTEL (Remixing Open Textbooks with an Equity Lens) Project. https://rotel.pressbooks.pub/understanding-organisms/chapter/transport-of-food-in-plants/.
Przykuta. (2010). Pinus nigra (Polski: Sosna czarna w parku w Świerklańcu). English Wikipedia. https://en.wikipedia.org/wiki/Pinus_nigra#/media/File:%C5%9Awierklaniec_pinus_nigra_12.06.2010_p.jpg

Quan, H., Pirosa, A., Yang, W., Ritchie, R. O., & Meyers, M. A. (2021). Hydration-induced reversible deformation of the pine cone, . Acta Biomaterialia, 128, 370-383. https://doi.org/https://doi.org/10.1016/j.actbio.2021.04.049
Reyssat, E., & Mahadevan, L. (2009). Hygromorphs: from pine cones to biomimetic bilayers. Royal Society Interface, 6(39). https://doi.org/https://doi.org/10.1098/rsif.2009.0184
Rezgui, D., Arroyo, I. H., & Theunissen, R. (2020). Model for sectional leading-edge vortex lift for the prediction of rotating samara seeds performance. The Aeronautical Journal, 1236-1261. https://doi.org/10.1017/aer.2020.25
Roberts, B. L. (2003). The Decibel Scale. D. o. Physics. https://physics.bu.edu/py231/db3.pdf
Song, K., Chang, S.-S., & Lee, S. J. (2017). How the pine seeds attach to/detach from the pine cone scale? Frontiers in Life Science, 10(1), 38-47. https://doi.org/10.1080/21553769.2017.1287777.
Song, K., Yeom, E., Seo, S.-J., Kim, K., Kim, H., Lim, J.-H., & Lee, S. J. (2015). Journey of water in pine cones. Scientific Reports, 5. https://doi.org/https://doi.org/10.1038/srep09963
Spengler, T. (2023). Pine Tree Sap Season: Pine Tree Sap Uses And Information. Gardening Know How. https://www.gardeningknowhow.com/ornamental/trees/pine/pine-tree-sap-information.htm
Swearingen, M. E., & White, M. J. (2007). Influence of scattering, atmospheric refraction, and ground effect on sound propagation through a pine forest. The Journal of the Acoustical Society of America,122(1), 113-119. https://doi.org/10.1121/1.2735108
Tapping into Health: Unlocking the Mysteries of Tree Sap and its Remarkable Uses. (2025). Tree Plantation. https://www.treeplantation.com/tree-sap.html
Tarrero, A. I., Martín, M. A., González, J., Machimbarrena, M., & Jacobsen, F. (2008). Sound propagation in forests: A comparison of experimental results and values predicted by the Nord 2000 model. Applied Acoustics, 69(7), 662-671. https://doi.org/https://doi.org/10.1016/j.apacoust.2007.01.007
Tetro, J. (2014). How Pine Trees Can Make Water Pristine. https://www.huffpost.com/archive/ca/entry/how-pine-trees-can-make-water-pristine_b_4885663
The Editors of Encyclopedia Britannica. (2025, September 17). Pine [Webpage]. Encyclopedia Britannica (Major North American Pines). https://www.britannica.com/plant/pine/Major-North-American-pines.
The Editors of Encyclopedia Britannica. (2025, September 17). Pine [Webpage]. Encyclopedia Britannica (Physical description and natural history). https://www.britannica.com/plant/pine#ref417098.
Trimpop, M., & Mann, P. (2014). Determination of noise damping by forests Inter-noise, https://acoustics.asn.au/conference_proceedings/INTERNOISE2014/papers/p499.pdf
Vander Wall, S. B. (2023). Seed Dispersal in Pines (Pinus). Botanical Review, 89, 275-307. https://doi.org/10.1007/s12229-023-09288-8
Wan, Y., Cui, P., Xu, J., & Yu, H. (2019). Directional water-collecting behavior of pine needle surface. Materials Letters 255. https://dx.doi.org/10.1016/j.matlet.2019.126561.
Wagner, Y., Volkov, M., Nadal‐Sala, D., Ruehr, N. K., Hochberg, U., & Klein, T. (2023). Relationships between xylem embolism and tree functioning during drought, recovery, and recurring drought in Aleppo pine. Physiologia Plantarum, 175(5). https://onlinelibrary.wiley.com/doi/10.1111/ppl.13995
What Happens to Trees in a Heatwave? (2019). https://alpinetreenj.com/heatwave-heat-stress-affects-trees/.
Willmcw. (2005). Sugar Pine (Pinus lambertiana). English Wikipedia. https://en.wikipedia.org/wiki/Pinus_lambertiana.
Yadeta, K. A., & J. Thomma, B. P. H. (2013). The xylem as battleground for plant hosts and vascular wilt pathogens. Frontiers in Plant Science, 4. https://doi.org/10.3389/fpls.2013.00097.
Yasuda, K., & Azuma, A. (1997). The Autorotation Boundary in the Flight of Samaras. Journal of Theoretical Biology, 185(3), 313-320. https://doi.org/10.1006/jtbi.1996.0299
Zhao, H., Jiang, Z., Zhang, Y., Jiang, B., & Cai, J. (2021). Hydraulic efficiency at the whole tree level stably correlated with productivity over years in 9 poplar hybrids clones. Forest Ecology and Management, 496. https://doi.org/10.1016/j.foreco.2021.119382
Zhao, S., & Erbilgin, N. (2019). Larger Resin Ducts Are Linked to the Survival of Lodgepole Pine Trees During Mountain Pine Beetle Outbreak. Frontiers in Plant Science, 10. https://doi.org/10.3389/fpls.2019.01459
Zhang, M., Meng, J.-X., Zhang, Z.-J., Zhu, S.-L., & Li, Y. (2017). Genetic Analysis of Needle Morphological and Anatomical Traits among Nature Populations of Pinus Tabuliformis. Journal of Plant Studies, 6(1), 62. https://doi.org/10.5539/jps.v6n1p62 https://doi.org/https://doi.org/10.1016/j.foreco.2021.119382
Ziaco, E., Liu, X., & Biondi, F. (2023). Dendroanatomy of xylem hydraulics in two pine species: Efficiency prevails on safety for basal area growth in drought-prone conditions. Dendrochronologia, 81. https://doi.org/https://doi.org/10.1016/j.dendro.2023.126116