
Table of Contents
Keywords: Pollination, Turgor Pressure, Internal Thermal Regulation, Ring shake, Glulam Ectomycorrhiza Symbiosis, Wasp parasitism, Seed Hoarders Mutualism.
Abstract
Chestnut trees (Castanea) use various mechanisms and strategies to adapt to biological pressures and to interact with their environment. In essence, this paper highlights the main physical, morphological, and structural properties of chestnut trees by exploring specific characteristics of different species. The American chestnut has two key evolutionary adaptations: flower structures that attract insects to help spread heavy pollen, and highly effective dehydration tolerance. Internal thermal regulation mechanisms and the sweet chestnut’s response to heat stress and cold temperatures are also discussed. However, a deeper analysis of the mechanical stress sustained by the tree reveals multiple weaknesses in its susceptibility to ring shake, due to its ring-porous material and its ray volume. Furthermore, the chestnut tree’s direct interaction with its environment, via symbiotic relationships, enhances its physical robustness, particularly through its root system, and ensures its growth.
Introduction
The chestnut tree, part of the Castanea genus, is a popular tree found across the world. Its most significant and popular species are the Chinese chestnut (C. mollissima) (Fig. 1), Japanese chestnut (C. crenata), Sweet (or European) Chestnut (C. sativa), and American chestnut (C. dentata), found in temperate Eastern Asia, Southern Europe, the Caucasus mountains, and Eastern North America, respectively (Miller, 2014). Each species has slight variations on leaf form (Fig. 2), nut size and toxicity, stem buds, and more (The American Chestnut Foundation, n.d). The tree and its chestnuts have held cultural significance for centuries, both as timber for homes and as a food source for wildlife and humans.

Fig. 1. Young Chinese chestnut tree (Franklin, 2012).

Fig. 2. Front view of chestnut tree leaves showing shape and size variations between species (The American Chestnut Foundation, n.d.).
In the 20th century, the American chestnut was severely impacted by a blight caused by the Cryphonectria parasitica fungus. The fungus was brought to America by the Japanese chestnut, devastating most of the population and bringing it to endangered levels. A restoration process has been in effect over the last couple of decades, but the American chestnut is still far from its original status (Fredericksen et al., 2021).
The different species are all similar in terms of their climate requirements, reproductive strategies, and morphological development. However, they differ in their density, turgor pressure, chestnut shape, and other physical properties. While the American chestnut is highly affected by the fungus, the Chinese chestnut is almost immune to its effects (Miller, 2014). Learning more about the mechanics behind the chestnut tree and its nut, along with how different species compare to each other, deepens our understanding of the tree and helps us develop stronger methods on how to restore the American chestnut.
Physical and Morphological Adaptations
Pollination
Chestnut trees, a cross-pollinated species, have been for a long time the center of multiple scientific debates regarding their primary pollination vector – whether it is insects or wind. Multiple recent studies have perfected their experiment methods and concluded that chestnut trees are insect-pollinated, despite their resemblance to wind-pollinated species. By using fine mesh nets that blocked insects but allowed airflow, researchers like Petit and Larue (2022) proved that at least 94% of chestnut flowers depend on insect pollination.
On a more physical basis, wind pollination depends on the aerodynamic characteristics of pollen grains and their capacity to be airborne long enough to reach another flower’s stigma. In general, wind-pollinated plants tend to produce dry, small, and very lightweight pollen grains to maximize their resulting motion through the air (Timerman & Barrett, 2021). An important parameter for estimating the theoretical dispersal distance of pollen grains falling through the air is the settling speed, a concept governed by Stoke’s law that applies for small spherical particles falling through a fluid medium. According to this principle, the value of the drag force – a force opposing the motion of an object – impacts the settling velocity of the particle, which is proportional to the mass and density of the particle (Di-Giovanni et al., 1995). However, while there is no strong evidence of chestnut pollen grains having an extraordinarily high mass or density, it can be hypothesized that their shape limits their aerodynamic properties (Snowsill, 2010). Indeed, unlike many wind-pollinated species, the lack of sacci in the grain’s structure, light air-filled bladders, may reduce their average dispersal distance (Fig. 3). The absence of sacci reduces the surface area of the grain, which decreases the resistance force from the air, increases terminal velocity and limits terminal distances (Schwendemann et al., 2007).

Fig. 3. Photographs taken using a scanning electron microscope of a) Eastern White Pine’s pollen grain (Pinus strobus) (Adapted from Schwendemann et al., 2007) and b) rehydrated Chinese chestnut’s pollen grain (Adapted from Buchner et al., 2020). The Eastern White Pine is a wind-pollinated species and its pollen grains present sacci, in contrast of the Chinese chestnut’s pollen grain.
Also, the relatively small size of the pollen grain (10-25 μm) may limit its momentum and its ability to pass through the boundary layer of the female flower (Timerman & Barrett, 2021). Moreover, the forest canopies where chestnut trees typically grow limit airflow and turbulence, reducing the chance of pollen grains being carried horizontally to a receptive stigma. Pollen grains will more likely fall to the ground near the trunk of the tree.
In contrast, chestnut trees present a lot of morphological and physical traits that are favorable for insect pollination. The most remarkable one is the fact that female flowers present six to eight rigid and upright styles at the end of which there is a small stigma (Fig. 4). The erect styles provide a large surface area for the insects to lay on and increase the probability of contact between pollen and stigmas. It is interesting to observe that the crater-shaped stigmas are unsuitable for capturing pollen diluted in the air but are perfect for insects to pollinate (Larue & Petit, 2024).

Fig. 4. Photography of the outside (left) and inside (right) of a female Chinese Chestnut flower. A white cluster of styles can be observed at the top of the structure. The cone-shaped stigma, at the end of the style, captures the pollen when insects pass by (Miller, 2014).
Furthermore, the Chestnut tree is a monoecious species, meaning that male and female flowers grow on the same tree, but are self-incompatible (Westbrook et al., 2020). Bisexual catkins (Fig. 5), where both female and male flowers develop, are an uncommon but very interesting structure from a physical point of view. The male flower attracts various pollinators with its strong odor and abundant nectar secretions. The nectar at the flower's base fluoresces under ultraviolet light (Fig. 6), which is visible to insects and further confirms that the species is insect-adapted. Along with that, the structural arrangement of bisexual catkins promotes insect-pollination through direct mechanical contact by placing female and male flowers in proximity. Beetles represent 78% of the insects found on female flowers, with the common red soldier accounting for 64% of those visits (Larue & Petit, 2024). Because these insects move by crawling, they are very likely to brush pollen from another tree against a receptive female flower at the base of the bisexual catkin. So, the pollination seems to rely more on a stochastic physical contact system than on precise pollen placement.

Fig. 5 Photography of a bisexual inflorescence on a bisexual catkin on a Chinese Chestnut. The female flower is located at the base of the catkin, while the male flower is situated at the tip (Qiu et al., 2025).

Fig. 6 Photographs of a bisexual catkin under visible light (left) and ultraviolet light (UV)(right). Under visible light, both male and female flowers appear yellow. Under UV light, the base of the male flower, containing the nectar, fluoresces, while the female flower doesn’t (Larue & Petit, 2024).
Turgor Loss Point
Turgor pressure is a fundamental physiological characteristic of plant tissues, playing a major role in plant growth. It refers to the positive hydrostatic pressure exerted by water, contained in the plant cell’s vacuole, against the cell walls, helping it maintain its size and shape (Ghosh, 2017). During drought, evaporation and lack of water cause the dehydration of leaf cells, resulting in a decrease in turgor pressure and wilting leaves. The physiological threshold at which the leaf water potential drops to zero (Farrell et al., 2017) and causes the plant to wilt (Su et al., 2022) is called the Turgor loss point (TLP). While it has been proven by multiple studies that the TLP of a plant is related to drought tolerance, this concept also includes numerous physical traits, including osmotic pressure, cell wall mechanics, and water potential gradient.
Turgor pressure is directly related to the physical concept of cell walls' elasticity and osmotic potential (Zhang et al., 2024)(Fig. 7). This latter refers to the capacity of the cell to retain or attract water under drought conditions. A negative water potential results when, under water stress, plant cells accumulate osmotically active solute to attract water by osmosis – the diffusion of water from a low concentration of solute to a high concentration of solute (Sharma et al., 2019). This biophysical adaptation delays the Turgor pressure drop and lowers the Turgor loss point – usually measured in megapascal. Therefore, a negative turgor loss point is associated with better drought resistance (Blackman, 2018).

Fig. 7. Representation of Turgor Pressure, Wall Pressure, and Osmotic Pressure in a turgid plant cell. The water contained in the vacuole creates internal pressure, which is countered by the wall pressure, external pressure. The turgor pressure is maintained and controlled by osmotic pressure (Camille Lebourg’s own artwork).
American chestnut tends to grow on sunny sites with well-drained, moist acidic soil and can also be found on dry sites (Kane et al., 2020). Chinese chestnut can grow under the same conditions, but this species needs to have optimum soil water conditions during its growing season (Revord, 2022). This difference in growth under drought can partly be explained by TLP. Reliable data from the Canadian Journal of Forest Research (Fredericksen et al., 2021) reveals the correlation between TLP and drought resistance for the American chestnut and the Chinese chestnut. Indeed, using the method of osmotic data at full leaf turgor, the study reports that TLP can be estimated at -2.375 MPa for the American chestnut leaves, which is significantly more negative than the Chinese chestnut TLP estimated at -2.125 MPa, (Fig. 8). Those results imply that American chestnut have a better capacity to contain water during drought, giving it an important physical advantage.

Fig. 8. Estimation of Turgor loss point (MPa) for American chestnut, Chinese chestnut. The median of the turgor loss point for American chestnut can be estimated at -2.375MPa, while the median of the turgor loss point for Chinese chestnut can be estimated at -2.125 (Adapted from Fredericksen et al., 2021).
Having a lower (more negative) TLP, used as a mechanism of a dehydration tolerance strategy, can directly impact the ecological performance of the tree. Cell wall mechanics, photosynthesis, and growth are factors that can be maintained when the leaf remains turgid despite decreasing water availability (Álvarez-Cansino et al., 2022). Indeed, research has proven that the American chestnut tends to keep its stomata open under drought conditions to maximize photosynthesis, a risky strategy, while the Chinese chestnut adopts a more conservative approach by closing its stomata earlier to prevent water loss (Fredericksen et al., 2021). Given its endangered status under Ontario's Endangered Species Act of 2007, understanding the turgor loss point of the American chestnut is essential to predict seedling drought survival and support restoration efforts (Canada et al., 2019).
Effects of Temperature: The Heat Dispersion Mechanism in Chestnut Trees
Trees are generally considered to be ectothermic organisms, in that they lack the means to regulate their own temperature and therefore tend to maintain a similar temperature to that of their surrounding environment. The Castanea genus does not stray from that rule. For example, the Sweet Chestnut’s timber is orthotropic, always absorbing light and heat, and performing continuous water exchanges with its surroundings. Heat distribution in the timber of Chestnut trees depends on internal humidity and wood density, which are uneven across the tree’s trunk cross-section and unique to every individual, with the tree’s growth rings also playing a minor role. Moisture can have a large impact on the tree’s thermal diffusivity, such that dryer areas heat up more easily while more humid areas remain cooler (Borghese et al., 2024). By superimposing a wave phase vs. density profile over the thermography of wood timber samples with different treatments (Fig. 9), the impact of humidity on the tree’s internal temperature can be evaluated.

Fig. 9. Phase vs. density plots superimposed over thermography of three Sweet Chestnut samples. Sample (a) is a dried sample. Geometric thermal patterns correlate with density. Heat signatures correspond to growth rings, with other variations attributed to humidity. (b) is salified timber. Moisture distribution is stabler, and humidity plays a lesser role in distributing heat. (c) is new timber. Shows a gradient of thermal patterns generated by differences in density (adapted from Borghese et al., 2024).
The phase plot reproduces the fiber distribution. Humidity tends to accumulate where fibers are denser, affecting their heat capacity and resulting in the effects previously described. The trees remain cooler in rainy seasons and hotter when the climate is drier, keeping a generally stable temperature (Borghese et al., 2024). However, this internal heat distribution mechanism sometimes must work against very high and very low temperatures, as will be discussed next.
Same Species, Different Behaviors…
Given the plant’s ectothermic nature, large changes in external temperature, especially those caused by climate change, tend to affect its metabolism and the functioning of its leaf cells. The response to heat stress is not uniform among all Sweet Chestnuts, as individuals raised in different geographical locations (Fig. 10) display slightly different behaviors due to natural selection and genetic variability. Heat stress can increase the concentration of the amino acid proline in plant leaves (Fig. 11), which is an osmolyte that stabilizes protein structure and helps maintain membrane integrity. On the contrary, excessive proline accumulation is toxic and detrimental to some plants' thermotolerance, such as Arabidopsis thaliana (Dorado et al., 2022).

Fig. 10. Sweet Chestnut trees growing in (a) humid, (b) continental, and (c) xeric forests in Spain (Adapted from Dorado et al., 2022).

Fig. 11. Plot showcasing the increase of the proline amino acid in Sweet Chestnuts seedlings grown continuously under 44.5 °C for seven days (Dorado et al., 2022).
It is verifiable that only trees with the genetic profile of humid forests significantly increased proline production in comparison to the control group. Given how the European chestnut is prevalent over most of Europe (and how the genus Castanea has spread all over the world), some individuals from the same species have developed better heat stress tolerance than others. The climate in continental and xeric forests is much warmer, pushing for the selection of better responses to heat, unlike in the humid forests. Yet, after analyzing the biomass of each variant and comparing it to the control group, it was found that proline does not greatly impact the plant’s health, with a similar decrease in biomass observed in all strains after being continuously submitted to great heat (Dorado et al., 2022). In addition, it is possible to analyze the effects of temperature on the chestnut burr (Fig. 12) growth. Sweet Chestnut best develops its burr when rain is abundant, given its thermo-inhibitive effect, and temperatures are milder. Chestnut burr grows much more in milder weather conditions during seasons like fall and spring in comparison to harsher weather in the summer, which negatively affects burr growth. The exception to this would be the period comprising the end of Summer and the beginning of Fall, when, despite the high temperatures, the availability of water is increased and the trees are much more moist, and therefore cooler (Perulli et al., 2020).
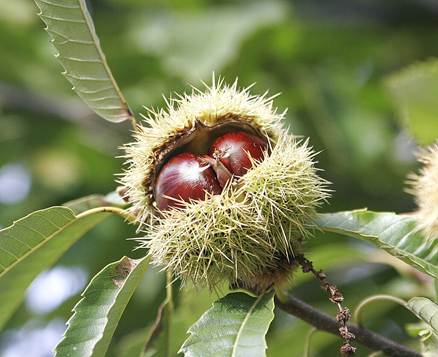
Fig. 12. Open Sweet Chestnut burr with chestnuts inside (Wikipedia, 2005).
Furthermore, not only do higher temperatures meddle with the species’ functioning, but so do colder temperatures. Sweet Chestnut suffers alterations to its circadian clock in colder temperatures. The plants, after detecting lesser periods of photoexposure during the winter, and especially after being submitted to temperatures as low as 4 °C, reach a state of endodormancy, which disrupts the canonical cyclic expression of at least five circadian oscillator genes, affecting overall development and growth (Ibañez et al., 2008).
Even without comparing to other variants of Chestnut trees, it is easy to see that within a single species, there is great variability and adaptability to diverse climatic conditions, as well as the unique thermal profile of each individual.
Mechanical Stress
Physical Properties
Similar to other hardwoods, such as oak, maple, and walnut, chestnut wood is a useful resource for timber. It has historically been used in castles, houses, roofs, and flooring, due to its high durability, good mechanical properties, and elegant appearance (Fig. 13). However, in the present day, large hardwood trees have become less accessible due to an imbalance in supply and demand. Although hardwoods are desirable for timber, their complex structure leads to a longer growth period than common softwoods. Some hardwood trees can take 150 years to grow before they are ready for harvesting, which is too long to keep up with the need for wood.

Fig. 13. Interior of the historic Cullisia Cabin, built in 1892 in Swain County, North Carolina and renovated in 2012 using the original American chestnut wood (Flannick, 2016).
To combat the long growth period of common wood materials, engineered wood products (EWPs) were developed from softwoods to create similar materials in a shorter time span. A common example is glue-laminated timber, also known as glulam, in which softwood is coated in glue to strengthen weaker sections. However, the low density of softwoods creates vulnerability during droughts and harsh weather, leading softwoods to be harshly affected by climate change. Sweet chestnut is one of the few tree species that sits in a grey area between soft and hardwood. It is classified as a hardwood, making it strong against environmental forces, but it sits in the C30 strength class, which is mostly reserved for softwoods (Fig. 14). The combination of hardwood and softwood properties makes this wood advantageous for use in glulam beams (Martins et al., 2025).

Fig. 14. Strength classifications for timber, adapted from Martins et al., 2025. Softwood is classified in the C-class from C14-C16. Hardwood is classified in the D-class from D30-D70. The number corresponds to the wood’s bending strength in MPa. Sweet chestnut is in the C30 class, which is rare for hardwood (Martins et al., 2025).
Sweet chestnut has a higher modulus of elasticity (13029 MPa) than other hardwoods, such as oak (10100 MPa) or beech (11627 MPa). This property measures the material’s stiffness at rest, implying how much resistance to deformation the wood will have under load. This is surprising for hardwood of low density, but it makes chestnut a useful material even before modification. However, the presence of ring shake and knots, discussed in further detail below, can make natural chestnut timber prone to damage (Fig. 15). When tested under bending stress, failures primarily occur at knots in the wood. Laminating the wood into glulam can significantly mitigate these weak points and make the wood more resilient (Martins et al., 2025). The tree’s softwood and hardwood properties make it a prime material for timber, and adding these small enhancements can make it even better. If the American chestnut is fully restored, it could be a very useful resource in the construction industry.

Fig. 15. Chestnut wood breaking under stress test. The failure occurred in the presence of a knot. These areas can create weak spots in the wood that are prone to breakage when used as timber (Martins et al., 2025).
Knots
Knots are imperfections in trees where failures under stress are most likely to occur (Fig. 16). They are formed when a branch grows from the tree, interrupting the natural grain pattern of the wood. A live knot occurs when the wood of the tree is harvested while the branch is still attached. Although their asymmetry reduces the strength of the wood, these knots have intact fibers and can still offer structural support. In contrast, dead knots form when a branch dies and falls off the tree, due to environmental forces or disease, and new layers of the tree grow around it. These spots are weak and often lead to breakage under stress. However, knots are often desired in wood planks due to their uniqueness and aesthetic appeal (Chang & Lin, 2021).
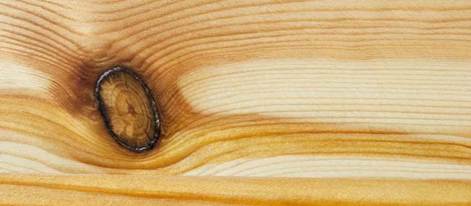
Fig. 16. A knot in a sample of wood. Although it adds to the natural appearance of the wood, it can significantly affect the structural integrity (Smith, 2025).
Ring Shake
Chestnut trees are especially prone to ring shake, a circular defect formed in the tissue of the tree’s trunk between two growth rings, which reduces the wood’s strength and increases likelihood of failure under stress (Fig. 17). The condition develops in the tangential plane of the tree trunk (Fig. 18) and leads to internal cracks and delamination (fractures between layers of tissue) due to growth, drying, or environmental stresses (Kakavas et al., 2018). Chestnut wood has two main structural weaknesses in its anatomy that make ring shake so prominent. The wood is ring-porous, forming fragile planes where shakes can form under minor stress, and is congested with reinforcing wood rays, leading to structural consequences when the stress is redistributed in the tree (Fonti et al., 2002). Ring shakes are often concealed from the outside and require further testing to be detected, which can be an economic burden. It increases variability in the mechanical behavior of the tree, making its strength, stiffness, and elasticity less consistent between various samples (Romagnoli & Spina, 2012).

Fig. 17. Example of ring shake in a sweet chestnut tree. The circular crack running parallel to the growth rings is a severe case of ring shake and drastically affects the strength of the timber (Schwab, 2018).

Fig. 18. Direction terminology used throughout the essay for describing ring shake. The radial direction points outwards from the core, the tangential direction points along the growth ring, and the axial direction points along the trunk (Ashby & Jones, 2013).
Since chestnut is a ring-porous material, its risk of shakes is increased by the wood’s weak points between growth rings. Ring-porosity refers to the distinctly larger xylem vessels (used for transport of water) being found in the earlywood (Fig. 19), the wood grown during the first part of the tree’s annual growth cycle. The excessive xylem makes the trunk less dense in these sections, creating a natural weak zone where ring shakes are more likely to occur (Fonti et al., 2002). This risk is especially present when growth stresses, permanent stresses from internal mechanical forces supporting the growth of the tree, are applied to the wood in the radial direction. Growth stress results from two mechanisms, namely cell wall maturation and an increase in dead weight. As the cell wall reaches the last stage of its formation, new xylem fibers tend to deform in axial and transversal directions. This deformation is restricted by the original xylem, inducing stress on the outermost surface of the new xylem and provoking a counteractive stress on the older xylem. As the tree grows and dead weight increases, the older part of the trunk takes on this stress. Each stage of growth provides additional stress distribution to balance the tree against gravitational forces (Gril et al., 2017). This stress reinforces the tree, but too much growth or environmental stress will result in ring shake. The defect is also normally found in the central part of the stem radius, where growth stresses are higher (Fonti et al., 2002).

Fig. 19. Cross-sectional photo of four rings on the sweet chestnut. The lighter, porous areas are the earlywood, and the darker, solid areas above them are the latewood. The light vertical lines seen in the late wood are wood rays (Schwab, 2018).
Another property that affects the mechanics of chestnut wood is the ray volume. Wood rays are tissues in the wood running perpendicular to growth rings. They are lines of living cells that serve as vital storage and transport for water, nutrients, and carbohydrates, while also acting as a reinforcement tissue that improves the resistance of wood against radial tensile stress. When there is higher internal stress in the trunk of the tree, it will produce more rays as a response. The rays tend to be much stiffer and stronger in the radial direction than the surrounding tissues. If the strength of the tree outweighs the stresses, the tree will be healthy and stable. However, in chestnut wood, the rays act as both a reinforcement and a structural point of weakness, depending on the direction of the load. An increased number of rays signifies that the tree has experienced more growth stresses, meaning the tree is prone to ring shake. When the tree falls, the force of gravity is no longer a demanding force on the trunk of the tree, and the stresses redistribute. The trees with a higher ray count will be more likely to develop ring shake because there is more stress present in the tree, and the rays no longer act against the force. In the tangential direction, the rays are not a reinforcement but rather an indication of the amount of internal stress on the tree. Once the stress outweighs the strength, the tree will be susceptible to shakes (Fonti & Frey, 2002).
The ring-porosity, ray volume, and other temporary loads, such as wind and frost, can all lead to ring shake in chestnut wood, making the material undesirable for use as a construction material. However, ring shake can also lead to wood with lower wood shrinkage. Shrinkage occurs when the dimensions of the wood change after drying, and it can be troublesome in commercial use because the measured timber may fit differently upon application. Shakes result in internal separations that relieve stress and allow for some movement in the mechanical system between rings, reducing the whole-disk shrinkage in the wood (Romagnoli & Spina, 2012).
Symbiotic Relationships
Ectomycorrhizal (ECM) Mutualism
Direct physical interactions with various organisms benefit the chestnut tree in terms of growth, structural strength, and external protection. Chinese chestnut is particularly known to form a symbiotic relationship called ectomycorrhiza (ECM), an interaction occurring between the roots of the tree and certain fungi. Moreover, as the term “mycorrhizal” suggests, the mutual symbiotic relationship developed between the tree and the fungus is beneficial for both species (Tikhonovich & Provorov, 2007). Typically, ectomycorrhizas are distinguished by their unique physical structure, the fungal mantle (thick outer layer) enveloping the host roots. This particularity increases the surface area needed for resource exchange (Johnson & Gehring, 2007). The word itself comes from “myco,” meaning “fungus,” and “rhiza,” meaning root. This translates to root fungi (Volk, 2001). ECM symbiosis modifies the tip of the root structure (Chen et al., 2025). By placing itself around the root tips, ECM fungi contribute to the absorption of nutrients and water. The tree provides products of photosynthesis (Xiong et al., 2025).
A study was conducted to investigate the effect of exposure of ECM fungi Pisolithus orientalis (Po) and Cenococcum geophilum (Cg) on chestnut seedlings. Root growth and nutrient levels of nitrogen, potassium, and carbon, three nutrients are important for plant growth and development (Jiaying et al., 2022), were measured. To test this, sterilized chestnut seeds were grown in a soil mixture under three treatments: inoculation with Cg, inoculation with Po, and a non-inoculated control. After six months of growth, the results showed that inoculation with Cg and Po promoted growth. This symbiotic relationship led to higher levels of nitrogen, phosphorus, and potassium in the shoots (Fig. 20). It also led to overall root development, especially in developing fine roots of the Chinese chestnut (Chen et al., 2025).

Fig. 20. Bar Graph of Shoot concentrations of Nitrogen, Phosphorus, and Potassium in Chinese chestnut (A–C) seedlings that were inoculated with Cenococcum geophilum (Cg) and Pisolithus orientalis (Po) after six months, modified from Chen 2025. Contents per plant were measured in milligrams (mg). Values were compared among three treatments: inoculation with Cenococcum geophilum (Cg), inoculation with Pisolithus orientalis (Po), and a non-inoculated control (Con). Distinct lowercase letters denote significant differences among treatments within the same host species (p < 0.05) (Chen et al., 2025).
Another study investigated the impact of ECM fungi symbiosis on chestnut trees’ growth, root development, and phosphorus nutrient acquisition. Again, two Castanea henryi seedlings were inoculated with ECM fungi, and two were used as control samples. The results, as seen in Figure 21, demonstrated that the ECM fungi increased root production, phosphorus absorption, and plant growth of the Castanea henryi (Xiong et al., 2025).

Fig. 21. Growth, root development, and phosphorus (P) uptake of Castanea henryi’s seedlings inoculated with ECM Fungi (JG) compared to the control sample (CK). Samples that were inoculated with ECM fungi (JG) are seen to have grown taller, have greener leaves, developed more roots, and have a higher P content above and below ground compared to control seedlings, which were not inoculated with ECM fungi. (A) Comparison of growth and leaf color. (B) Root development. (C) is a closer picture of the root system, and (D) Cross-section of stems of Castanea henryi. (E) Total phosphorus (P) content (mg-1) above and below ground (Xiong et al., 2025).
Another benefit from the ECM symbiosis is that the fungi enhance the root’s resistance to pathogens, such as Phytophthora root rot. The fungi modify root structure and provide protection to the roots by forming a physical barrier and activating the plant’s defense mechanisms. For example, the plant responds by producing tannin compounds, which are antimicrobial and act as a chemical barrier against pathogens (Huang et al., 2024) (Zheng et al., 2024). Moreover, by increasing the root’s absorption capacity of mineral elements, the plant gains more resources, which support stronger defense systems. These defenses can be physical, such as thicker tissues and the production of protective waxes (Lombardero et al., 2022). In addition, ECM fungi strengthen plants’ ability to withstand dry conditions (Xiong et al., 2025). This is due to the mycelium networks that allow different trees of different ages to be connected, which allows them to exchange nutrients to those in need (Holewinski, n.d.). Therefore, the area of the tree’s absorption increases.
Overall, ectomycorrhizal symbiosis between fungi and chestnut tree roots allows the tree to increase its nutrient uptake, root development, drought tolerance, and pathogen resistance. This relationship supports healthier growth and long-term survival of the chestnut tree.
Seed Hoarders Mutualism
After the blight that substantially declined the American chestnut population, few fully grown chestnut trees remain in the area. A critical mechanism for the revival is the seed dispersal mutualism between animals and the trees, which helps spread the seeds to new areas and increases their potential to thrive. This process is dependent on the physical properties of the chestnut, such as the size and thickness, as that determines which chestnut the animal selects. The animal selects the nuts as they create their winter stock, but often some get left behind and dispersed in the process. The location at which they cache their food can be farther than the parent tree, avoiding competition and seed predation (Wright et al., 2022). If forgotten at these secret sites, the seeds can then germinate under suitable conditions, leading to new chestnut trees and ensuring their survival. The ideal properties of nut selection differ by the animal. Medium sized birds, including woodpeckers and blue jays, prefer chestnuts with a flattened shape, as this allows their smaller bills to hold them better. In contrast, the titmouse, a smaller bird, prefers chestnuts with a thinner shell as this makes them lighter. The titmouse is too small to hold the nut in its beak, so instead it grabs onto the remaining flower stem. A lighter chestnut is less likely to snap off, increasing the efficiency of the collection process. In general, most of the species evolved for a thinner shell, as that makes it easier for them to break into the shell. As restoration efforts continue for the chestnut blight, it is important that considerations on chestnut size and thickness are considered when selecting seeds from parent trees, as that will determine the rate at which the seeds get spread (Matthews et al., 2022). So, this mutualistic relationship does not only facilitate effective seed dispersal for chestnut trees but also provides a reliable food source for the animals. This highlights the interconnected benefits of both organisms.
Wasp Parasitism
The Asian chestnut gall wasp (ACGW) (Dryokosmus kuriphilus Yasumatsu) is originally from China but spread to different countries through the introduction of chestnut trees carrying infested galls (Labbate & McCullugh, 2021). Their attack on European chestnut (Castanea sativa Mill) became a serious issue due to the wasps’ life cycle being synchronized with the tree’s phenology (Marcolin et al., 2021) They are considered the primary parasite of chestnut trees because the wasps benefit from the host tree and harm it. This relationship leads to a decrease in the tree’s growth and in nut production (Labbate & McCullugh, 2021). Moreover, chestnut stomata lose capacity to control gas-exchange, resulting in a decline of bud development. This causes branch deformity, crown deterioration, and green biomass reduction. The decrease in tree-ring growth rate leads to a loss of timber biomass and heightens the risk of ring shake. Together, these effects impact timber production and quality (Marcolin et al., 2021). The mechanism responsible for this involves the wasps depositing their eggs inside chestnut buds at the end of summer, with the larvae only hatching in the spring (Labbate & McCullugh, 2021). This is when the tree starts leaf production. The larvae take advantage and start feeding, a behavior that contributes to small gall growth on the tree’s shoot and leaves, depleting the resources of the host that would be otherwise available for its own growth, development, and regeneration (Fig. 22).

Fig. 22. Leaf galls on chestnut shoot resulting from induced by Asian chestnut gall wasp (Labbate & McCullugh, 2021).
In summary, Asian chestnut gall wasps are parasites of chestnut trees. They grow inside the buds, causing several negative effects on the trees’ health, such as the increase in ring shake and the decrease in timber quality.
Conclusion
Despite a blight severely affecting the American chestnut population in the 20th century, the chestnut tree still holds cultural and environmental significance across the world. The principles of classical physics, such as pressure, strength, and stress, can explain the potential of various chestnut species as a timber resource, mutualistic partner, and reference for the restoration of the American chestnut. Turgor pressure plays an important role in plant growth and is severely affected by environmental forces. A comparison of the American and Chinese chestnut showed their different responses to drought and revealed the limitations of the American species. Chestnut trees struggle to reproduce due to the unlikelihood that the pollen of one tree will reach the female flower of another. However, the tree utilizes the movement of common flower dwellers, the beetle, to spread their pollen to other locations. Gravity applies a constant pressure to the tree as it grows, but the wood rays in the tree help increase its strength and tolerance. Nutrients and water can be scarce in the tree’s immobile position, but a symbiotic relationship with the ECM fungi helps them absorb nutrients in return for their photosynthetic products. Many animals rely on the chestnut for food, and their consumption helps spread the chestnut seeds to new locations. The nut maximizes this relationship by evolving a thin shell for animals to easily carry and break into. The chestnut tree has experienced many perils to blight and ring shake, but its fascinating physical properties, responses to stress, and partnerships demonstrate how nature can create innovative design solutions and make chestnut wood an advantageous resource for many industries.
References
References
Álvarez-Cansino, L., Comita, L. S., Jones, F. A., Manzané-Pinzón, E., Browne, L., & Engelbrecht, B. M. J. (2022). Turgor loss point predicts survival responses to experimental and natural drought in tropical tree seedlings. Ecology, 103(6), e3700. https://doi.org/10.1002/ecy.3700
Blackman, C. J. (2018). Leaf turgor loss as a predictor of plant drought response strategies. Tree Physiology, 38(5), 655-657. https://doi.org/10.1093/treephys/tpy047
Buchner, R., Halbritter, H., Heigl, H., Sam, S. (2020). Castanea sativa. https://www.paldat.org/pub/Castanea_sativa/303767
Borghese, V., Santoro, L., Santini, S., & Sesana, R. (2024). Correlation between thermal and density properties of chestnuts: preliminary results of experimental non-destructive testing. Archives of Civil and Mechanical Engineering, 24(3), 157. https://doi.org/10.1007/s43452-024-00969-8
Canada, E., Climate Change, C., & Committee on the Status of Endangered Wildlife in, C. (2019). Recovery strategy for the American chestnut (Castanea dentata) in Canada. Environment and Climate Change Canada. http://epe.lac-bac.gc.ca/100/201/301/weekly_acquisitions_list-ef/2019/19-07/publications.gc.ca/collections/collection_2019/eccc/En3-4-295-2019-eng.pdf
Chang, C.-W., & Lin, F.-C. (2021). Strain concentration effects of wood knots under longitudinal tension obtained through digital image correlation. Biosystems Engineering, 212, 290–301. https://doi.org/10.1016/j.biosystemseng.2021.10.014
Chen, T., Zhu, C., Li, S., Xia, Y., Huang, J., Wang, W., Lian, C., Chen, Y., Zhao, Y., & Zhang, S. (2025). Impact of ectomycorrhizal symbiosis on root system architecture and nutrient absorption in Chinese chestnut and pecan seedlings. Plant and Soil. https://doi.org/10.1007/s11104-025-07332-7
Di-Giovanni, F., Kevan, P. G., & Nasr, M. E. (1995). The variability in settling velocities of some pollen and spores. GRANA -STOCKHOLM-, 34(1), 39.
Dorado, F. J., Solla, A., Alcaide, F., & Martín, M. Á. (2022). Assessing heat stress tolerance in Castanea sativa. Forestry: An International Journal of Forest Research, 95(5), 667-677. https://doi.org/10.1093/forestry/cpac021
Farrell, C., Szota, C., & Arndt, S. K. (2017). Does the turgor loss point characterize drought response in dryland plants? Plant Cell Environ, 40(8), 1500-1511. https://doi.org/10.1111/pce.12948
Flannick, J. (2016, October 28). Home of the week: Rare chestnut cabin in Swain. The Asheville Citizen Times. https://www.citizen-times.com/picture-gallery/life/home-garden/2016/10/27/home-of-the-week-rare-chestnut-cabin-in-swain/92821724/
Franklin, J. (2012). Castanea Mollissima Blume (Chinese Chestnut), Growth Habit, Tree Form. [Digital Color Photograph]. The Morton Arboretum, Lisle, IL, United States. https://acorn.mortonarb.org/Detail/objects/76666
Fredericksen, B., Kukor, S., & Rosenthal, D. M. (2021). Physiological changes in advanced hybrid chestnuts do not alter blight resistance under co-occurring drought. Canadian Journal of Forest Research, 51(11), 1678-1687. https://doi.org/10.1139/cjfr-2020-0505
Holewinski, B. (n.d.). Underground Networking: The Amazing Connections Beneath Your Feet. National Forest Foundation. https://www.nationalforests.org/blog/underground-mycorrhizal-network
Hosh, B., Ghosh, P.K., Roy, S., Hossain, Z., Gupta, S., Adak, M.K., Sarkar, S.N. (2017). POST GRADUATE DEGREE PROGRAMME (CBCS) IN BOTANY [Self-Learning Material]. University of Kalyani. https://dodl.klyuniv.ac.in/download/DODL%20M.A_M.Sc%20SLMs/DODL_M.A_M.Sc_%20SLMs_%20SEM-II/SLM_botany_Sem-II.pdf
Ibañez, C., Ramos, A., Acebo, P., Contreras, A., Casado, R., Allona, I., & Aragoncillo, C. (2008). Overall alteration of circadian clock gene expression in the chestnut cold response. PLoS One, 3(10), e3567.
Jiaying, M., Tingting, C., Jie, L., Weimeng, F., Baohua, F., Guangyan, L., Hubo, L., Juncai, L., Zhihai, W., Longxing, T., & Guanfu, F. (2022). Functions of Nitrogen, Phosphorus and Potassium in Energy Status and Their Influences on Rice Growth and Development. Rice Science, 29(2), 166-178. https://doi.org/10.1016/j.rsci.2022.01.005
Johnson, N. C., & Gehring, C. A. (2007). CHAPTER 4 - Mycorrhizas: Symbiotic Mediators of Rhizosphere and Ecosystem Processes. In Z. G. Cardon & J. L. Whitbeck (Eds.), The Rhizosphere (pp. 73-100). Academic Press. https://doi.org/10.1016/B978-012088775-0/50006-9
Kane, J. M., Varner, J. M., Stambaugh, M. C., & Saunders, M. R. (2020). Reconsidering the fire ecology of the iconic American chestnut. Ecosphere, 11(10). https://doi.org/10.1002/ecs2.3267
Larue, C., & Petit, R. J. (2024). Insect pollination in chestnut: an organized mess? Acta Horticulturae(1400), 331-340. https://doi.org/10.17660/ActaHortic.2024.1400.40
Marcolin, E., Pividori, M., Colombari, F., Manetti, M. C., Pelleri, F., Conedera, M., & Gehring, E. (2021). Impact of the Asian gall wasp Dryocosmus kuriphilus on the radial growth of the European chestnut Castanea sativa. Journal of Applied Ecology, 58(6), 1212-1224. https://doi.org/10.1111/1365-2664.13861
Martins, C., Ferreira, C., Monteiro, S. R., & Dias, A. M. (2025). Mechanical properties of sweet chestnut sawn wood and glulam performance. European Journal of Wood and Wood Products, 83(3). https://doi.org/10.1007/s00107-025-02266-4
Miller, A., Miller, D.D., Pijut P. M. (2014). How a Flower Becomes a Chestnut: Morphological Development of Chinese Chestnuts (Castanea mollissima) [Scientific article]. The Journal of the American Chestnut Foundation, 13-18. https://ohioline.osu.edu/sites/ohioline/files/imce/Plant_Pathology/PLPATH-FRU-0051-FlowertoChestnut.pdf
Perulli, G. D., Boini, A., Bresilla, K., Morandi, B., Grappadelli, L. C., & Manfrini, L. (2020). Growth analysis of sweet chestnut burr in two seasons with differing weather conditions. Italus Hortus, 27(1), 31-39.
Petit, R. J., & Larue, C. (2022). Confirmation that chestnuts are insect-pollinated. Botany Letters, 169(3), 370-374. https://doi.org/10.1080/23818107.2022.2088612
Qiu, Q., Tian, X., Wu, G., Wu, J., Yuan, D., & Fan, X. (2025). Basis of single-seed formation in chestnut: cytomorphological observations reveal ovule developmental patterns of Castanea henryi. PeerJ, 13, e18711. https://doi.org/10.7717/peerj.18711
Revord, R., Gold, M., Meier, N., Webber, B., Hunt, K., Warmund, M. (2022). GROWING AND MARKETING
Schwendemann, A. B., Wang, G., Mertz, M. L., McWilliams, R. T., Thatcher, S. L., & Osborn, J. M. (2007). Aerodynamics of saccate pollen and its implications for wind pollination. American Journal of Botany, 94(8), 1371-1381. https://doi.org/10.3732/ajb.94.8.1371
Sharma, A., Shahzad, B., Kumar, V., Kohli, S. K., Sidhu, G. P. S., Bali, A. S., Handa, N., Kapoor, D., Bhardwaj, R., & Zheng, B. (2019). Phytohormones Regulate Accumulation of Osmolytes Under Abiotic Stress. Biomolecules, 9(7). https://doi.org/10.3390/biom9070285
Smith, R. (2025, July 29). The Pros and Cons of Knots in Wood. Wagner Meters. https://www.wagnermeters.com/moisture-meters/wood-info/pros-cons-knots-in-wood/
Snowsill, W. L. (2010). Chapter 16 - Particle Sizing. In W. Boyes (Ed.), Instrumentation Reference Book (Fourth Edition) (pp. 175-189). Butterworth-Heinemann. https://doi.org/10.1016/B978-0-7506-8308-1.00016-4
Su, R., Liu, H., Wang, C., Zhang, H., & Cui, J. (2022). Leaf turgor loss point is one of the best predictors of drought-induced tree mortality in tropical forest. Frontiers in Ecology and Evolution, 10. https://doi.org/10.3389/fevo.2022.974004
The American Chestnut Foundation. (n.d.). Chestnut Species Overview. https://tacf.org/identification/chestnut-species/
Tikhonovich, I. A., & Provorov, N. A. (2007). Chapter 14 - Beneficial plant–microbe interactions. In Y. T. Dyakov, V. G. Dzhavakhiya, & T. Korpela (Eds.), Comprehensive and Molecular Phytopathology (pp. 365-420). Elsevier. https://doi.org/10.1016/B978-044452132-3/50018-3
Timerman, D., & Barrett, S. C. H. (2021). The biomechanics of pollen release: new perspectives on the evolution of wind pollination in angiosperms. Biological reviews of the Cambridge Philosophical Society, 96(5), 2146-2163. https://doi.org/10.1111/brv.12745
Westbrook, J. W., Holliday, J. A., Newhouse, A. E., & Powell, W. A. (2020). A plan to diversify a transgenic blight-tolerant American chestnut population using citizen science. Plants, People, Planet, 2(1), 84-95. https://doi.org/10.1002/ppp3.10061
Wikipedia. (2005). [Chestnuts]. Retrieved 10/03/2025 from https://en.wikipedia.org/wiki/File:Chestnuts.jpg

Xiong, H., Yu, S.-Y., Zou, F., & Yuan, D.-Y. (2025). 2 - Symbiosis of ectomycorrhizal fungi with Castanea. In Q.-S. Wu (Ed.), Management of Mycorrhizal Symbiosis for Mycoremediation and Phytostabilization (pp. 9-28). Elsevier. https://doi.org/10.1016/B978-0-443-24863-4.00002-9
Zhang, X., Ramakanth, K. K., & Long, Y. (2024). The biomechanics of turgor pressure. Current Biology, 34(20), R986-R991. https://doi.org/10.1016/j.cub.2024.07.013