Table of Contents
Keywords: Hevea brasiliensis, fruits, explosive dehiscence, root system, photosynthesis, leaves, structure, layers, latex flow.
Abstract
The Hevea brasiliensis is commercially very important. Although it is more known for all the ways it is useful to humans, the tree is also very efficient at providing itself with design solutions that help it thrive in its own environment. This paper highlights firstly how H. brasiliensis undergoes reproduction in a unique way using explosive dehiscence examined under a physics lens. Secondly, its strong root and anchorage system which allows it to grow tall while not falling over. Continued, by the energy distribution in the leaves of the tree which results in the tree still being able to perform photosynthesis at all levels. Finally, this paper will look into the laticiferous system and physiology of latex flow. Inspired by the physics behind H. brasiliensis from each of these four processes, this essay offers a few design solutions for the H. brasiliensis’ tree to overcome some of the challenges it faces due to nature and its environment.
Introduction
Hevea brasiliensis is a tree originating from the upper Rio Madeira region of Brazil, within the Amazon River Basin. As a suggestion by Sir Clement Markham of the British India Office, it was exported to many Southeast Asian countries (Table 1) starting in June 1876 for its latex (Priyadarshan et al., 2017), a key ingredient of natural rubber. H. brasiliensis now represents 95% of the world’s rubber production.
Table 1: Natural rubber production (in million metric tons) in Asian countries against the world in 2012 and 2013 (Priyadarshan et al., 2017).
| Country | 2012 | 2013 |
|---|---|---|
| Bangladesh | 0.18 | 0.19 |
| Cambodia | 0.64 | 0.85 |
| China | 0.8 | 0.86 |
| India | 0.91 | 0.7 |
| Indonesia | 3.0 | 3.2 |
| Laos | 0.07 | 0.08 |
| Malaysia | 0.92 | 0.82 |
| Myanmar | 0.013 | 0.14 |
| Papua New Guinea | 0.075 | 0.075 |
| Philippines | 0.11 | 0.11 |
| Sri Lanka | 0.15 | 0.13 |
| Thailand | 3.8 | 4.17 |
| Vietnam | 0.8 | 0.9 |
| Asia total | 10.85 | 12.15 |
| World total | 11.6 | 12.22 |
H. brasiliensis belongs to the Euphorbiaceae family, and to the Hevea genus, that assembles more than 10 different variations of Hevea trees with which it is capable of recombination. It diverged from them approximately 3.77 million years ago, making it a rather recent, compared to oak tree that has 56 million years of history (Fang et al., 2024).
H. brasiliensis possesses a straight trunk with an open leafy crown. Like other Hevea species, it has tri-foliated leaves, as well as greenish-yellow, petal-less flowers. It can be as tall as 40 m and has a lifespan of 100 years in the wild, though domesticated rubber trees tend to be limited to 30 m due to the regular harvest of their latex and are replanted every 30 years. This Hevea species is a monoecious plant that is predominantly cross-fertilized by insects. Its strongly scented flowers mostly attract midges, ants and thrips, that carry triangular pollen grains within a radius of 0.3 to 1.1 km. The pollination of a population of H. brasiliensis can be slightly reduced by rain. It reaches physiological maturity and ripeness to flower after 4-5 years. However, latex maturity is only attained once its trunk has a girth of 50 cm and a height of 125 cm, adding 2-3 years of wait for a total of 6-7 years.

Fig. 1. H. brasiliensis being tapped in a Malaysian plantation near Kuala Lumpur (Schultz et al., 2025).
As a tropical tree, H. brasiliensis has to compete with a myriad of other beings in its natural habitat. Through evolution, it has adapted to obstacles to its growth within the Amazonian canopy by taking advantage of various mechanics of physics. Indeed, its reproduction, germination process through explosive dehiscence allows it to enjoy relatively empty growth spaces. H. brasiliensis is also able to reach the highest levels of the canopy and efficiently receive sunlight to produce energy through photosynthesis using its peculiarly structured and layered root and leaf systems. The former provides sufficient stability and anchorage to the ground to prevent uprooting, while the latter is carefully organized to maximize sunlight interception, even in the lower echelons of the canopy. Finally, the turgor pressure that guides the latex through the organism operates as a defense mechanism that preserves the integrity of the tree.
Reproduction
The Physics of the Fruit and Seed
The Hevea brasiliensis tree commences its fruit production at the age of 4 (Baidya et al., 2023). Once fertilization has occurred, the ovary of the flower develops into a three-lobed, dehiscent fruit which contains three large, ovoid-shaped seeds (Priyadarshan et al., 2017). The fruit is referred to as a regma and can be observed in Fig. 1 below.

Fig. 2. Fruit of Hevea brasiliensis still attached to the tree (Balasubramanian, 2023)
Mature fruits that contain less than three seeds are rare which suggests that all three ovules of the female flower has to form seeds for the fruit to develop to maturity. Therefore, signifying for fruit development, pollen must germinate on all three of the stigmas of a flower.
Each seed within the fruit, an ellipsoidal capsule, typically has a mass between 3.5 and 6 g in which the endosperm comprises around 50 to 60 percent of this mass. The seed's coat is hard and shiny, usually entirely brown or with shades of grey. There are several darker pigmentations on its dorsal side, and the ventral side of the seed is slightly flattened (Priyadarshan et al., 2017). Figure 3 demonstrates the exterior of the seed.

Fig. 3. Hevea brasiliensis fruit opened exposing the seed (Bakewell-Stone, 2025).
Twenty to twenty-four weeks after pollination has occurred, the ripe and dry fruit will fall from the tree and will explosively dehisce. The endocarp encasing the seeds splits into six pieces. The seeds get dispersed to a distance of around 15 meters from the tree (Priyadarshan et al., 2017). When close to a river the seeds will often explode into the rivers that are present under the tree. The seeds can then be carried over a longer distance until they reach an area that is suitable for germination such as areas that have high light exposures. In areas where there are not any rivers, the result is a high density of seeds under the tree (Zhou et al., 2015). Each tree produces around 800 seeds during two periods throughout the year (Baidya et al., 2023).
Mechanics of Explosive Dehiscence
During the process of explosive dehiscence, the three valves of H. brasiliensis coil rapidly expelling the seeds. Energy stored in the walls is swiftly transferred to the seeds where it is transformed into kinetic energy. The amount of energy stored in the walls is related to the level of hydration. Elastic energy is obtained through the physical breaking of bonds. When the fruit dehydrates, it shrivels, increasing bending stress and eventually cracking. The bonds then break by the fruit undergoing a fast-moving crack. Something to note is that the cracks also consume energy and therefore limit the amount of stored energy (Deegan, 2012).
The distance the seeds get dispelled to depends on a few factors which are the seed mass, the interaction between the seed and air, and their launch trajectory. There is therefore an optimal launch angle in order to maximize the distance in which the seeds get projected which consequently depends on the factors mentioned (Hayashi et al., 2009).
The resultant velocity of the seed can be calculated using the following formulas. In equation 1, vvx and vvy the components of the velocity (vv) within the vertical plane (Hayashi et al., 2009).

In equation 2, the resultant velocity in the horizontal plane can be calculated by using the following formula (Hayashi et al., 2009).

Here, vhx and vhy are the components of the horizontal velocity. Finally, to calculate the resultant velocity the following formula can be applied (Hayashi et al., 2009).
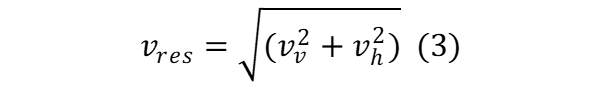
The angle the seed is getting launched at, also known as the launch angle (θ) can be calculated using equation 4 below (Hayashi et al., 2009).

Germination
The seed is initially dry when it comes in contact with soil. The seed coat of a H. brasiliensis is hard and allows for the slow entry of water through diffusion and capillary motion, which delays germination and slows the imbibition time. The process of imbibition occurs in three phases. Firstly, during phase I, the seed undergoes a fast uptake of water causing the tissues to swell and increasing the turgor pressure. Phase II includes the activation of metabolism and a slowdown in the absorption of water into the cell tissues. The final phase of imbibition is once again the fast uptake of water which causes swelling and allows the roots to break the seed coat. A study was done where the imbibition process was observed and put into a graph, this can be observed in Fig. 3 below (de Carvalho JC et al., 2022).

Fig. 4. Imbibition curve of H. brasiliensis of cultivated (⭘) and wild (⏺) seeds with arrows indicating the emergence of root primordia. (b) The changes in seed mass over time of wild and cultivated seeds of H. brasiliensis (de Carvalho JC et al., 2022).
The physics the H. brasiliensis tree uses in order to thrive in its environment can be applied for improving technologies today. For instance, controlled cracking involves designing materials that predictably crack in a certain way which will ensure that if the material is to crack or fail it does so in a safe way. This would be needed in situations where structural failure is not avoidable and would be beneficial if it occurred safely. This would mimic how H. brasiliensis cracks to explosively expel its seeds. Another example is drug delivery capsules which crack under certain conditions or environments within the body such as pH change or certain concentrations of substances. This would mimic how the seeds explosively dehisce when they reach a critical hydration level, storing and releasing energy at the right moment. This will make it possible to provide medication to the place that needs it most.
Structure of Hevea brasiliensis: Anchorage and the Root System
Challenges to Growth
In its natural habitat, the Amazon River Basin, H. brasiliensis faces a competitive environment for energy and harsh climatic conditions. An incredibly abundant flora, consisting even of trees capable of reaching above 100 m, is omnipresent in these regions of South America: a single acre has been known to contain over a hundred non-recurring species of trees. The Amazonian canopy, as the top layer of the layered structure of the rainforest, rising to 40 m, with some exceptions called “emergent trees” that go up to 70 m, creates an absolute need for height to access sunlight (Schultz et al., 2025). The Amazon River Basin is subject to heavy rainfall, winds and frequent floods in the floodplains. For high-reaching trees like H. brasiliensis, maintaining a straight shape to attain the sunlight and staying anchored becomes a biological challenge of survival. Many trees in the same basin have large buttresses or enlarge the basal portions of their trunk, like the Bertholletia excelsa (the Brazil Nut) (Priyadarshan, 2017). However, the H. brasiliensis, lacking those features, has developed an extensive root system as a solution for the harsh conditions of the Amazon River Basin by providing great anchorage and resistance to lateral above-ground stresses.
H. brasiliensis’ Root System
This species of Hevea sits at the intersection of multiple main root system morphologies. This intermediate morphology (Stachew et al., 2021) consists of joining a taproot system and a lateral root system together. Combined so, they provide sufficient mechanical support and nutrient absorption to meet the needs of the tree.

Fig. 5. Different types of typical root systems (not including H. brasiliensis’), (Ding et al., 2022).
Taproot systems are characterized by central, straight, vertical roots. In contrast, lateral root systems, or the “plate morphology”, grow lateral roots horizontally and slightly obliquely downwards from the base of the trunk. These lateral roots can branch into new roots, or into vertical sinker roots. (Fig. 5) H. brasiliensis possesses multiple taproots, and extensive lateral roots that branch within 30 cm of the ground from those taproots, reaching much farther than the spread of the branches. While there are lateral roots up to 80 cm under the surface, these do not reach as far.
In deep soil, with no obstacles to root growth and elongation, a 3-year-old H. brasiliensis has taproots burrowing around 1.5m from the surface, and laterals branching 6 to 9 m from the base of the tree and a 7-year-old Hevea, 2.4m taproots, and 9 m laterals. The roots spread rapidly after germination in order to provide sufficient anchorage and nutrient absorption for this fast-growing tree (Priyadarshan, 2017). Compared to the Mallotus Wrayi, whose taproot at maturity extends to 1.4 m, with a rigid part at 0.5 m, H. brasiliensis possesses a very fast-growing taproot (Crook & Ennos 1998).
The root system represents roughly 15% of the total dry weight of a mature tree, for around 6-8% of the total tree size. This concentrated mass at the base of the Hevea provides a lower center of gravity for the tree, improving its stability. This is a common design solution for trees, that prevents toppling caused by the weight of the branches or weak lateral stresses (Priyadarshan, 2017).
The Taproots’ Role
Considering the fast-growing nature of H. brasiliensis, it is essential for it to find strong anchorage as soon as possible. The taproots of the H. brasiliensis can provide that. With a very rapid elongation rate in the first 6 months of growth of 9.43 +/- 0.6 mm/day (Fig. 7), the taproots can reach around 60% of their maximum length within that period (Carron et al., 2000). The taproot then provides, at a very young age, the H. brasiliensis with a rigid element to prevent immediate uprooting (Fig.6). This is especially true when you consider the failed cuttings of the best part of the 20th century. With this process, rubber research institutes were not able to achieve complete reproduction of the Hevea root systems for their regenerated trees. Lacking a taproot, these trees were frequently uprooted by strong winds before yielding latex, reinforcing the importance of the taproot during early growth (Carron et al., 2000).

Fig. 6. Taproot of a one-year-old PR 107 H. brasiliensis clone (Carron et al., 2000).

Fig. 7. Measuring the length of the taproot system on 50 trees in the first two years of growth in the field (Carron et al., 2000).
Studies of other trees indicate that while taproots play a major role in the anchorage of young trees, its usefulness declines with growth. Crook & Ennos (1998) have studied the Mallotus wrayi, also of the Euphorbiceae, for its rather simplistic model of a single taproot in the soil. Results show that many tall trees fail mechanically under lateral stress due to the taproot pushing the soil. Moreover, they conclude that as tall standing trees grow taller, there is an increased chance that it will fall over, therefore making trees taller than M. wrayi almost incapable of creating a taproot allowing near full anchorage. H. brasiliensis, being double the size of this tree, necessitates additional roots to keep it stable. However, the taproots’ influence on anchorage does not stop here.
In H. brasiliensis, the taproot grows deeper than the lateral roots (see “The lateral roots’ role”). This way, the taproot still contributes to anchorage against lateral stress. Indeed, the regions of the taproots close to the base of the tree are strengthened when horizontal forces push the tree, to lower the total energy expenditure for anchorage. Their bending resistance also allows them to reduce the forces exerted on both sides depending on the soil compressive resistance.
The Lateral Roots’ Role
In H. brasiliensis, the lateral roots grow as circular levels of roots from the primary taproot of a H. brasiliensis tree (Figure 8). They form multiple rings of roots, going outwards. These allow to, firstly, create a larger and stronger base of support, preventing the tree from toppling from its own height. By anchoring themselves into the soil with the aid of vertical sinker roots beyond even the reach of the branches in that circular pattern, lateral roots ensure that an area large enough around the tree works as the base of the tree (Priyadarshan, 2017). Additionally, lateral roots in H. brasiliensis are known to engage in intraspecific root grafting (Stachew et al., 2021), intermingling with other Hevea’s in the area’s roots to create a wide communal anchorage base. These two phenomena drastically improve the stability of the tree, making it difficult for the weight of its branches to act outside of the base, hence significantly reducing its chances of toppling.

Fig. 8. Examples of lateral root systems and their point of equilibrium, after three years’ growth in the field, from 6 clones of H. brasiliensis (Carron et al., 2000).
Secondly, by reaching this far from the tree both horizontally and vertically, lateral roots create a very large Root-Soil plate (Stachew et al., 2021), where the rooted soil behaves as a single unit when under load. This happens when resistance of the root-soil interface is higher than the surrounding soil strength. A strong and extensive Root-Soil plate can strengthen the soil’s shear strength by 1-17 kPa and stiffen it (similarly to steel bars in concrete) throughout the tree’s growth. Consequently, this not only allows for the base of the tree to be even heavier under its weight, but it also extends the area that is unlikely to deform under tensile and shear forces. This is the tree’s solution to weak or malleable soils: the Root-Soil Plate ensures that an area large enough for the tree to expand will not cede under lateral stress. Here is where H. brasiliensis differs from other trees: since its taproot is the origin of the rings of lateral roots, it goes deeper into the soil than them, reinforcing the Root-Soil plate and increasing the slip surface between the plate and the soil (Fourcaud et al., 2008).
The root system works as an ensemble to resist dynamic lateral loading conditions. In addition to the taproots’ work, lateral roots respond to the lateral stresses caused by gusts of wind with increased root growth and girth on the leeward side, where bending and compressive forces direct the roots towards the soil. On the leeward side, with the help of their branched vertical sinker roots, lateral roots resist the tensile and shear forces that drive the Root-Soil plate upwards. Its dynamic response to stress allows H. brasiliensis’ root system to efficiently allocate energy to stay upright among the trees of the canopy (Stachew et al., 2021).
Energy Distribution of Leaves
Texture and Structure of Leaves
The first notable structure of a typical Hevea brasiliensis tree is that it has a particularly long chunk of bare trunk, making up approximately 10 m of the trees, about a third of their total height. As shown in Figure 9, a large portion of the tree above ground is both branchless and leafless. This allows better light penetration at the bottom layers where there is more shade. Once it passes 10 meters in height, leaves emerge in groups of three around the node. During leaf formation, the apical meristem first develops the bud, a tough sheath that envelopes the immature leaves, protecting them during the maturation process, and finally unpeels when the leaf matures. Additionally, the growth of leaves follows a specific cluster pattern with the nodes producing triplets of leaves, these clusters of leaves are separated by the internodes, distributing the weight of the branch evenly. These large, oval shaped leaves, which are approximately 10-35 centimeters long and 5-15 centimeters wide at maturity, are seen in Figure 9. The leaves are attached to their branch by a leathery textured petiole, whose flexibility and durability helps the leaves withstand wind breakage and stay attached to the branches (Baidya et al., 2023). Overall, the long and slim leaves of H.brasiliensis, subjects them to more bending stress than shearing stress against wind, while the leathery textured petiole provides enough flexibility from fracturing and falling from the branch (Louf et al., 2018).

Fig. 9. Appearances of a full-grown H.brasiliensis, with specific leaf grown pattern in groups of three that together forms a dense cluster of leaves (Puccio & Beltramini, 2018; Baidya et al., 2023)
Light Interception
H.brasiliensis maximizes light interception through three features: the leaf orientation, leaf area per unit land area (LAI), and the crown architecture. Similar to the last section, the petiole has another role in leaf orientation. Specifically, it stabilizes the lamina’s attachment to the branch and orients it at an angle perpendicular to the stem, thus optimizing its photosynthetic abilities by maximizing its exposure to the sun (Louf et al., 2018). During hot summers with sufficient water supply, canopies are as dense as having a high LAI of 6-7. This leaf area index value indicates that for every 1 m2 of land, there is 6-7 m2 of area covered by leaves, achieved by stacking multiple thick layers of leaves throughout the upper and middle section of the tree. H.brasiliensis’ high density of leaves increases the area where incident photosynthetically active radiation (PAR) interacts with the photosystems of the leaves to perform photosynthesis (Devakumar et al., 1999; Kirkham, 2023).
In order to have a high leaf density, there is a notable difference among the top layer of leaves in irrigated trees. Specifically, these trees have a wider primary branch angle of around 58°, which provides room for secondary branches to grow and hold more leaves. In contrast, the crown architecture is much smaller among rainfed trees during hot season. These tree have a smaller branch angle of 49° , which has less room for secondary branches and leaves, causing their canopy to smaller and less compact. When there are not enough water resources, the energy of the tree is allocated towards survival, rather than growth, and the top outer layer is photoinhibited from saturated light. Meanwhile, the minimal water also limits their ability to perform photosynthesis, causing a the top layer to have less leaf and allows more light to penetrate to the middle and bottom layers, shifting the primary photosynthesis role to older leaves on lower layers to assimilate carbon. While the photosynthetic efficiency decreases when the lower layers are primarily photosynthesizing, it allows the top leaves to minimize their energy expenditure for survival. As seen in Fig. 10, there is a significant difference for photon flux density (PFD) between irrigated and rainfed trees during summer, when the irrigated trees still have dense leaf layers, while the rainfed trees become sparse; it converges again post monsoon rain, exhibiting identical crown architecture again. These changes in branch angle, leaf density, and crown shape of H.brasiliensis account for the amount of PFD interception in extreme weathers based on water availability (Devakumar et al., 1999).

Fig. 10. Illustration of different levels of photon flux density on upper and lower layer of leaves. Comparing irrigated and rainfed trees, 185 μmol/m²·s of PFD penetrates through all layer of the leaves and to the ground, the rainfed tree allowed 944 μmol/m²·s of PFD to penetrate to the ground, due to a less compact leaf (Devakumar et al., 1999).
Now, during monsoon seasons, where H.brasiliensi has high LAI, the incident photosynthetic photon flux density (PPFD) is always highest among the top layer of the canopy, followed by the lower layers. As shown in Figure 11, the PPFD is generally higher among top and middle layers than the bottom layer. To account for this different level of light interception, H.brasiliensis’ photosynthetic capacity is highest at the top layer, being the densest layer, and functioning at 40% more than the bottom leaves. Additionally, the top and bottom layer have a different saturation level of light intensity to perform photosynthesis, with the bottom layer only requiring 10% of the light intensity of the top layer, at 100 µE s-1m-2 to reach its photosynthetic threshold (Satheesan et al., 1984).

Fig. 11. Distribution of photosynthetic photon flux density absorbed by the top (⭘), middle(⏺) and bottom layers (x) on a clear day (top) and on a rainy day (bottom) (Gunasekera et al., 2013)
The lower leaves produce a sufficient amount of energy via photosynthesis by having higher quantum efficiency, as it has an increased amount of chlorophyll concentration per leaf that allows them to photosynthesize with this lower light intensity (Gunasekera et al., 2013).
Microclimate and Energy Dissipation
The relative humidity (RH) among the three canopy layers also varies throughout the day, with the maximum RH being first detected at the top layer in both early morning and later afternoon; then between 10 a.m. and 2 p.m., it is the bottom layer that is the most humid. Compared to the well winded top layer, and the more shaded bottom layer, the middle layer of the canopy experiences a steeper gradient of temperature and RH between the leaves and the air. As such, the highest transpiration rate is consistently detected at the middle layer of the canopy, which supports why the highest RH is never found at the middle layer (Gunasekera et al., 2013). This high transpiration rate of the middle layers helps the tree's leaves to remain within a temperature range. Like other species, H.brasiliensis’ photosynthetic ability is best preserved between 15-45 °C, and the rate of CO2 assimilation (direct measurement of rate of photosynthesis) is modelled by the following equation:

Where P(T) and P(Topt) measure carbon assimilation rate at leaf temperature and optimal leaf temperature. To look at this deeper, Figure 12 depicts the ratio of A/Aopt over different temperatures, where a higher photosynthetic ability is illustrated at values close to 1. From this, it can be observed that the optimal temperature for H.brasiliensis’ to photosynthesize is at 30 °C (Kibler et al., 2023).

Fig. 12. Ratio of net carbon assimilation rate/optimal carbon assimilation rate over different temperature ranges (Kibler et al., 2023).
To maintain photosynthetic function, the leaf temperature has to be around 15-45°C, or at the ideal temperature of 30°C that maximizes photosynthetic ability. In order to do so, it relies on all layer’s, particularly the middle layer’s evapotranspirative abilities to release heat energy. Out of the total energy on the leaves Qa, which is the net radiation subtracting the heat lost to the ground. The leaf temperature TL fluctuates based on the amount of energy dissipated at latent heat flux (λE), the energy used by transpiration, or by sensible heat flux (H), the energy transferred to surrounding air. In equation 6, the evaporative fraction (fE) shows the amount of energy in the leaf used by transpiration:

This is tied to the temperature of the leaf by equation 7:

Where Ta is air temperature, TL is the leaf temperature, rH is aerodynamic resistance to heat transfer, cρ is specific heat capacity of air, ρ is air density, and k is geometry coefficient (1 for one-sided leaf, 2 for two-sided).
With higher transpiration, the latent heat flux increases, and the evaporation fraction approaches one, this keeps TL of H. brasiliensis as close as possible to the ideal temperature (Kibler et al., 2023).
The Energy Efficient Solution From H. brasiliensis
Like other trees, H. brasiliensis’ canopy architecture means that the amount of light on each layer differs. Therefore, if the photosynthetic efficiency of each layer is the same and does not account for the different amount of light interception, excessive energy will be wasted on unused chlorophyll organelles in the lower layers. To address this, the top layers have more chlorophyll concentration in each of their cells compared to the lower layers (Gunasekera et al., 2013). This allows for a higher level of photosynthetic efficiency that utilizes the higher amount of photosynthetically active radiation the top layer can intercept due to its proximity to the sun. Meanwhile, a lower concentration in lower layers ensures no unnecessary energy is wasted. Additionally, the tree addresses issues like drought common in its habitat of Southeast Asia by having smaller branch angles, decreasing the number of secondary branches (Devakumar et al., 1999). As such, under extenuating circumstances like drought, the smaller tree trunks only have to support a smaller canopy, as well as maintaining basic level of photosynthesis with the minimal amount of leaves it has. Overall, H. brasiliensis’ design principle is highly focused on utilizing available resources like light and energy based on the condition of the tree or its proximity to the sun.
The Laticiferous System and Physiology of Latex Flow
Laticifers Cells Involved in Plant Defense
Laticifers are defined as cells or rows of cells synthesizing and accumulating latex that can be classified into two types based on their terminal walls: articulated and nonarticulated (Figure 13). Articulated laticifer consists of a row of cells, anastomosed or not, that is continuously formed in the shoot apex (Figure 13 A, B). During anastomosis, the dissolution of terminal walls, which occurs early in the organogenesis, can be partial or complete (Figure 13 C). In terms of length, articulated laticifers vary greatly, going from two to four cells ranging from 200 to 400µm, to systems of cells that are hundreds of meters long. Such dimensions are possible because all the laticifers of the plant anastomose to form a complex network of tubes through all the organs. As for the nonarticulated laticifers, they are single elongated cells, branched or unbranched, that grow intrusively between other cells via a process called tip growth (Figure 13 B). Tip growth requires a partial disassembly of the cell wall components and a disruption of cell wall connections with surrounding mesophyll cells. Non-articulated laticifers develop from embryonic precursor cells called laticifer initials. As the embryo matures, these cells elongate and undergo karyokinesis without forming cell plates. Reaching lengths of tens of centimeters, they are the largest cell type in plants (Castelblanque et al., 2016; Ramos et al., 2019).

Fig. 13. The two types of laticifers. (A) Partial (PCw) or complete (CCw) dissolution of the terminal walls of articulated anastomosed laticifers with branched and unbranched nonarticulated laticifers. (B) Shoot apex beside the large arrow. (C) In the shoot apex, articulated anastomosed laticifers and their terminal walls identified by the thin arrows (Ramos et al., 2019).
According to recent studies, latex abundance in laticifers may be induced by jasmonic acid, a hormone involved in plant defense signaling. This indicates that laticifers contribute to the defense strategy of plants (Ramos et al., 2019). Moreover, for the H. brasiliensis, depending on the defense gene, expression levels are five to twenty times higher in the laticifers than in the leaves (Figure 14) (Kush et al., 1990).

Fig. 14. Expression levels of plant defense genes in leaf (LF) and laticifer (LT) of H. brasiliensis. (A) Chitinase, 1.1 kb. (B) Pathogenesis-related (PR) protein, 1.0 kb. (C) Chalcone synthase, 1.2 kb. (D) Chalcone isomerase, 0.7 kb. (E) Phenylalanine ammonia-lyase, 1.5 kb. (F) Cinnamyl alcohol dehydrogenase, 1.7 kb. (G) 5-Enolpyruvylshikimate-3-phosphate synthase, 1.8 kb (Kush et al., 1990).
The growth and distribution of laticifers throughout the plant body ensures an efficient and precise delivery system of their contents to a site of injury. When released at the point of an herbivory attack, the stickiness of latex traps and immobilizes herbivorous insects. Furthermore, some latex chemicals, like inducible and constitutive Pathogenesis-related (PR) proteins, have toxic effects on various plant aggressors. However, it is important to note that infectious processes like those triggered by fungi, bacteria, or viruses may not be initiated via laticifers. In those cases, the progress of these infections will face the structural network of laticifers that surround the primary site of infection and will be confined in it (Konno, 2011; Ramos et al., 2019).
Bark Anatomy
Two distinct zones can be determined in the Hevea bark: the outer hard blast and the inner soft base (Figure 15 A). With mostly discontinuous and nonfunctional laticifers, the outer hard blast plays a role of protection. In the inner soft base, there are continuous and productive laticifers differentiated from the vascular cambium that are oriented 3-5° in a counterclockwise direction to the vertical (Prabhakaran Nair, 2010). Anastomosed laticifers, also known as latex vessels, follow an arrangement of concentric cylinders among the phloem tissue (Figure 15 A, B). The cylinders form latex vessel rings in the bark of the rubber tree. Within a ring, there is lateral anastomosis between adjacent latex vessels to make up the laticiferous system, a network of interconnected vessels. When the rubber tree is tapped, the network of interconnected vessels allows the release of latex from both the punctured laticifers and the connected laticifers near the tapping cut (Priyadarshan, 2017; Yeang, 2005).

Fig. 15. Anatomy of the Hevea bark. (A) Cross section of a virgin bark with cambium (C), conducting phloem (CP), outer hard bark (OHB), inner soft bark (ISB), latex vessels (L), secondary xylem (SX), and vascular ray (VR). (B) Cross section of a regenerated bark with cork (C), inner soft bark (ISB), latex vessel ring (LR), outer hard bark (OHB), phelloderm (PH), vascular ray (VR), clustered stone cells (STC), secondary phloem (SP), sclerenchyma ring (SR), secondary xylem (SX), wood vessel (WV) (Priyadarshan, 2017).
Rubber Tapping to Better Understand Latex Flow
Turgor pressure is defined as the force applied on the elastic plant cell walls by the contents of the cell. This pressure is attributable to osmotica, a process in which a negative osmotic potential is set in the cell to allow water to enter. It is important to note that, in the case of rubber trees, due to limitations of the known methods of measurements, the measured turgor pressures are derived from a group of latex vessels and the conducting phloem. Thus, phloem turgor pressure (PTP) or phloem hydrostatic pressure is more precise than laticifer turgor pressure when talking about latex flow (An et al., 2014). In the intact latex vessels, latex accumulates under pressure of the order of 10 atmospheres (Yeang, 2005). When tapped, the latex vessels are breached, reducing the turgor pressure of the laticiferous system near the cut to atmospheric pressure. Between the cut itself and the nearby laticiferous system, there will be a PTP difference of 0.7-1.4 MPa. The sudden release of turgor pressure leads to a laticifer wall contraction and latex exudation, where cut latex vessels can contract up to one fifth of their diameter (An et al., 2014; Priyadarshan, 2017). Immediately after tapping, the loss of PTP decreases rapidly the latex flow before it gets stopped completely by the plugging of latex vessel extremities after a few minutes or even hours (Yeang, 2005; Priyadarshan, 2017). Figure 16 demonstrates latex exuding from a tapped rubber tree.

Fig. 16. Latex harvested by rubber tapping (Rubber Tree Extraction).
Within laticifers, there are specific unit-membrane vacuole-based organelles that represent around 20% of the latex volume known as lutoids. Vessel plugging which leads to the cessation of latex flow is due to the damage of these organelles caused by changes in osmotic concentration and shear stress. Damaged lutoids release the intralutoid coagulant serum, B-serum, which contains latex de-stabilizing factors, and leads to the formation of plugs of microflocs of rubber particles and degraded lutoids at the cut ends of the latex vessel (Priyadarshan, 2017; Yeang, 2005).
As shown in Figure 17, the PTP varies throughout the day. The decrease of PTP can be explained by the fact that, when exposed to more sunlight, stomatal transpiration rate is more active. A higher PTP leads to an increased yield of latex, which means that latex flow diminishes in increased sunlight (Table 2). Therefore, during the hours of greater sun exposure, the latex leaked becomes more viscous, which impacts the behavior strategies of herbivores. The feeding strategies of cutting and trenching insects consist of reducing the latex volume by draining in the tissue surrounding the area of the leaf to be ingested. The increased stickiness of latex hence restrains smaller insects and hinders the performance of their mouth apparatuses (An et al., 2014; Ramos et al., 2019).

Fig. 17. Diurnal variation of PTP in the foliation season, in August. The experimental site was in Danzhou, Hainan, China. It is a region with an average annual temperature of 23.3 ◦C and annual precipitation of 1826 mm. The values are the means of four 11-year-old rubber trees (An et al., 2014).
Table 2: Changes in latex yields according to different times of tapping. The data is from nine three-year-old rubber trees separated in three groups (An et al., 2014).
| Time of tapping | Latex yield (g) |
|---|---|
| 0:00 a.m. | 139 ± 28 |
| 6:00 a.m. | 127 ± 21 |
| 12:30 p.m. | 94 ± 16 |
Vital Role of Laticiferous System
The mechanism behind the growth of the nonarticulated laticifers combined with the anastomosis of articulated laticifers allows the laticiferous system to spread out throughout H. brasiliensis. Knowing that latex contains chemicals toxic to various plant aggressors and that its characteristic viscosity traps insects, the laticiferous system, which leaks out latex by pressure difference, plays a vital role in the protection of H. brasiliensis by delivering rapidly, efficiently, precisely, and everywhere latex. In the case of an infection by fungi, bacteria, or viruses, latex is not exuding since no damage is done to the laticifer system. However, the laticifer system is still able to confine the invader to the primary site of infection, which limits the progress of the disease. Thus, the laticiferous system contributes to the defense strategy of H. brasiliensis by either efficiently delivering latex or by forming an ultrastructural barrier against microbe dissemination (An et al., 2014; Konno, 2011; Ramos et al., 2019).
Conclusion
Natural species utilizes its sophisticated mechanisms to best survive and reproduce, and H.brasiliensis is no exception. As a seed, the tree aims to find an optimal environment that ensures the tree’s survivability through high reproductivity. To do so, the shell is structured to hold numerous seeds, and shaped to crack simultaneously (Deagan, 2012). Therefore, a small amount of stored energy in its walls has to be converted to one burst of energy to crack the shell, converting the rest to kinetic energy to propel the seed to an optimal environment. In its adulthood, the tall-standing, 30-40 m tree has to withstand tremendous force to stand up straight. Instead of developing a complex root system, its rare lateral and tap root system interconnects into the Root-soil plate, delegating its weight to neighboring trees. The energy of H.brasiliensis is supplied by its large, compact canopies, which adapt to the level of light interception on each layer of its canopy to use energy efficiently. To do so, its photosynthetic capacity varies among each layer due to the different levels of chlorophyll concentration. Finally, H.brasiliensis’ defensive mechanism delivers latex to wounds, plugging the site of injury with herbivore attacks and contains site of infection with microbe dissemination. This mechanism only relies on the tree’s natural turgor pressure to push the latex to the designated site. In fact, most of these design solutions are passive responses that arise from physical structures. Altogether, it shows the evolutionary ways H.brasiliensis configures its structures to adapt flexibly and survive a diverse range of circumstances.
References
References
An, F., Lin, W., Cahill, D. M., Rooks, J. E., Kong, L. (2014). Variation of phloem turgor pressure in Hevea brasiliensis: An implication for latex yield and tapping system optimization. Industrial Crops and Products, 58, 182-187. https://doi.org/10.1016/j.indcrop.2014.04.016
Baidya, M., Maji, H. S., & Kumar, S. A. (2023). Hevea brasiliensis: A concise review. International Journal of Biology, Pharmacy and Allied Sciences, 12(5), 1891–1902. https://doi.org/10.31032/ijbpas/2023/12.5.7092
Bakewell-Stone, P. (2025, May 27). Hevea brasiliensis (rubber) | cabi compendium. CABI Digital Library. https://www.cabidigitallibrary.org/doi/abs/10.1079/cabicompendium.27999
Balasubramanian, H. (2023, April 3). Rubber Tree: Facts, benefits, how to grow, and maintain. Housing News. https://housing.com/news/rubber-tree-hevea-brasiliensis/
Carron, M.-P., Le Roux, Y., Tison, J., Dea, B., Caussanel, V., Clair, J., & Keli, J. (2000). Compared root system architectures in seedlings and in vitro plantlets of Hevea brasiliensis, in the initial years of growth in the field. Plant and Soil, 223(1), 75-88. http://www.jstor.org/stable/42950792
Castelblanque, L., Balaguer, B., Martí, C., Rodríguez, J. J., Orozco, M., Vera, P. (2016). Novel Insights into the Organization of Laticifer Cells: A Cell Comprising a Unified Whole System. Plant Physiology, 172(2), 1032-1044. https://doi.org/10.1104/pp.16.00954
Crook, M., & Ennos, A. (1998). The increase in anchorage with tree size of the tropical tap rooted tree Mallotus wrayi, King (Euphorbiaceae). Annals of Botany, 82(3), 291-296. http://www.jstor.org/stable/42765791
de Carvalho, J., Miranda, M., Kramer, Y., Reis, A., & Gonçalves, J. (2022, January). Morphophysiological features of seeds and seedling between wild and cultivated genotypes of Heave brasiliensis. Digital Library. https://www.cabidigitallibrary.org/doi/pdf/10.5555/20230356720
Deegan, R. D. (2012, April 3). Finessing the fracture energy barrier in ballistic seed dispersal. Proceedings of the National Academy of Sciences of the United States of America. https://pmc.ncbi.nlm.nih.gov/articles/PMC3325694/
Devakumar, A. S., Prakash, P. G., Sathik, M. B. M., & Jacob, J. (1999). Drought alters the canopy architecture and micro-climate of Hevea brasiliensis trees. Trees, 13(3), 161–167. https://doi.org/10.1007/pl00009747
Fang, Y., Xiao, X., Lin, J., Lin, Q., Wang, J., Liu, K., Li, Z., Xing, J., Liu, Z., & Wang, B. (2024). Pan-genome and phylogenomic analyses highlight Hevea species delineation and rubber trait evolution. Nature Communications, 15(1), 7232. https://www.nature.com/articles/s41467-024-51031-3
Ding, H., Xue, L., Liu, H., Li, L., Wang, H., & Zhai, M. (2022). Influence of root volume, plant spacing, and planting pattern of tap-like tree root system on slope protection effect. Forests, 13(11), 1925. https://www.mdpi.com/1999-4907/13/11/1925#
Fourcaud, T., Ji, J.-N., Zhang, Z.-Q., & Stokes, A. (2008). Understanding the impact of root morphology on overturning mechanisms: a modelling approach. Annals of Botany, 101(8), 1267-1280. https://doi.org/10.1093/aob/mcm245
Gunasekera, H. K. L. K., De Costa, W., & Nugawela, A. (2013). Canopy photosynthetic capacity and light response parameters of rubber Hevea brasiliensis with reference to exploitation. Current Agriculture Research Journal, 1(1), 01–12. https://doi.org/10.12944/carj.1.1.01
Hayashi, M., Feilich, K. L., & Ellerby, D. J. (2009, March 25). The mechanics of explosive seed dispersal in orange jewelweed (impatiens capensis). Journal of experimental botany, 60(7), 2045-2053. https://pmc.ncbi.nlm.nih.gov/articles/PMC2682495/
Hofhuis, H., Moulton, D., Lessinnes, T., Routier-Kierzkowska, A.-L., Bomphrey, R. J., Mosca, G., Reinhardt, H., Sarchet, P., Gan, X., Tsiantis, M., Ventikos, Y., Walker, S., Goriely, A., Smith, R., & Hay, A. (2016, June 30). Morphomechanical innovation drives explosive seed dispersal. Cell. https://pmc.ncbi.nlm.nih.gov/articles/PMC4930488/
Kibler, C. L., Trugman, A. T., Roberts, D. A., Still, C. J., Scott, R. L., Caylor, K. K., Stella, J. C., & Singer, M. B. (2023). Evapotranspiration regulates leaf temperature and respiration in dryland vegetation. Agricultural and Forest Meteorology, 339, 1–14. https://doi.org/10.1016/j.agrformet.2023.109560
Kirkham, M. B. (2023). In Principles of Soil and Plant Water Relations (3rd ed., Vol. 1, pp. 17–31). Essay, Elsevier.
Konno, K. (2011). Plant latex and other exudates as plant defense systems: Roles of various defense chemicals and proteins contained therein. Phytochemistry, 72(13), 1510-1530. https://doi.org/10.1016/j.phytochem.2011.02.016
Kush, A., Goyvaerts, E., Chye, M. L., Chua, N. H. (1990). Laticifer-specific gene expression in Hevea brasiliensis (rubber tree). Proceedings of the National Academy of Sciences of the United States of America, 87(5), 1787-1790. https://doi.org/10.1073/pnas.87.5.1787
Louf, J.-F., Nelson, L., Kang, H., Song, P. N., Zehnbauer, T., & Jung, S. (2018). How wind drives the correlation between leaf shape and mechanical properties. Scientific Reports, 8(1). https://doi.org/10.1038/s41598-018-34588-0
Prabhakaran Nair, K. P. (2010). 8 - Rubber (Hevea brasiliensis). The Agronomy and Economy of Important Tree Crops of the Developing World (pp.237-273). Elsevier. https://doi.org/10.1016/B978-0-12-384677-8.00008-4
Priyadarshan, P. M. (2017). Biology of Hevea Rubber. Springer Cham. https://doi.org/10.1007/978-3-319-54506-6
Puccio, P. (2018, February 2). Hevea brasiliensis. Monaco Nature Encyclopedia. https://www.monaconatureencyclopedia.com/hevea-brasiliensis/?lang=en
Ramos, M. V., Demarco, D., da Costa Souza, I. C., de Freitas, C. D. T. (2019). Laticifers, Latex, and Their Role in Plant Defense. Trends in Plant Science, 24(6), 553-567. https://doi.org/10.1016/j.tplants.2019.03.006 In-Text: (Ramos et al., 2019)
Rubber Tree Extraction [Photograph]. Good Nature Travel Blog. Retrieved September 21, 2025 from https://www.nathab.com/blog/rubber-tree-extraction
Satheesan, K. V., Rao, G. G., Sethuraj, M. R., & Raghavendra , A. S. (1984). Canopy Photosynthesis in Rubber (Hevea Brasiliensis): Characteristics of Leaves in Relation to Light Interception. In Advances in Photosynthesis Research (Vol. 4, pp. 125–128). essay, Springer Dordrecht.
Schultz, A.R., Parsons, J.J., Crist, R.E. (2025, September 16). Amazon River. Encyclopedia Britannica. https://www.britannica.com/place/Amazon-River
Stachew, E., Houette, T., & Gruber, P. (2021). Root systems research for bioinspired resilient design: A concept framework for foundation and coastal engineering. Frontiers in Robotics and AI, 8, 548444. https://doi.org/10.3389/frobt.2021.548444
Yeang, H. Y. (2005). The Kinetics of Latex Flow from the Rubber Tree in Relation to Latex Vessel Plugging and Turgor Pressure. Journal of Rubber Research, 8(3), 160-181. https://www.shoreaword.com/wp-content/uploads/2010/09/JNR-lx-flow-kinetics-Yeang-with-Corrigenda.pdf
Zhou, H., Yue, H., Ai, X., Chen, G., Cun, M., Xie, J., & Tian, Y. (2015, September 23). Poor seed dispersal, seed germination and seedling survival explain why rubber trees (Hevea brasiliensis) do not expand into natural forests in Xishuangbanna, Southwest China. ScienceDirect, 358, 240-247. https://www.sciencedirect.com/science/article/abs/pii/S0378112715004910