
Table of Contents
Keywords: Pistol Shrimp, Jet propulsion, Energy efficiency, Shockwaves, Antarctic Krill, Pressure Gradient, Cavitation, Hydrodynamic Signaling, Metachronal Stroking, Filtering system
Abstract
For centuries, organisms have developed complex and unique solutions to address environmental pressures and survival challenges. This paper explores how two ancient crustaceous superorganisms, the pistol shrimp and the Antarctic krill, adapted to and overcame specific pressures and challenges through ingenious physical mechanisms and strategies. The pistol shrimp’s snapping claw generates cavitation bubbles that stun or kill prey through rapid water jets, producing shockwaves, thermal spikes, and sonoluminescence. Antarctic krill, on the other hand, employ an efficient filter-feeding mechanism using thoracic legs to create a feeding basket, allowing them to filter food with precision. Additionally, krill swim in dense schools, optimizing energy use through jet propulsion and hydrodynamic signaling. The mechanisms and strategies discussed not only ensure the crustaceans’ survival but also offer insights into the evolutionary processes that drive biodiversity and resilience in marine ecosystems.
Introduction
Pistol shrimp and krill share a common ancestry as members of the subphylum Crustacea, which are characterized by their hard exoskeleton, segmented bodies, and jointed limbs. Crustaceans’ exoskeleton is composed of chitin and calcium carbonate, which provide protection and support, and is periodically molted to allow for growth. Their bodies are typically divided into three main regions: the cephalon (head), thorax, and abdomen. The order Euphausiacea, which includes krill, diverged from other crustaceans during the Lower Cretaceous period, around 130 million years ago. This divergence was driven by changes in the marine environment and the need to adapt to different ecological niches (Jarman, 2001). The main differentiator of pistol shrimp from other crustacea is the placement of the dactyl-closing muscle. Regular shrimp evolved to have a simple slip joint with all of the muscle below the fulcrum. However, they evolved a step further and have part of the muscle below the fulcrum and part of it above. This allows for a cocking slip joint, an energy storage system in their muscles that greatly increases the speed of the claw snap.

Fig. 1. Comparison of the simple slip joint and the cocking slip joint (Reproduced from Macdougal, 2021).
Pistol shrimps (Alpheidae) have asymmetrical front claws, with the larger one capable of producing a loud snapping sound. They are crevice-dwelling organisms that prefer tropical and temperate coastal waters, meaning they are mostly found in coral and oyster reefs, and sponge cavities (Bohnenstiehl et al., 2016). Pistol shrimp primarily prey on small invertebrates and fish. They use their powerful snapping claw to stun or kill their prey, but may also scavenge for detritus, algae, and carcasses near their burrows.
Antarctic krill (Euphausia superba) play a crucial role in the Southern Ocean's ecosystem and thrive in the Southern Ocean, particularly along the continental shelf and in deeper oceanic regions. Although individually small, their combined biomass is immense, making them one of the most abundant wild animal species on Earth, along with copepods, ants, and termites (Shao et al., 2023). Known as a keystone species, they are essential for maintaining the balance of the Antarctic food web. These tiny organisms serve as the primary food source for a wide variety of marine animals, from fish to large whales. Krill play a vital role in the Antarctic ecosystem by consuming phytoplankton and metabolizing it into a usable form by other animals, which then sustains higher-level predators. Shown in figure 2, krill contributes to the nutrient mixing and recycling within the ocean. Krill filter-feed on phytoplankton and zooplankton using specialized appendages known as endopodites and exopodites (Cavan et al., 2019).

Fig. 2. Cycling of nutrients by individual krill. Krill incorporates carbon, phosphorus, and calcium from phytoplankton and release essential nutrients such as ammonium (NH4) and organic compounds such as DOC, DON, DOP, which are crucial for maintaining the nutrient balance in the ecosystem. This process not only supports higher-level predators but also contributes to the nutrient mixing and recycling within the ocean. (Cavan et al., 2019)
The pistol shrimp and Antarctic krill are regarded as superorganisms because of their strong cooperative behaviors and the intricate social structures they develop within their groups. The former lives in mutualistic symbiotic relationships with organisms such as sponges and small fish, while the latter form large schools which require an immense amount of coordination to evade predators and enhance feeding efficiency.
How do pistol shrimp prey on fast-moving invertebrates? Why is filter feeding the optimal mechanism for Antarctic krill to feed on phytoplankton? What allows Antarctic krill to form and stay within densely packed schools? These are some of the questions that will be answered in the following paper. The mechanisms and strategies discussed not only ensure the crustaceans’ survival but also offer insights into the evolutionary processes that drive biodiversity and resilience in marine ecosystems.
The Pistol Shrimp’s Powerful Snap
The Mechanics of the Claw and the Snap
The mechanics of the pistol shrimp's snapping claw represents a convergence of biological design and physical principles. Characterized by their asymmetry, this shrimp has one distinctive disproportionately large claw, and another smaller one. The claw is a strikingly large appendage, often exceeding half the size of its body. The main segments are a protruding plunger on the hammer like structure called the dactylus, which is the moving part, and the pollex, which remains stationary. A unique feature of this claw is its angular offset between these two segments (Koukouvinis et al., 2017). This design prevents physical contact between the dactylus and pollex during the snapping action, differentiating it from the pincers of other crustaceans such as crabs and lobsters, which use their claws primarily for pinching prey or grasping objects (Fig. 3).

Fig. 3. Photographs of the snapper claw (Amini et al. 2018).
The snapping mechanism begins with the claw being cocked open through the co-contraction of opener and closer muscles, generating significant tension in the claw (Fig. 4). This preparatory phase is essential for the rapid closure that follows, which can occur in just 600 microseconds. When a second closer muscle contracts, it initiates an extremely fast closure of the claw. As the plunger on the dactylus is driven into the socket of the pollex, the resulting movement creates a high-velocity water jet and subsequent cavitation. The structure of the claw is intricately designed to facilitate this rapid closure. Specialized cocking pivot joints and slip joints evolve within the claw’s architecture, enhancing the efficiency of movement. Additionally, the surface of the dactylus features cone-shaped micro papillae, which serve to minimize underwater resistance during the snapping motion (Amini et al., 2018). This reduction in drag is crucial, as it allows for the rapid closure required to create the cavitation effects associated with the claw’s snap.

Fig. 4. Stages of the powerful snap. 1. The closed pistol shrimp claw with the hidden plunger (P). 2. Open claw with the exposed plunger (P) and chamber (C). 3. Open claw with water (W) entering the open chamber(C). 4. Claw with plunger (P) pushed into chamber (C), forcing jet stream (J) out of the chamber(C) (Ouellette, 2022).
Cavitation Bubble Formation
The pistol shrimp is renowned for its ability to generate cavitation through the rapid snap of its claw, producing high-velocity water jets that result in the formation of cavitation bubbles capable of stunning or killing prey. This process begins where the rapid claw closure generates a water jet with core velocities reaching up to 70 m/s. This results in a sharp drop in pressure, as described by Bernoulli’s principle, which defines the inverse relationship between the pressure and speed at a point in a fluid. The pressure falls below the vapor pressure of water, leading to the formation of cavitation bubbles from pre-existing microbubbles in the seawater. As the jet moves through the claw’s socket and nozzle, these microbubbles expand due to the low-pressure environment. At the same time, vortices form around the jet as its velocity decreases near the walls of the claw due to a pressure gradient. The pressure difference between the vortex core and its surrounding liquid is governed by Eq. 1.
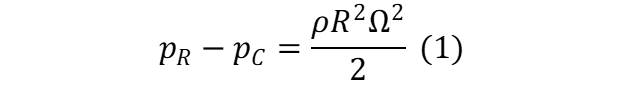
Where pR is the pressure at the vortex radius, pC is the pressure at the vortex core, ρ is the liquid density, R is the vortex radius, and Ω is the angular velocity of the vortex. In the case of the pistol shrimp, the pressure at the vortex core drops far below the vapor pressure of water, encouraging further cavitation. The boundary layer thickens and separates from the nozzle, leading to the formation of vortex structures near the nozzle with opposite rotational directions (Fig. 5). Again, the pressure at the core of these vortices drops significantly, creating ideal conditions for cavitation inception.

Fig. 5. Toroid bubble shape (Wikimedia Commons, n.d.).
As the water jet and vortices move forward, the cavitation bubbles that initially form near the nozzle develop and evolve. The vortices take on a ring-like structure (Yang et al., 2020), which guides the cavitation bubbles, expanding and transporting them along with the flow. The bubbles themselves change shape as they move with the jet, beginning as toroidal structures and gradually stretching into a more cone-like form as they are carried forward. This transformation, confirmed by both simulations and high-speed imaging, mirrors other high-speed jet phenomena, such as air vortex cannons, where vortex rings form and expand as the jet moves through fluid.
The development of vortex cavitation is driven by the interaction between the water jet and the surrounding fluid, which entrains additional fluid and causes the vortex ring and cavitation bubbles to grow. These expanding bubbles follow the movement of the vortex, which creates a persistent low-pressure zone that allows them to maintain their shape as they travel. The vortices not only play a critical role in initiating cavitation but also ensure that the bubbles remain intact and move with the jet until they are far enough from the shrimp’s claw.
Bubble Collapse and Energy Release
After the formation of the cavitation bubble, the most critical stage occurs: the bubble's collapse. It is during this collapse that the pistol shrimp's powerful snap reaches its full potential, unleashing stored energy explosively.
Once the cavitation bubble reaches its maximum size, it becomes unstable due to the higher pressure of the surrounding water. According to Pascal’s principle, any pressure change in a confined fluid is transmitted equally in all directions. This means that, as the external pressure overwhelms the vapor bubble, it is uniformly compressed from all sides. This compression is depicted in stage C of Figure 6. The re-pressurization forces the bubble to implode almost instantly as the surrounding water rushes in, as illustrated in stage D of Figure 6. This implosion is driven by the inertia of the water. Inertia, as explained by Newton’s First Law of Motion, is the tendency of an object to resist changes in its motion, and it is directly proportional to its mass: the greater the mass, the greater the inertia. Since liquid water has a much higher density than the gases inside the bubble (mainly water vapor), a given volume of water contains much more mass. This greater mass results in greater inertia, allowing the surrounding water to continue moving inward with significant force during the collapse. Additionally, water’s incompressibility ensures that the pressure from the surrounding liquid is transmitted efficiently and rapidly into the bubble, further accelerating the collapse by concentrating the energy inward. The pistol shrimp effectively leverages water’s intrinsic properties, density and incompressibility, to amplify the force of the bubble’s collapse.

Fig. 6. Stages of the cavitation bubble (ProSys, 2024).
This rapid inward compression resembles an adiabatic process, a type of process in which no heat is exchanged with the surroundings because it happens too quickly for heat transfer to occur. In this case, the collapse of the cavitation bubble occurs so rapidly that there is no time for heat to escape. As a result, as the bubble's volume decreases, all of the energy remains concentrated inside, setting the stage for the implosion.
When the bubble finally collapses, as shown in stage D of Figure 6, the stored energy is released explosively. This results in multiple distinct but interconnected effects: a shockwave, an intense acoustic impact, a thermal spike, and sonoluminescence. Each of these outcomes plays a critical role in the pistol shrimp's ability to hunt and defend itself in its underwater environment.
1. Shockwave
The first primary effect of the energy released during the collapse is the formation of a shockwave. A shockwave is a propagating disturbance that moves faster than the speed of sound, causing an abrupt increase in pressure, temperature, and density. The sudden im plosion of the cavitation bubble compresses the surrounding water, creating a high-pressure pulse that radiates outward as a shockwave. This process can be explained by Newton's third law of motion: as the water rushes inward to fill the collapsing bubble, it exerts an equal and opposite force outward, generating a shockwave.
Measurements show that cavitation bubble collapse from the pistol shrimp’s claw generates pressure pulses up to 80 bar (8 MPa) (Koukouvinis et al., 2017)—about the pressure found 800 meters underwater. Theoretical models estimate pressures as high as 2000 bar (200 MPa) (Koukouvinis et al., 2017), similar to the extreme pressures in deep-sea trenches.
This intense force is sufficient to stun or disorient prey, leaving them momentarily immobile and vulnerable to capture. By producing such a powerful shockwave, the pistol shrimp can incapacitate prey that would otherwise be too quick or resilient for direct confrontation (Williamson, 2024).
2. Acoustic impact
A second critical effect of the cavitation bubble's collapse is the intense acoustic impact generated during the process. As the bubble implodes, the rapid compression and subsequent movement of water generate a powerful sound that can reach levels of up to 200 decibels (dB) (Williamson, 2024). This makes the pistol shrimp’s snap one of the loudest biological sounds recorded in the ocean, comparable to the noise of a gunshot (Williamson, 2024). The sound is produced when the surrounding water rushes in to fill the void left by the collapsing bubble, creating a sharp pressure gradient that releases acoustic energy.
The loud snap is vital for the pistol shrimp's survival, primarily as a hunting mechanism. The intense sound, generated by the rapid closure of its claw, can disorient, stun, or even kill nearby prey, such as small fish and crustaceans (Williamson, 2024). This snapping action significantly increases the shrimp's chances of a successful capture.
Sound waves move efficiently through water due to its higher density compared to air. This density facilitates the effective transfer of sound vibrations between molecules, allowing acoustic signals to propagate farther with minimal energy loss.
Consequently, the pistol shrimp’s snap is used for communication and defense, often to attract mates and establish territorial boundaries (Williamson, 2024). Their burrows, which can reach up to three feet deep, are central to their habitat (Williamson, 2024). The powerful snap, which can be heard up to 3 kilometers away, is key to their ability to fend off competitors and predators without direct confrontation (Williamson, 2024).
3. Thermal spike and Sonoluminescence (“Shrimpoluminescence”)
As the cavitation bubble collapses, the rapid increase in pressure results in a significant rise in temperature, leading to what is known as a thermal spike (Lohse et al., 2001). As previously mentioned, this adiabatic process prevents heat from escaping, causing the internal energy to concentrate within the bubble (Lohse et al., 2001). Studies have recorded temperatures reaching 5000 K, comparable to the surface of the sun, during the collapse of the pistol shrimp's cavitation bubble (Lohse et al., 2001).
Alongside this extreme heat, a phenomenon known as sonoluminescence occurs. This process involves the compression of energy into a small volume as the bubble collapses, producing a brief flash of light (Lohse et al., 2001). Lohse et al. (2001) coined the term "shrimpoluminescence" to describe the first documented case of an animal generating light through the collapse of a cavitation bubble. The light emitted lasts only nanoseconds, coinciding with the moment when the bubble reaches its minimum volume (Lohse et al., 2001).
While shrimpoluminescence is a remarkable demonstration of the energy involved in cavitation, the biological significance remains uncertain. Most researchers consider both the light emission and the intense thermal spike a by-product of the energy released during the bubble's collapse, rather than evolved features with specific functions (Lohse et al., 2001). The light is not visible to the naked eye and does not occur at regular frequencies (Lohse et al., 2001), making it unlikely to serve as a communication tool or aid in prey detection. Similarly, the extreme temperatures generated inside the bubble are incidental to the process and do not serve a known biological role. Rather, the collapse-induced shockwave and acoustic impact serve as the primary mechanisms underlying the shrimp’s predatory and defensive behaviors. Ultimately, the pistol shrimp's snap is a remarkable demonstration of how a small organism can exploit fundamental physical principles—such as cavitation and shockwave generation—to thrive in its environment, harnessing with impressive efficiency for both predation and defense.
Thoracic Legs
Antarctic Krill’s Ingenious Water Filtering System
In the cold waters of the Antarctic, Antarctic Krill (Euphausia superba) have developed an efficient way of feeding that allows them to thrive in this challenging environment. These small crustaceans are filter feeders, meaning they rely on microorganisms like phytoplankton from water. However, their method is more advanced than passively drifting through the ocean. Krill use their thoracic legs to create a specialized “feeding basket” (Fig. 7), a unique structure that allows them to filter the water around them with precision.

Fig. 7. Configuration of krill legs during feeding. The krill's endopodites and exopodites during feeding. The endopodites are folded below the midventral groove and actively engage in trapping food particles, while the exopodites assist in propulsion and stabilization. The compression filtration mechanism is illustrated, where the legs open to draw in water and food particles and then close to expel water, trapping food on the filter setae (Hamner, 1988).
The configuration of the krill’s during feeding is essential. Its endopodites and exopodites work together to trap food particles from the water. Krill rhythmically open and close their legs to enclose water, which creates a "compression filtration" system. The endopodites are the inner branches of the krill’s leg and are directly involved in the filtration process by assisting in trapping food particles. On the other hand, the exopodites are the outer branches that aid in swimming and help stabilize the krill’s movement.
Together, these two parts of the legs coordinate to form a filtering net that captures small plankton and particles in the water as the krill moves. When the legs spread apart during feeding, a pressure gradient is created, pulling water and particles into the feeding basket from the front. The legs then rapidly come together to squeeze the water out, leaving the food particles trapped on the filter setae (fine hair-like structures) (Hamner,1988). It is an efficient, active way to collect nutrients in an environment where food can be scarce.
Pressure Gradient: the Secret to Success
Krill generate a pressure gradient during feeding by expanding their thoracic appendages outward (Figure 8). This gradient draws water and food particles into the feeding basket. Notably, water only enters from the front; the basket is designed to prevent water from entering through the sides, below, or behind (Hamner, 1988). This directional flow design minimizes wasted effort and maximizes feeding efficiency.

Fig. 8. Feeding mechanism of Antarctic krill using pressure gradient for efficient food capture. The three stages of how water and food particles are drawn into the feeding basket and expelled are shown: the feeding basket open (frame 449), partially closed (frame 455), and fully closed (frame 464), highlighting how the krill manipulates its appendages to capture food. (Hamner, 1988)
The filter itself is composed of a fine mesh formed by overlapping setae on the krill's legs (Fig. 9). Each of the six pairs of thoracic legs has long filter setae, with even smaller secondary and tertiary setules that create a fine mesh for trapping particles. As water passes through the filter, food particles are captured while the water is expelled.

Fig. 9. Scanning electron micrograph of filter setae. The filter is composed of primary setae (P), secondary setae (S), and tertiary setules (T), which together form a fine mesh used for trapping food particles from the water. This system plays a crucial role in the krill's feeding strategy, allowing it to efficiently filter and capture food while expelling water (Hamner, 1988).
Once the food is trapped in the filter, krill squeeze water out by closing their legs, forcing the water through the filter setae while retaining food particles inside. The exopodites, which are part of the leg structure, function like flapper valves. During the compression stroke, these valves lift slightly to allow water to escape but prevent water from entering during the next intake stroke (Hamner, 1988). This process is finely tuned to maximize the efficiency of food capture, as illustrated in the scanning electron micrograph in Figure 9, which shows the seta and setule that make up the filter system.
This finely tuned system shows how krill have adapted to efficiently gather the resources they need to survive in the vast Antarctic waters. Their feeding strategy is a remarkable example of how organisms can evolve specialized tools to make the most of their environment.
Krill Schools
As superorganisms, krill congregate in massive groups known as schools (Fig. 10). These groups are classified as schools rather than swarms or aggregations due to the polarized nature of the member krill (Tarling & Fielding, 2016). A typical school can range from tens to thousands of meters in length with an estimated density of 20,000 to 30,000 krill per cubic meter (Murphy et al., 2019). However, these schools are also largely variable, meaning they can either be large and scattered, or dense and exist in smaller patches (Miller et al., 2019).

Fig. 10. Photograph of an Antarctic krill school (Alberts, 2022).
Variations in the distribution of light and nutrients occur both temporally and spatially in the ocean. Phytoplankton, zooplankton, and other small invertebrates that rely on localized patches of light and nutrients for survival also tend to form aggregations. Krill's survival depends on encountering these dense aggregations of small invertebrates. However, groups can locate food patches faster than individuals and schooling behavior itself promotes long-distance horizontal or vertical search patterns (Hamner et al., 1983). It is comparable to a search party for a missing person; a group of people will cover more ground and find the missing person quicker than a single solo searcher will. Additionally, baleen whales, the primary predators of krill, can eat up to 16 tons of krill in one day. However, attacks on groups are often less successful, with capture rate decreasing as group size increases (Landeau and Terbogh, 1986). The amount of prey in the predator’s vicinity can overwhelm the predator, and though some of the krill may be eaten by the predator, their sacrifice will allow for most of the krill to scatter and escape. Thus, krill have developed and upheld the behavior of swimming in schools as it provides efficiency in foraging and protection from predators.
Jet Propulsion: Energy Saving Theory
In denser schools, krill swim in extreme proximity to one another, indicating how they favor swimming in the propulsion jet of the swimmer in front of them (Murphy et al., 2019). The principles of jet propulsion are based on Newton’s third law of motion, which states that for every action, there is an equal and opposite reaction (Benson, 2021). In this case, when thousands of krill push water back simultaneously, a cumulative force of these actions propels the entire group forward. This propulsion mechanism is also improved by how vortex rings form. After closing its abdomen and speeding up, Euphausia superba creates a clear chain of vortex rings behind its antennae (Fig. 11). As the krill swims forwards or backwards, it experiences fluid shear, which is the stress in a fluid caused by layers moving at different speeds. This occurs due to the no-slip condition at its surface, meaning that a fluid in contact with the krill will have the same velocity as the krill itself. At the tips of its antennae, this shear mixes with the suction flow produced by its movement, leading to the creation of these vortex rings (Connor & Webster, 2023).

Fig. 11. A diagram which shows the flow created by the krill, causing fluid to shear off and form vortex rings behind its antennae (Connor & Webster, 2023).
By swimming in this structured flow, krill not only capitalize on the momentum of the leading individual, thereby conserving energy to maintain speed, but the low-pressure vortex generated by the propulsion jet also reduces the drag experienced by the following krill. This reduction in drag arises from the difference in fluid velocity and the speed of the individual krill, which aligns with Bernoulli’s principle (Hall, 2022). Indeed, assuming horizontal fluid flow, faster-moving fluid areas will exhibit lower pressure compared to slower-moving areas (Hall, 2021). Thus, a lower pressure in the vortex would result in an increase in the fluid velocity moving in the same direction, causing less resistance against the moving organism. Nonetheless, there is a lack of experimental evidence on this energy-saving theory. In fact, some believe the reason krill place themselves within the propulsion jet of their leading neighbor is to have improved communication and coordination through hydrodynamic signals (Murphy et al., 2019).
Jet Propulsion: Hydrodynamic Signal Creation
Krill have eyes that help them evade predators and fishing nets, locate phytoplankton, and see other krill ahead, but vision alone cannot provide the continuous communication necessary to maintain the school. This is especially true at
night and in the deep parts of the ocean, where visibility is limited. Therefore, krill rely on hydrodynamic signals, or movements in the water around them, to perceive their position relative to their neighbors (Fig. 12). Thus, the krill’s ability to create and receive these hydrodynamic signals is critical for the formation and preservation of a school. As krill propel themselves through the water, they produce a high-velocity jet-like flow that causes disturbances in the water below and behind them. The neighboring krill sense these disturbances and are then able to monitor their position and coordinate their movements with the school. So, to understand the creation of hydrodynamic signals, the mechanics of krill motion must be discussed.

Fig. 12. The velocity vector fields for synchronous paddling, with red indicating counterclockwise and blue indicating clockwise vorticity. The red boxes highlight the vortices (Ford, 2019).
Actuator Disk Theory
Krill, a negatively buoyant animal, must, in addition to propelling themselves through the water, keep itself from sinking. To accomplish this, krill beat their five pairs of pleopods, which are paddle-shaped appendages, in rhythmic oscillations. Each pair experiences a phase delay relative to their adjacent pairs, creating a metachronal wave, which is a wavy coordinated movement produced by sequential action in the direction the krill is moving (Ford et al., 2019). The pleopods function like paddles as they drag through the water, creating vortices with every beat (Fig. 12). The amalgamation of these vortices provides the thrust required to sustain movement in both the forward and upward directions. The greater the delay between individual pleopod beats, the greater the angular orientation of the vertical thrust generated (Ford et al., 2019).
The force required for krill to remain in the same spot of the vertical column can be calculated through the actuator disk theory. The actuator disk theory is a mathematical model used to describe the performance of propellers and rotos in fluid dynamics. When applied to krill swimming through water with metachronal strokes, the theory helps to understand how the coordinated wave-like movements of their appendages generate thrust and propel the krill forward. Each of a krill’s five pleopods can be modelled as a single actuator disk (Fig. 13). To understand this theory, it is necessary to be familiar with Bernoulli's Principle, which was previously stated. Thus, Equation 2 can be derived through Bernoulli’s equation with the following pressures and velocities corresponding to the different points around the pleopods.

Fig. 13. Illustration of the conceptual framework for actuator disk theory. It can be pictured as a model for one of the krill’s pleopods (Murphy et al., 2013).

The difference in pressure across the area of the pleopods creates a force (𝐹=𝐴⋅∆𝑃 ), which in turn counteracts the underwater weight (𝑊𝑢) of the krill, allowing it to hover. Thus, the upthrust force the animal experiences is equal to its underwater weight.

𝑇 represents the thrust produced by the krill or the force needed to hover; Wu denotes the underwater weight, which is equivalent to the thrust in this context; 𝜌 is the density of the fluid (usually water) in which the krill is swimming; 𝐴 is the area of the actuator disk, which can be thought of as the effective area of the pleopod; vW is the wake velocity, which is the speed of the fluid moving in the wake created by the krill as it generates thrust. Thus, the equation expresses how thrust is related to the fluid's properties and the krill's movement, illustrating the relationship between these factors in generating upward force.
The principle of the actuator disk illustrates how there is enough momentum generated by pressure gradients to support the weight of the krill underwater. Power can then be calculated by manipulating the formula with the mass flow rate as well as kinetic energy (Eq. 4).

Plugging in the different values for these variables, the resulting power consumption of one 43-mm krill is roughly 4.2 x 10⁻⁶ J, which for one day is equivalent to 0.363 J. According to (Clarke & Morris, 1983) and (Cataldo-Mendez et al., 2024) respectively, krill consume 5% of its body weight per day and during the summer season has an energy content of 15.24 and 22.6 kJ/g of dry mass. Assuming the weight of one 43-mm individual to be around 0.25 g (Constable & Kawaguchi, 2018), the daily energy consumption would range between 190.5 J and 282.5 J. As a result, the average percentage of energy allocated to hovering would be just 0.16%. This illustrates how little energy krill use for hovering, indicating that they devote most of their energy to other critical functions such as paddling, which has been identified as an ineffective swimming technique for individual krill (Murphy et al., 2013). While paddling may seem inefficient for a single krill, it plays a crucial role in the context of a school. The collective movement of many krill, each contributing to the propulsion through their rhythmic beating of pleopods, generates a powerful jet that enhances the overall efficiency of the group. This method of swimming, although not energy-efficient for an individual, provides safety in numbers and improves the school's ability to evade predators.
Hence, in a school, the shared dynamics of paddling create a cohesive flow that allows krill to conserve energy while maximizing their collective thrust. This design solution highlights the importance of social behavior and cooperative movement, enabling krill to navigate their environment effectively. By prioritizing safety and coordination over individual efficiency, krill can enhance their survival while maintaining the energy budget necessary for reproduction and other vital activities. Thus, while paddling may appear ineffective for a single krill, it becomes a strategic advantage in the context of a school, ensuring both safety and efficiency.
Conclusion
Nature’s design solutions are exhibited by the pistol shrimp and Antarctic krill, where they adapt to overcome their environmental challenges with efficiency. Both pistol shrimp and Antarctic krill are captivating examples of how superorganisms in nature evolve ingenious mechanisms and intricate cooperative behaviors to enhance survival and reproductive success.
For example, the pistol shrimp has developed a unique solution to hunting and communication by collapsing cavitation bubbles with explosive force. This adaptation produces shockwaves and intense thermal spikes, enabling the shrimp to stun its prey and communicate in its surroundings. This design demonstrates how the shrimp harnesses physical phenomena, turning natural forces into tools for survival.
Similar to the pistol shrimp, the Antarctic krill faces a critical challenge and has evolved specialized energy-efficient movement and avoidance of their predators such as whales, fish, and squid. To thrive in their environment, they must optimize their energy use and communicate effectively. One of their key design solutions involves the coordinated movement of their pleopods, enabling jet propulsion for quick escapes while conserving energy. Additionally, swimming in schools enhances their hydrodynamic signaling, allowing them to communicate and confuse predators more effectively. Together, these adaptations help krill maximize their energy efficiency and increase their chances of survival in their dynamic ecosystem.
The pistol shrimp and Antarctic krill provide compelling examples of nature's ability to solve environmental challenges through evolutionary innovation. Both organisms showcase how natural forces and behaviors are harnessed and refined, allowing even the smallest creatures to thrive in their respective ecosystems.
References
References
Alberts, E. C. (2022, October 2). Krill, the most abundant species on earth and key food source for whales, are in trouble. Deep Green Resistance News Service. https://dgrnewsservice.org/civilization/even-antarctic-krill-the-most-abundant-species-on-earth-are-threatened/
Amini, S., Tadayon, M., Chua, J. Q. I., & Miserez, A. (2018). Multi-scale structural design and biomechanics of the pistol shrimp Snapper Claw. Acta Biomaterialia, 73, 449–457. https://doi.org/10.1016/j.actbio.2018.04.038
Benson, T. (2021, May 5). Newton's Third Law Applied to Aerodynamics. NASA Glenn Research Center. Retrieved 30 September 2024 from https://www.grc.nasa.gov/www/BGH/newton3.html
Bohnenstiehl, D. R., Lillis, A., & Eggleston, D. B. (2016). The Curious Acoustic Behavior of Estuarine Snapping Shrimp: Temporal Patterns of Snapping Shrimp Sound in Sub-Tidal Oyster Reef Habitat. PLOS ONE, 11(1), e0143691. https://doi.org/10.1371/journal.pone.0143691
Cataldo-Mendez, C., Kawaguchi, S., Cox, M. J., Melvin, J., Rae, V., & Swadling, K. M. (2024). The energy content and demographic composition of Antarctic krill (Euphausia superba) swarms in East Antarctica. Frontiers in Marine Science, 11. https://doi.org/10.3389/fmars.2024.1337080
Category: Tesseract torus rgby. Wikimedia Commons. (n.d.). https://commons.wikimedia.org/wiki/Category:Tesseract_torus_rgby
Cavan, E. L., Belcher, A., Atkinson, A., Hill, S. L., Kawaguchi, S., McCormack, S., Meyer, B., Nicol, S., Ratnarajah, L., Schmidt, K., Steinberg, D. K., Tarling, G. A., & Boyd, P. W. (2019). The importance of Antarctic krill in biogeochemical cycles. Nature Communications, 10(1). https://doi.org/10.1038/s41467-019-12668-7
Cavitation. ProSys. (2024, January 15). https://prosysmeg.com/cavitation/
Clarke, A., & Morris, D. J. (1983). Towards an energy budget for krill: The physiology and biochemistry of Euphausia superba Dana. Polar Biology, 2(2), 69-86. https://doi.org/10.1007/bf00303172
Connor, A. A., & Webster, D. R. (2023). Hydrodynamics of the fast-start caridoid escape response in Antarctic krill, Euphausia superba. Scientific Reports, 13(1). https://doi.org/10.1038/s41598-023-31676-8
Constable, A. J., & Kawaguchi, S. (2018). Modelling growth and reproduction of Antarctic krill, Euphausia superba, based on temperature, food and resource allocation amongst life history functions. ICES Journal of Marine Science, 75(2), 738-750. https://doi.org/10.1093/icesjms/fsx190
Ford, M. P., Lai, H. K., Samaee, M., & Santhanakrishnan, A. (2019). Hydrodynamics of metachronal paddling: effects of varying Reynolds number and phase lag. Royal Society Open Science, 6(10), 191387. https://doi.org/10.1098/rsos.191387
Hall, N. (2021, May 13). Bernoulli's Equation. NASA Glenn Research Center. Retrieved 30 September 2024 from https://www.grc.nasa.gov/WWW/K-12/airplane/bern.html
Hall, N. (2022). What is Drag? https://www1.grc.nasa.gov/beginners-guide-to-aeronautics/what-is-drag/#drag
Hamner, W. M., Hamner, P. P., Strand, S. W., & Gilmer, R. W. (1983). Behavior of Antarctic Krill, Euphausia superba: Chemoreception, Feeding, Schooling, and Molting. Science, 220(4595), 433–435. https://doi.org/10.1126/science.220.4595.433
Jarman, S. (2001). The evolutionary history of krill inferred from nuclear large subunit rDNA sequence analysis. Biological Journal of the Linnean Society, 73(2), 199-212. https://doi.org/10.1006/bijl.2001.0538
Koukouvinis, P., Bruecker, C., & Gavaises, M. (2017). Unveiling the physical mechanism behind pistol shrimp cavitation. Scientific Reports, 7(1), 13994. https://doi.org/10.1038/s41598-017-14312-0
Landeau, L., & Terborgh, J. (1986). Oddity and the ‘confusion effect’ in predation. Animal Behaviour, 34(5), 1372–1380. https://doi.org/10.1016/s0003-3472(86)80208-1
Lohse, D., Schmitz, B., & Versluis, M. (2001). Snapping shrimp make flashing bubbles. Nature, 413(6855), 477-478. https://doi.org/10.1038/35097152
Macdougal, H. (2021, August 31). How did snapping shrimp evolve their snap?. Science Connected Magazine. https://magazine.scienceconnected.org/2021/08/snapping-shrimp-evolved-snap/
Miller, E. J., Potts, J. M., Cox, M. J., Miller, B. S., Calderan, S., Leaper, R., Olson, P. A., O’Driscoll, R. L., & Double, M. C. (2019). The characteristics of krill swarms in relation to aggregating Antarctic Blue Whales. Scientific Reports, 9(1). https://doi.org/10.1038/s41598-019-52792-4
Murphy, D. W., Olsen, D., Kanagawa, M., King, R., Kawaguchi, S., Osborn, J., Webster, D. R., & Yen, J. (2019). The Three Dimensional Spatial Structure of Antarctic Krill Schools in the Laboratory. Scientific Reports, 9(1). https://doi.org/10.1038/s41598-018-37379-9
Murphy, D. W., Webster, D. R., & Yen, J. (2013). The hydrodynamics of hovering in Antarctic krill. Limnology and Oceanography: Fluids and Environments, 3(1), 240-255. https://doi.org/10.1215/21573689-2401713
Ouellette, J. (2022, July 12). This is why the pistol shrimp is immune to its own powerful shock waves. Ars Technica. https://arstechnica.com/science/2022/07/pistol-shrimp-sport-tiny-helmets-to-protect-selves-from-their-own-shock-waves/
ProSys. (2024). Cavitation. Retrieved October 11, 2024, from https://prosysmeg.com/cavitation/
Shao, S., Sun, K., Liu, J., Wang, J., Li, S., Liu, Q., Deagle, B. E., Seim, I., Biscontin, A., Wang, Q., Liu, X., Kawaguchi, S., Liu, Y., Jarman, S., Wang, Y., Wang, H.-Y., Huang, G., Hu, J., Feng, B., De Pittà, C., Liu, S., Wang, R., Ma, K., Ying, Y., Sales, G., Sun, T., Wang, X., Zhang, Y., Zhao, Y., Pan, S., Hao, X., Wang, Y., Xu, J., Yue, B., Sun, Y., Zhang, H., Xu, M., Liu, Y., Jia, X., Zhu, J., Liu, S., Ruan, J., Zhang, G., Yang, H., Xu, X., Wang, J., Zhao, X., Meyer, B., & Fan, G. (2023). The enormous repetitive Antarctic krill genome reveals environmental adaptations and population insights. Cell, 186(6), 1279-1294.e19. https://doi.org/10.1016/j.cell.2023.02.005
Tarling, G.A. & Fielding, S. (2016). Swarming and Behaviour in Antarctic Krill. In: Siegel, V. (eds) Biology and Ecology of Antarctic Krill. Advances in Polar Ecology. Springer, Cham. https://doi.org/10.1007/978-3-319-29279-3_8
Versluis, M., Schmitz, B., von der Heydt, A., & Lohse, D. (2000). How Snapping Shrimp Snap: Through Cavitating Bubbles. Science, 289(5487), 2114-2117. https://doi.org/doi:10.1126/science.289.5487.2114
Williamson, J. (2024). Pistol Shrimps: The Super Snappers of the Sea. AnimalResearcher. Retrieved October 11, 2024 from https://animalresearcher.com/pistol-shrimps-the-super-snappers-of-the-sea/
Yang, Y., Qin, S., Di, C., Qin, J., Wu, D., & Zhao, J. (2020). Research on Claw Motion Characteristics and Cavitation Bubbles of Snapping Shrimp. Applied bionics and biomechanics, 2020, 6585729. https://doi.org/10.1155/2020/6585729