Table of Contents
Keywords: sequoia, mathematics, fractal dimension, growth rate, fire, Fibonacci, clustering, tension fork, networks, graph theory
Abstract
The sequoia tree has evolved to solve a variety of problems throughout its life, from surviving droughts to resisting mechanical stress. As such, the tree exhibits patterns on different scales. This essay presents how sequoias use mathematics to survive and thrive within their environment. To avoid dehydration during droughts, the sequoia exhibits lower fractality, reducing transpiration by lowering their total leaf surface area. However, the lower surface area also ends up reducing growth rate. Another factor limiting the sequoia’s growth rate is competition. Denser stands reduce the speed at which a tree can grow, though sequoia trees are able to minimize this effect with the help of thinning events such as forest fires. The lower leaf surface area can also be countered via the use of the Fibonacci pattern. This pattern is used by sequoia trees to make stronger cones, but the spacing created by the pattern minimizes leaf overlap, which increases light capturing efficiency. In addition, sequoia trees tend to clump in mosaic aggregation, which favors group diversity within the species. On top of that, when the stem of sequoias separates into smaller branches, creating the shape of a two-pronged fork, the shape and structure of the fork distribute mechanical stress along the inner contour, which reduces the risk of breakage. This resistance to stress is further enhanced by the structure of tree’s wood, made of lignin and polymers. On a relatively small scale, these lignin and polymers are organized into a hierarchical network, which is resistant to random failures. However, on a larger scale, many hierarchical networks combine into a scale-free network. Thus, the sequoia benefits from the resilience of both hierarchical and scale-free networks.
Introduction
Sequoiadendron giganteum and Sequoia sempervirens are the two marvelous species of sequoia that span across the state of California, where they impress many with their remarkable height and size. Despite their shared ancestry, both species live in vastly different habitats. The coast redwoods live, as their name suggests, along the Californian coastline, where the climate is cold and foggy. Meanwhile, the giant sequoias are situated in the middle of California and must deal with dry air and many raging storms across their lifespans of thousands of years (Burns et al., 2018).
The sequoia’s structure has evolved to survive its rough living conditions by interacting with its environment using many principles of physics (see Sequoia Physics). Internally, the sequoia has been evolving chemical solutions to thrive as well (see Sequoia Chemistry). Now, it is time to talk about the big tree’s use of mathematical principles. Although it is not obvious, this tree uses math every moment it is alive, and even before that, when it is still one of the many seeds packed into its cone! This paper will talk about the math responsible for the sequoia’s branching pattern, drought resistance, competition, growth rate, and cone structure.
Tree Fractality and Drought Resistance
Sequoias, ostensibly, are remarkably featureless trees whose shape can be likened to tall cones. This is because the sequoias’ structure has a remarkably low fractal dimension. Where many trees exhibit intricate branching patterns that increase crown area, others present very streamlined, low fractality, highly vertical postures. Fig. 1 below illustrates what is represented as the fractal dimension of tree branching. Fig. 2 shows a glanceable outline of a typical sequoia’s structure.

Fig. 1. An illustration of the fractal dimension of simulated trees. (Created by Martel, A. A., 2025)

Fig. 2. A bottom-up view of a sequoia tree. Note the characteristically low fractality of its branching behavior (Olarte, 2018).
As discussed in the first paper of this series (see Sequoia Physics), sequoias present innovative solutions to resist the frequent occurrence of drought periods in their habitat, the Sierra Nevada in California. It is also possible to examine its water-stress resilience through the lens of the fractality of its structure. It has been found that trees exhibiting lower fractality in branching behavior also show very high resistance to water stress. This negative correlation between increasing fractality and specie drought resistance is especially strong for conifers like the sequoia: broad-leafed trees had , while needled trees had (Arseniou & MacFarlane, 2021). Less fractal tree crowns have reduced total leaf count and total leaf area, features that lead to lower heat gain and help reduce excessive water loss via leaf-level gas exchanges. As reported by Arseniou & MacFarlane (2021) urban trees can cope with the photosynthetically unfavorable consequences of lower leaf area because they are less likely to lie in the shade of other trees than trees in dense-canopy forests and because drought events occur frequently in urbanized areas. Sequoias, as the tallest trees in any forest, also share this advantage and drought risk, enabling them to minimize their crown area while ensuring sufficient photosynthesis for it to thrive. While sequoia saplings are more likely to experience shade from other trees due to their lesser size, the adult’s serotinous cones ensure that the forest canopy will not cast shade on the sapling, as discussed in the Sequoia Physics.
The Cupressaceae clade, which contains Sequoia sempervirens and Sequoia giganteum, has been theorized to have evolved its low-fractality crown during a major climate-change events of the Cenozoic during which the global atmospheric CO2 concentration decreased heavily, inducing a mean global temperature drop of 3-4ºCover approximately 300,000 years. This environmental change favored the evolution of closer-together, less fractal leaf arrangements due to the reduction of carbon dioxide in the atmosphere that limits the rate of photosynthesis over wider crowns (Pittermann, et al., 2012). This is done at the expense of growth rate (Arseniou, & MacFarlane, 2021), but sequoias notably engage in symbiotic relationships to help with sugars production (see Sequoia Chemistry).
Sequoia Growth Rate
Effects of Competition on Sequoia Growth
Although sequoia trees have the capacity to grow to large sizes, reaching these sizes takes time, and their growth can be impeded. One of the ways a sequoia’s growth rate can be impeded is competition with its own kind (Lalemand, et al., 2024). Lalemand, and colleagues (2024) found that thinning, the removal of certain trees from the population, generally increased the basal area increment (BAI) of sequoia sempervirens by 49%. BAI refers to the cross-sectional area that is added to a tree during its growing season (Lalemand, et al., 2024).
Determining the Growth Rate of the Sequoia Tree
Although the growth rate of trees can be determined via BAI, other measurements such as the quadratic mean diameter (Dq) are also helpful. The quadratic mean diameter (Dq), as shown in Eq. 1, can be thought of as the average trunk diameter at breast height of a population of trees (Curtis & Marshall, 2000). di is the diameter of the tree’s trunk at breast height, 1.4 m above the ground, of each individual tree, and n is the number of trees (Curtis & Marshall, 2000; Queensland Arboricultural Association, n.d.).

For sequoia sempervirens, the Dq function is very similar to the already existing Dq equation of the pine tree (Kimberley & Watt, 2021). As such, Kimberley and Watt (2021) found that the growth of Dq for sequoia trees can be represented as Eq. 2, where N is the number of trees per hectare of land, d controls how much stand density affects the growth rate, g is the Dq at which the Dq of a new stand surpasses the Dq of an older and denser stand, f controls how quickly trees notice a lack of competition before increasing their growth rate, and D(tBH) is another function that predicts Dq as a function of time tBH without considering competition (Kimberley & Watt, 2021).

In addition, thinning events can also be considered with the help of Eq. 3, where D1 and N1 are Dq and tree density respectively, before the thinning event, and D2 and N2 are Dq and tree density respectively, after the thinning event (Kimberley & Watt, 2021). As such, the quadratic mean diameter of a stand of sequoias after thinning can be determined.

Combining the effects of Eq. 2 and Eq. 3 gives Fig. 3 as shown below.

Fig. 3. Visualization of the of a stand of Dq Sequoia sempervirens. Lines A and B represent the Dq of a stand with a density of 300 trees/ha and 800 trees/ha respectively. Line C shows the Dq of a stand before and after thinning, with a tree density going from 800 trees/ha to 300 trees/ha. The sudden jump on line C is the thinning event. As weaker individuals, trees with smaller trunk diameters, are removed, the mean jumps up due to an increased proportion of trees with relatively bigger trunk diameters. Line C also increases faster after the thinning due to reduced competition. Δtthin helps determine the age of the thinned stand if it grew with a density of 300 trees/ha from the start. Δtthin + 0.25 is similar to Δtthin, but it also accounts for crown expansion after thinning (Kimberley & Watt, 2021).
Thus, as demonstrated in Fig. 3, the removal of competing individuals from the same species could contribute to the gigantic sizes certain sequoia trees can reach, since growth rate increases drastically after thinning.
Forest Fires and Sequoia Growth Rate
Thinning often refers to humans removing trees from a population to promote the health of the forest (Rayonier, 2024). However, natural thinning can occur in the form of forest fires. Due to the sequoia’s bark being physically and chemically resistant to fires (see Sequoia Physics and Sequoia Chemistry), it is possible that they benefit from forest fires more than other species. Their natural resistance to fires ensures that only adequately dominant trees get to survive. In contrast, younger or weaker individuals, sequoias with smaller trunk diameters, have lower chances of survival (Kane & Carrasco, 2025). However, if an individual survives, the lower competition from other sequoias ensures a boost to the tree’s growth rate, as they can acquire more sunlight, water, and nutrients for themselves. As such, in younger sequoias, living through a fire could increase its future chances of survival, since it can reach larger sizes faster, protecting it from future fires or other threats like boulders or herbivores. Meanwhile, older sequoias receive space to grow even larger. In addition, the removal of other species of trees that are not as well-adapted to forest fires, hence experiencing a higher mortality rate during forest fires, liberates even more space and nutrients for Sequoia sempervirens.
Fibonacci Sequence
Fibonacci Sequence in the Sequoia
Although it is subtle, the Fibonacci sequence can be found throughout nature: from the number of petals in sunflowers to the spiral of snail shells (Campbell, 2013; Minarova, 2014). Taking a closer look at the sequoia would reveal that it also uses this special mathematical pattern. This big tree makes use of the Fibonacci sequence twice: in both its cones and its branching. Each use of this pattern is an important design solution that the tree has adapted to thrive and will be discussed further in the subsections below. Before that, it is important to understand what the Fibonacci sequence is.
The Fibonacci sequence is a pattern of numbers, starting at 0, and increasing with each new number equal to the sum of the two numbers that precede it (Campbell, 2013). To better visualize it, the pattern can be observed by the simple equations (Eq. 4) below:

As seen above, the first few numbers of this sequence would be: 0, 1, 1, 2, 3, 5, 8, 13, etc. The nth Fibonacci number, represented by Fn, can be found using Eq. 5.
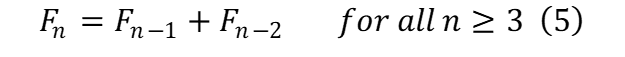
The Fibonacci pattern is usually represented as a unique spiral (Fig. 4), drawn using the help of squares of increasing size, that have the dimensions of the Fibonacci numbers (Minarova, 2014).

Fig. 4. The Fibonacci spiral (AwkwardBotany, 2019).
What makes the Fibonacci sequence unique is that it can be used to obtain an approximation of a number called the Golden Ratio (≈1.61803). This is achieved by taking any two neighboring numbers from the Fibonacci sequence and dividing the bigger by the smaller (Edkins, 2007).
Fibonacci in the Sequoia’s Cone
A closer look at the big tree’s cones would reveal that both the giant sequoia and the coast redwood’s cones have scales which, when observed from the top of the cone, form spirals that wrap around the cone in alternating opposite directions (Fig. 5). These spirals make up numbers in the Fibonacci fraction. In the case of the giant sequoia, these spirals are much easier to spot and make up a Fibonacci fraction of 3/5. This is because three of the spirals wrap around the cone to the left while the other five spirals wrap around to the right when counting from the cone’s stem. In a study observing thousands of sequoia cones, all but one cone displayed this 3:5 ratio. The singular outlying cone had another Fibonacci ratio: 5:8 (Campbell, 2013; Hartesveldt et al., 1975).

Fig. 5. Illustration of the sequoia cone and its 3:5 Fibonacci ratio. To the left is the view of the cone from the stem and to the right is the view from the side. Drawing by Ivan Linderman (Hartesveldt et al., 1975).
So far, there seems to be two reasons behind why these cones follow the Fibonacci sequence so strictly. For one, this sequence leads to an approximation of the Golden Ratio, which, when followed, should prevent the bracts of the cone from lining up. If they did, the cone’s structure would be weakened and much more susceptible to breaking (Minarova, 2014). The second reason is because the Golden Ratio also maximizes the spacing of parts, allowing for seeds to be as efficiently packed into the cone as possible (Vasiltsov, 2022).
Fibonacci in the Sequoia’s Branching Pattern
Interestingly, the sequoia’s branching pattern follows the same Fibonacci fraction as its cone: 3/5. To help visualize what this looks like, this means that the giant sequoia grows its branches in a spiral pattern, with each branch growing 3/5 of a revolution around the trunk or limb that it is growing from. Two branches will only be able to line up exactly one on top of the other after five branches, and three rotations around the trunk or limb (Campbell, 2013).
The reasoning behind the Fibonacci sequence being the sequoia’s design solution is once again due to its approximation to the Golden Ratio. In this case, the Golden Ratio helps the leaves overlap with each other as little as possible, which maximizes the amount of sunlight the tree is able to absorb. This Fibonacci pattern in branching is also the slowest possible way to reach the Golden Ratio, which works in favor of tree branches as it allows the branches to be as unevenly distributed as possible. This way, only a few random branches may get covered by coincidence, leaving the majority of them exposed to the sunlight (Haggerty & Ziner, 2022).
Multiscale Clustering
Despite being placed in similarly spacious groves with the same tree density, both Muir grove and Castle Creek grove of Sequoia National Park in California demonstrate a curiously different spatial pattern for similarly sized trees. Within a grove, different trees are observed to congregate differently depending on age and size while even neighboring groves do not follow the same pattern. The giant sequoia-mixed conifer forest is not just a random jumble of trees but instead grows in what is mathematically described as a mosaic of aggregations. Whilst younger trees of both mixed conifers such as white fir and sequoia trees tend to contagious (clumped) distributions, their spatial organization changes significantly with age (Bonnicksen & Stone, 1980).
The aggregation patterns of trees in the Sequoia National Park forest community change noticeably as trees mature, whilst mixed conifers tend toward uniformity and decomposition of groups, Sequoiadendron display a unique persistence of its aggregation patterns which may be perpetuated by its low mortality rate (Bonnicksen & Stone, 1980).
In order to determine the growing patterns of these trees, researchers make use of several mathematical methods such as the point to plant distance, represented by Eq. 6, which sums the square distance to the nearest tree of random points, then takes the average of these values. Under random conditions we should expect:

Where X is the mean number of trees per unit-radius circle (i.e. density). To see whether a forest is random, uniform or clumped we can compare the actual average to the expected random average using and index, represented by Eq. 7.

If the trees were randomly placed the index would be approximately 1, whereas values of <1 signal uniformity and index of larger than 1 indicate contagion (Bonnicksen & Stone, 1980).
Similarly, plant-to-plant distance compares the mean nearest-neighbor distance among trees (ra) with the expected random (Eq. 8).

If ra <re the pattern is uniform, otherwise if ra > re it is contagious.
The giant sequoia’s use of mosaic aggregations creates a heterogeneous fuel matrix that slows surface fires, allowing the forest to protect mature giant sequoias whilst simultaneously allowing regeneration in canopy gaps (Bonnicksen & Stone, 1980). This spatial complexity reduces the continuity of fine fuels, causing fires to burn in a patchy rather than uniform pattern, thus minimizing damage to large trees while still maintaining the low to moderate intensity fires necessary for seedling establishment. The persistence of large, long-lived aggregations unlike most species that gradually decompose into more uniform arrangements with age, ensures that viable seed sources remain distributed across the landscape (Bonnicksen & Stone, 1980). These persistent clusters not only facilitate the local regeneration of sequoia but also help preserve diversity across centuries by maintaining intermixing among multiple age cohorts. Thus, the stability of these aggregated structures is essential to contributing to the ecological integrity, regenerative capacity, and long-term survival of the iconic Sequoiadendron (Bonnicksen & Stone, 1980).
Tension Fork Structure
The tension fork is characterized by forces, like gravity or wind for example, that bend two connected stems away from each other, creating tensile stresses in the joint. An ordinary engineering design with a semicircular transition curve in the joint region would produce high localized notch stresses, which will lead to failure (Mattheck & Vorberg, 1991). Thus, the sequoia must optimize the shape of these joints in order to prevent such notch stresses from arising. What trees use in order to solve this issue is to instead completely homogeneously distribute Von Mises stresses across the inner contour, as seen in Fig. 6. This optimization adheres to the principle of constant mechanical stress at the surface for the most important natural load cases. Which means that no point on the surface is overloaded or underloaded, meaning every point has the same risk of breaking and thus no point is structurally weaker than another (Mattheck & Vorberg, 1991).

Fig. 6. Comparison of stress distributions in a semicircular fork joint with a naturally optimized tree fork. Note the tightly packed stress contours in the left diagram indicating the highly localized notch stresses which are source of structural failure (Mattheck & Vorberg, 1991).
In the fork, the inner contour line of the fork is most important. Although the external contour may vary widely from tree to tree, maintaining the optimum inner contour line is essential to preserve the homogenous stress state (Mattheck & Vorberg, 1991).
Additionally, the growth rings within the fork are arranged along the lines of force flow (principal stress trajectory), which are defined as lines free of shear loading. This “smart” behavior avoids dangerous shear between the growth rings, further strengthening the joint (Mattheck & Vorberg, 1991).
Thus, the geometry of the Sequoiadendron’s fork represents a natural form of topological optimization, where material is distributed only where it is mechanically needed. Through gradual adaptation and growth, the tree achieves a structure that maintains a uniform stress distribution and eliminates critical stress concentrations (Mattheck & Vorberg, 1991).
Networked Nature of Sequoia Bark Material
Sequoia bark is composed of a highly lignified and hierarchical polymer that allows for high compressive stress resistance and efficient energy dissipation. While the intermolecular bonds permitting the branching have been discussed in the second paper of this series (see Sequoia Chemistry), the networked material can also be examined with notions from graph theory. The highly hierarchical material composing the outer bark can be modeled as a network with hierarchical topology.
Common network topologies include scale-free networks where most nodes have few connections and few nodes have many connections, random networks where connections are assigned stochastically, and hierarchical networks that contain centralized nodes to which every other node or node cluster is connected. Fig. 7 below illustrates these three types of graphs.

Fig. 7. An illustration of three different types of graphs. Networks shown have (a, d) random topology (b, e) scale-free topology and (c, f) hierarchical topology (Almaas et al., 2007).
Each one of these networks responds differently to failure events, occurrences in which one or more nodes are severed from the network. The failure behavior of scale-free networks is generally robust, meaning they will likely keep their structural integrity if it is attacked at random, but the relatively many central failure points (the few very connected nodes) can make it impractical for frequent, intense stress like rockfall events in the Sierra Nevada. The robustness of scale-free networks is characterized as fragile: attacks targeting the hub nodes will make (Artime et al., 2024). It can therefore be said that the optimal network topology for high mechanical stress applications is hierarchical.
Hierarchical networks are inherently modular: they exhibit failure behavior in which either (1) one of the multiple node clusters are damaged or (2) one of the node clusters is severed from the network. This can be preferred over the many failure points of scale-free networks as their failure behavior is predictable and has only a very small probability of rendering the network ineffective. This is an advantage of the modular behavior of hierarchical networks, and it represents a highly desirable feature when it comes to resisting impact (Artime et al., 2024).
In practice, the outer, softer layer of sequoia bark is composed of “nodes” embodied by rows of rigid, highly lignified cells acting as central hubs to which non-lignified, softer tissue adheres. In Fig. 8 below, note how only the lignified tissue makes many connections, and how the fibers forming the majority of the tissue mass seen in green visibly don’t form strong bonds with each other.

Fig. 8. Photomicrograph of S. giganteum bark stained with toluidine blue, showing two rows of highly lignified fiber cells in bluish turquoise, also indicated by two arrows (Bold et al., 2020).
Note that, at large scale, hierarchical networks exhibit scale-free behavior, with the accumulation of central node points. This further enhances the network’s resilience, as it combines modularity and a certain decentralization, essentially combining the advantages of both network types (Almaas et al., 2007). Classifying biological tissues into one specific graph type isn’t straightforward, but the mechanically hierarchical nature of outer sequoia bark, as discussed in the first paper if this series, makes it interesting to study as a hierarchical network.
Conclusions
Mathematically modelling the complex behaviors and interactions of sequoia trees gives some important insights on how the tallest living organism on Earth is optimized to survive and thrive. One of these is the sequoia’s branching behavior: to resist the frequent droughts of its native habitat, the sequoia minimizes the fractal dimension of its crown, a feature that leads to less water loss by transpiration, all the while compensating for the reduced useful area for photosynthesis by growing tall and on forest floors cleared up by wildfires. To thrive in the competitive environment of the redwood forests, sequoias take advantage of human-induced and natural thinning, ensuring the development of its saplings. Taking this into account, sequoia growth rates can be modelled by the quadratic mean diameter equations. The cones of the sequoia also face a unique challenge: they must efficiently pack seeds, while the tree must maximize its light intake while branching. To solve this problem, the cone scales and branches arrange in Fibonacci spirals to optimize packing space and minimizing leaf overlap. Sequoias also use multiscale clustering to help maintain the diversity and ensure regeneration of their population. These age-size patterns help the trees protect the mature specimens from fires while keeping the group diverse maturity-wise. The tension forks employed by sequoias have stress-distribution optimized inner contours and their growth rings align with the main stress axes, helping to reduce shear stress, helping the giant tree to remain upright. Lastly, the outer bark of sequoias can be modelled as a hierarchical network in which the central nodes are high-lignin stone cells and the peripheral nodes compose the bulk of the tissue mass to help sequoias survive life-threatening rockfall impacts. In short, the sequoia makes use of mathematical principles to ensure its livelihood and exhibits behaviors that can be modelled insightfully with quantitative laws, all of which exhibit the greatness of the tall sequoia tree.
References
References
Almaas, E., Vázquez, A., & Barabási, A.-L. (2007). SCALE-FREE NETWORKS IN BIOLOGY. In F. Képès, Complex Systems and Interdisciplinary Science (Vol. 3, pp. 1–19). WORLD SCIENTIFIC. https://doi.org/10.1142/9789812772367_0001
Arseniou, G., & MacFarlane, D. W. (2021). Fractal dimension of tree crowns explains species functional-trait responses to urban environments at different scales. Ecological Applications, 31(4), e02297. https://doi.org/10.1002/eap.2297
Artime, O., Grassia, M., De Domenico, M., Gleeson, J. P., Makse, H. A., Mangioni, G., Perc, M., & Radicchi, F. (2024). Robustness and resilience of complex networks. Nature Reviews Physics, 6(2), 114–131. https://doi.org/10.1038/s42254-023-00676-y
AwkwardBotany. (2019). [Photo]. Pine Cones and the Fibonacci sequence. awkward botany. https://awkwardbotany.com/2019/12/25/pine-cones-and-the-fibonacci-sequence/
Bold, G., Langer, M., Börnert, L., & Speck, T. (2020). The Protective Role of Bark and Bark Fibers of the Giant Sequoia (Sequoiadendron giganteum) during High-Energy Impacts. International Journal of Molecular Sciences, 21(9), 3355. https://doi.org/10.3390/ijms21093355
Bonnicksen, T. M., & Stone, E. C. (1980). The giant sequoia—mixed conifer forest community characterized through pattern analysis as a mosaic of aggregations. Forest Ecology and Management, 3, 307-328.
Burns, E. E., Campbell, R., & Cowan, P. D. (2018). State of Redwoods Conservation Report. Save The Redwoods League. https://www.savetheredwoods.org/wp-content/uploads/State-of-Redwoods-Conservation-Report-Final-web.pdf
Campbell, R. (2013). Finding patterns in the redwoods: It’s easy as 1, 1, 2, 3... Save the Redwoods League. https://www.savetheredwoods.org/blog/wonders/finding-patterns-in-the-redwoods-its-easy-as-1-1-2-3/
Curtis, R. O., & Marshall, D. D. (2000). Technical Note: Why Quadratic Mean Diameter? Western Journal of Applied Forestry, 15(3), 137-139. https://doi.org/10.1093/wjaf/15.3.137
Edkins, J. (2007). Fibonacci numbers and golden ratio. Interesting numbers - Golden ratio and Fibonacci numbers. https://www.theedkins.co.uk/jo/numbers/interest/golden.htm#gold
Haggerty, N., & Ziner, N. (2022). The mathematical patterns hidden in Northeastern’s arboretum. Northeastern University College of Science. https://cos.northeastern.edu/the-mathematical-patterns-hidden-in-northeasterns-arboretum/
Hartesveldt, R., Harvey, H., Shellhammer, H., & Stecker, R. (1975). The Giant Sequoia of the Sierra Nevada. National Park Service. https://npshistory.com/series/science/giant-sequoia.pdf
Kane, J. M., & Carrasco, J. T. (2025). Tree and stand characteristics moderate wildfire severity and promote resilience in secondary coast redwood forests. Forest Ecology and Management, 596, 123078. https://doi.org/https://doi.org/10.1016/j.foreco.2025.123078
Kimberley, M., & Watt, M. (2021). A Novel Approach to Modelling Stand-Level Growth of an Even-Aged Forest Using a Volume Productivity Index with Application to New Zealand-Grown Coast Redwood. Forests, 12, 1155. https://doi.org/10.3390/f12091155
Lalemand, L. B., van Mantgem, P. J., Sherriff, R., Kane, J. M., & Teraoka, J. (2024). Sequoia sempervirens and Pseudotsuga menziesii tree growth and drought resistance following restoration thinning in secondary northern coast redwood forests of California. Forest Ecology and Management, 569, 122149. https://doi.org/https://doi.org/10.1016/j.foreco.2024.122149
Mattheck, C. P. D., & Vorberg, U. (1991). The biomechanics of tree fork design. Plant Biology, 104, 399-404.
Minarova, N. (2014). (PDF) the fibonacci sequence: Nature’s little secret. CRIS Bulletin. https://www.researchgate.net/publication/275994357_The_Fibonacci_Sequence_Nature’s_Little_Secret
Olarte, S. (2018). California, Sequoia, Nature image. https://pixabay.com//?utm_source=link-attribution&utm_medium=referral&utm_campaign=image&utm_content=3675733
Pittermann, J., Stuart, S. A., Dawson, T. E., & Moreau, A. (2012). Cenozoic climate change shaped the evolutionary ecophysiology of the Cupressaceae conifers. Proceedings of the National Academy of Sciences, 109(24), 9647–9652. https://doi.org/10.1073/pnas.1114378109
Queensland Arboricultural Association. (n.d.). How to correctly measure Diameter at Breast Height (DBH). Queensland Arboricultural Association. https://qaa.net.au/resources/calculations/correctly-measure-diameter-gbh/?srsltid=AfmBOoodGbCVEa2oCpq64v8Va6aSxDo51fwavMCmgjvZCe41_9LLBOVb
Rayonier. (2024). What is Thinning Trees, and Why Do Foresters Do It? Rayonier. https://www.rayonier.com/stories/what-is-thinning-trees-and-why-do-foresters-do-it/
Sharma, M., Amateis, R. L., & Burkhart, H. E. (2002). Top height definition and its effect on site index determination in thinned and unthinned loblolly pine plantations. Forest Ecology and Management, 168(1), 163-175. https://doi.org/https://doi.org/10.1016/S0378-1127(01)00737-X
Vasiltsov, K. (2022). Fibonacci in nature. Writing | Kirill Vasiltsov. https://www.kirillvasiltsov.com/writing/fibonacci-in-nature/