
Table of Contents
Keywords: bijugate phyllotaxis, allometry, slenderness ratio, fractal dimension, surface-to-volume optimization, structural equation modeling, Crassostrea virginica, foundational species, machine learning modeling
Abstract
Beneath its calm canopy, Rhizophora mangle, also known as the red mangrove, is a living structure shaped by mathematics. Occupying the interface between land and sea, it endures harsh environmental conditions while simultaneously providing habitat for diverse neighboring species. Its survival depends on specialized architectural traits such as bijugate phyllotaxis, which optimizes light capture through precise leaf arrangement, and modular orthotropic branching. This enables flexible growth and rapid recovery from damage. The allometric relationships between tree height, crown size, and root morphology maintain the tree’s structural stability while supporting efficient vertical growth. Prop roots offer mechanical stability in soft substrates and exhibit fractal-like branching that maximizes surface area for nutrient absorption, oxygen exchange, and habitat formation for oysters and other organisms. Its interaction with oysters creates a hierarchical foundation species system and can be modeled using structural equation modeling, known as SEM. The red mangrove also contributes to carbon productivity, with photosynthetic rates influenced by salinity, temperature, light availability, and canopy density, all of which can be quantified using machine learning models. Finally, Rhizophora mangle’s adaptations show how it can maintain ecosystem resilience and biodiversity while surviving in harsh coastal conditions.
Introduction
Rhizophora mangle is a coastal tree that occupies intertropical shorelines across North and South America, the Caribbean, and West Africa (Takvorian, 2022). Its name derives from the Greek words rhizo (“root”) and phora (“to carry”), referring to the stilt-like prop roots that suspend its trunk above water. With its arched roots and symmetrical branching, Rhizophora mangle has long captured the attention of scientists not only for its resilience but also for the mathematical precision it embeds in its form.
Unlike most trees, the red mangrove builds its life between two worlds. It grows in shallow coastal waters where tides rise and fall daily, and yet it remains firmly anchored by a web of stilt-like roots. At first glance, Rhizophora mangle appears chaotic, a tangle of roots and leaves clinging to unstable coastlines (Fig. 1). Yet beneath this apparent disorder lies an organized mathematical structure. These roots not only support the tree but also form complex patterns that shelter fish, crabs, and oysters. Because Rhizophora mangle can support entire neighboring ecosystems, many regions have begun protecting mangrove forests through conservation acts (Heemsoth, 2020).

Fig. 1. Rhizophora mangle standing in coastal waters, showing its network of prop roots (Gardenia, https://www.gardenia.net/plant/rhizophora-mangle).
Nature rarely wastes material, and Rhizophora mangle is no exception. Every curve of its trunk and every split of its roots obey principles of optimization, maximizing reach, strength, and surface area while minimizing the cost of energy. Its design offers a living example of how mathematics manifests in nature, where form and function are inseparable.
Bijugate Phyllotaxis
Phyllotaxis refers to the arrangement of leaves on a stem (Strauss et al., 2020). Plants strategically organize their leaves around the stem axis to maximize light interception for photosynthesis. The Fibonacci, or golden angle of 137.5 is the most common divergence angle and is often considered optimal for light capture. However, it was shown that other angles can be equally efficient and beneficial for plant fitness. These divergence angles are influenced by factors such as the angle of incident light, the inclination of the leaf relative to the stem, the internode length (the distance between successive leaves), leaf shape, and petiole length (the length of the leaf stalk) (Fig. 2) (Strauss et al., 2020).

Fig. 2. Factors influencing the optimal divergence angle for light capture (Own work by Eileen Lange).
The red mangrove’s phyllotaxis exhibits a modified decussate arrangement (Strauss et al., 2020). “Decussate” means “to intersect,” and this type of phyllotaxis is characterized by pairs of leaves positioned in the middle of the precedent pair, resulting in a divergence angle of 90° (Strauss et al., 2020). Like most members of the Rhizophoraceae family, red mangroves display a bijugate phyllotaxis, in which opposite pairs of leaves are initiated at the same time and are equally spaced in whorls (Strauss et al., 2020; Tomlinson & Wheat, 1979).
In red mangroves, the angle between the vertical leaf rows, called orthostichies, is always less than 90°, often approaching half the Fibonacci angle, approximately 68.75° (Fig. 3) (Tomlinson & Wheat, 1979). This pattern persists even in plagiotropic (horizontally growing) branches, resulting in a radial symmetry. Such an arrangement allows Rhizophora mangle to maximize light capture while minimizing leaf overlap, an essential adaptation for survival in dense mangrove forests (Tomlinson & Wheat, 1979).

Fig. 3. The bijugate phyllotaxis of the red mangrove (Rhizophora mangle (Red Mangrove), https://www.gardenia.net/plant/rhizophora-mangle)
Tree Architecture
The architecture of Rhizophoreae, including the red mangrove, can be described by Attim’s model (Fig. 4) (Chi et al., 2022). This model involves equivalent branches emerging at fixed angles from a monopodial trunk, characterized by a single main stem that grows vertically and continuously, with lateral branches developing along its length. Each new branch can produce additional offshoots, contributing to a repetitive and modular structure (Chi et al., 2022).
The branches are orthotropic, meaning their axes grow vertically, either continuously or discontinuously (Tomlinson, 2016). The orthotropy of red mangroves enables damaged axes to be rapidly replaced by adjacent shoots. In saplings, for instance, branch axes have been observed to convert into trunk axes, demonstrating a high degree of architectural plasticity. Branch expression in mangroves is therefore opportunistic, allowing trees to respond adaptively to environmental conditions, like by reorienting shoots to compensate for a broken main stem or by growing toward light sources (Tomlinson, 2016).

Fig. 4. Attim’s architectural model of tree growth (Santos et al., 2022).
Allometry
Beyond the architecture of its leaves and branches, the red mangrove demonstrates its uniqueness and adaptability through the development of prop-roots that emerge from its main stem (Méndez-Alonzo et al., 2015). These aerial roots provide structural support from the trunk to the ground, enabling stability even in unstable, waterlogged, or muddy substrates. The specific root architecture varies with the distance from the main stem, stem height, and crown position. These relationships can be analyzed allometrically, by establishing quantitative correlations between the tree’s dimensions and its functional properties (Méndez-Alonzo et al., 2015).
In a study conducted in a coastal lagoon in Mexico, Méndez-Alonzo et al. (2015) quantified the geometry of Rhizophora mangle roots using detailed morphological measurements (Fig. 5). The crown area was approximated as an ellipse, allowing for the estimation of crown leaning relative to structural support provided by the roots (Méndez-Alonzo et al., 2015).

Fig. 5. Morphological measurements of Rhizophora mangle: maximum stem diameter (A), minimum stem diameter (B), first-order rhizophore height (Y), first-order rhizophore length (X), and center of mass of the tree (W) (Méndez-Alonzo et al., 2015).
The mean orientation of rhizophores was analyzed in relation to crown leaning using vector analysis (Méndez-Alonzo et al., 2015). The baseline reference for measurement was north (N), defined as 0° , such that all angles (θ) were measured clockwise from this direction.
The first set of coordinate pairs represented crown orientation. Its vector was derived from the orientation of leaning (y, N = 0° ), and the hypotenuse of leaning (x), both calculated from the leaning angle (θ) and the distance (m) between the center of the main stem and the center of the crown.
The second set of coordinate pairs represented rhizophore orientation. This vector was determined from the angle of emergence of the rhizophore from the main stem (θ, N = 0° ) and the horizontal distance (m) between the stem and the point of insertion into the ground.
These two sets of coordinate pairs are expressed in Equations 1 and 2, which describe the geometric relationship between crown inclination and root orientation (Méndez-Alonzo et al., 2015):


The mean rhizophore orientation (θ) of each tree was then determined using Equation 3 (Méndez-Alonzo et al., 2015). If y was less than 0, 180° was added to ensure proper orientation.

The mean rhizophore angle was found to be 113°, pointing southeast (Méndez-Alonzo et al., 2015). The mean crown leaning was approximately 80°, slightly less than the 90° expected if the tree were perfectly upright. This indicates that the tree’s geometry is subtly adapted to environmental forces such as wind, waves, and storms. However, the deviation from vertical is small, suggesting that the red mangroves maintain a nearly straight form from base to crown, reflecting structural resistance to external stressors (Méndez-Alonzo et al., 2015).
To examine the relationship between height (H) and diameter (D) above the uppermost rhizophore, the upper limit of tree height (Hmax) and a regression constant (a) were applied, as described in Equation 4 (Méndez-Alonzo et al., 2015):

The slenderness ratio (Sr) was then calculated as the total height (H) divided by the tree’s diameter at breast height (D) (Equation 5) (Méndez-Alonzo et al., 2015).

This ratio is commonly used to evaluate tree stability. A high slenderness ratio indicates a tall, slender tree, which is more vulnerable to mechanical loads such as wind (Ige & Komolafe, 2022). Such trees often have less developed roots and shorter crowns, reflecting rapid height growth in competitive environments at the expense of crown and diameter development. On the other hand, a low slenderness ratio indicates a shorter, thicker tree with better developed roots and a larger crown, offering greater stability (Ige & Komolafe, 2022).
Analysis of Rhizophora mangle showed that, for a given diameter above the upper rhizophore, the trees tend to grow taller than expected (Méndez-Alonzo et al., 2015). This suggests that red mangroves prioritize vertical growth, likely to maximize sunlight exposure for photosynthesis, resulting in taller and slenderer individuals.
Despite their high slenderness ratio, red mangroves maintain stability due to their prop-root system, which can constitute 10-33% of the total main stem height (H) (Méndez-Alonzo et al., 2015). Furthermore, taller trees were associated with a greater number of prop roots and longer as well as higher roots (Fig. 6) (Méndez-Alonzo et al., 2015). This structural adaptation allows mangroves to combine vertical growth with mechanical stability in challenging coastal environments.

Fig. 6. Allometric relationships between tree height (H) and rhizophore morphology of Rhizophora mangle, namely (A) rhizophores per tree, (B) maximum rhizophore length, and (C) maximum rhizophore height. Adapted from Méndez-Alonzo et al. (2015) (Méndez-Alonzo et al., 2015).
This positive correlation indicates that red mangroves rely heavily on their prop-root system for stability (Méndez-Alonzo et al., 2015). For example, trees growing in unprotected areas or on unstable substrates tend to produce more rhizophores for a given trunk size and may even be shorter in height compared to individuals in sheltered locations. Therefore, the production and morphology of rhizophores are influenced not only by tree size but also by environmental conditions, including exposure to tropical storms and substrate stability (Méndez-Alonzo et al., 2015).
Finite Wood and Infinite Tasks
Rhizophora mangle faces a fundamental structural problem: it must anchor and elevate itself using limited biomass while maintaining stability across a wide, unstable sediment surface. Its trunk is supported by a complex network of prop roots that extend through mud and seawater, forming the primary system responsible for both support and nutrient transport (Fig. 7)

Fig. 7. Prop roots of Rhizophora mangle showing stilt-like support and branching near the sediment surface (Royal Botanic Gardens, Kew, 2024).
To survive, the tree must grow upward toward sunlight for photosynthesis while simultaneously expanding outward to anchor itself, breathe, and host a large community of oysters, crabs, and fish that depend on its root system as habitat. Yet the tree has finite energy and biomass, despite needing to cover a broad horizontal area for stability while also gaining vertical height for photosynthesis. This leads to the central mathematical question for this section: How can Rhizophora mangle maximize surface area using only a limited amount of root material?
Theoretical Solution 1: Cylindrical Root Growth
One simple way for Rhizophora mangle to increase surface area would be for the tree to grow a few very thick, cylindrical roots. It a root is modeled as a cylinder of radius, r, its outer surface area, A, scales with the size of that radius according to:

However, the biomass (material cost), M, of such a root increases much faster, roughly proportional to its volume as shown in Equation 7:
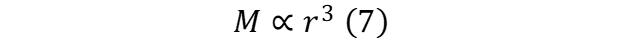
Since volume (and thus biomass) grows cubically while surface area only grows quadratically, each unit of new material yields proportionally less additional surface area. In other words, as the root thickens, the surface-to-volume ratio, A/M, decreases as follows in Equation 8:

This means that the thicker the root becomes, the less efficient it is at exchanging gases, absorbing nutrients, or hosting symbiotic organisms. For a tree like Rhizophora mangle, which depends on surface-dependent processes like oxygen diffusion through lenticels, nutrient exchange with water, and colonization by oysters and algae, this geometry is inefficient. A few massive roots would anchor the trunk securely but drastically limit the functional surface area per unit of biomass, reducing the tree’s ability to breathe and support its ecosystem.
Theoretical Solution 2: Planar Growth
It has thus been established that the tree must have a large surface area. A theoretically simple way to achieve this would be to grow a flat sheet of tissue as its roots. Its geometry would be approximately two-dimensional where the exposed surface area, A, and the length of the sheet, L, are related according to Equation 9:

where the thickness of the sheet, t, remains very small. Simultaneously, its weight, W, would still increase with the total span, roughly proportional to L3 (Equation 10).

In other words, as the sheet expands, its surface area increases quadratically with its length, but its weight increases cubically. This means that the total load acting on the sheet rises at a much faster rate than its ability to support it. Under harsh environmental forces in Rhizophora mangle’s habitat, such as waves, wind, or flowing water, the sheet would experience tensile stresses, σmax, that are proportional to its thickness as in Equation 11 (Gere & Goodno, 2012):

However, because the structure’s weight and external forces scale steeper with its span, these stresses would soon exceed the material’s tensile limit. In practice, this would cause the roots to deform, crack, or tear under its own load (Gere & Goodno, 2012). In other words, while a flat sheet would maximize A/M , it would do so at the expense of structural stability.
Rhizophora Mangle’s Solution
What we actually see as Rhizophora mangle’s genius solution is something in between: each large prop roots forks into smaller roots, which split again, and again, producing a network that is visually and statistically self-similar (Fig. 8). This is exactly what fractal geometry describes, structures that repeat a basic pattern across scales and are characterized by a non-integer dimension between a line a surface.

Fig. 8. Stilt roots of Rhizophora mangle, extending from the trunk into the mud and water in branching arches. Adapted from Kamal (2016).
Fractal Dimensions
In fractal geometry, a branching network can be described by how the number of segments, and their lengths can change with each level of branching. If each root segment is shortened by a factor r and replaced by k daughter segments, the fractal dimension D is described by Equation 12 (Kuang, 2024):

For a simple line, D=1, and for a fully filled surface, D=2. A fractal network with 1<D<2 is more space-filling than a line but does not solidify into a sheet (Kuang, 2024). This means that the network is neither 1-dimensional nor 2-dimensional, but rather of an intermediate dimension (Kuang, 2024). Such an intermediate dimension indicates that the roots fill more space than a simple line or rod, but without forming a solid sheet that would require much more biomass. A fractal dimension between 1 and 2 indicates that each branching step increases the total length and coverage of the network significantly yet still leaves gaps for water and sediment to pass through. This is exactly what Rhizophora mangle needs; to fill just enough space to stabilize the shoreline and access resources without spending infinite biomass and remaining mechanically lightweight.
In mangroves, this idea has been pushed into 3-dimensional assessment. Studies of mangroves commonly begin with a 3D scan of the root system but then compute the fractal dimension from 2D cross-sections or projections of that scan (Kamal, 2016). This is standard practice in ecological fractal analysis, because the complexity of a branching structure is captured by how densely it fills a plane. Kamal (2016) applied 3D laser scanning and image reconstruction techniques to quantify the complexity of mangrove root systems as fractals (Fig. 9).

Fig. 9. 3D reconstruction of mangrove stilt-root networks showing the branching complexity characteristic of fractal growth (Kamal, 2016).
The study found that both the individual Rhizophora mangle and entire stands exhibit fractal dimensions between 1.6 and 1.9 (Kamal, 2016). This range implies that the geometry of the tree is highly efficient. In other words, they are more space filling than a line (D=1) yet still porous, unlike a surface (D=2). Such structure allows water and sediment to flow freely while maximizing the stability of the tree and its mechanical stability (Kamal, 2016).
Each new branch or root follows the same mathematical rule as its predecessor, expanding the total surface area exponentially without requiring a proportional increase in biomass. This self-similar geometry allows the tree to achieve a remarkable balance between structural stability and ecological permeability. Thus, Rhizophora mangle turns its limited access to material into an almost infinite interface, effectively anchoring, capturing nutritious sediment, and creating microhabitats for surrounding species.
Interaction of Rhizophora mangle and Crassostrea virginica
Understanding the interactions between the red mangrove and the eastern oyster known as Crassostrea virginica (Fig. 10) requires a framework that can capture the complexity of their shared environment. Crassostrea virginica is a foundational species, meaning it supports its environment, acting as an ecological engineer, similarly to how the red mangrove does in its own habitat. Red mangroves modify hydrodynamics, sedimentation patterns, shading, and nutrient flows, while eastern oysters engineer their habitats through filtration, reef building, and nutrient processing. The two species' coexistence creates a hierarchical foundation species system where the mangrove supports the oyster, and the oyster further helps the ecosystem (Chacin et. al., 2025).

Fig. 10. Large clusters of Eastern Oysters thriving on the prop roots of a Red Mangrove tree (Matthews, 2024).
Structural equation modeling (SEM) can be used to study the relationship between the mangrove and the eastern oyster (Vovides et. al., 2021). SEM is a multivariate modeling technique (ideal for ecological systems) where direct and indirect effects merge and can be studied. It allows construction of a network that represents how different variables interact. SEM can be used to model oyster abundance and size both as latent variables, quantities that cannot be observed therefore must be inferred from other measurable quantities. To study oyster abundance, the number of live oysters on various parts of prop roots and the diameter of oyster clumps were considered. Furthermore, for studying their size, maximum shell height and average height in the lower and middle sections of each root was measured. Due to these latent variables, the SEM can account for random measurement error and any inconsistencies in oyster measurements producing a more accurate representation of patterns in oyster populations (Vovides et. al., 2021).
Predictor variables in SEM are variables which are used to estimate another, separate variable. In the oyster-mangrove relationship, these include mangrove habitat characteristics, water quality gradients, physical stressors, and geographic position within oyster habitat. The mangrove habitat variables account for prop root sizing, tree height and diameter, and the length of shoreline taken up by mangrove trees. Moreover, water quality variables describe the average variation in salinity, chlorophyll a, and turbidity (murkiness of the water). The physical stressors, sediment firmness, fetch (wave energy), and the slope of the intertidal elevation gradient represent the forces that influence viral risk and hydrodynamic stress (Vovides et. al., 2021).
Each of these predictors was connected in the SEM shown in Figure 11 through one-sided arrows representing cause and effect relationships and two-sided arrows representing connections without causality. For example, increased distance from inlets decreases mean salinity, while increasing salinity variability, which reduces oyster growth and survival. Mangrove shoreline length increases oyster abundance by providing more habitat structure and by stabilizing sediment, while finer sediment enhances oyster feeding due to higher microbial loads. FETCH, representing wave exposure, increases sediment firmness (more sand, fewer fine particles), and therefore negatively influence oysters on the ground but not necessarily oysters on prop roots, which are physically elevated and protected.

Fig. 11. Best-fitting structural equation model (SEM) describing oyster abundance on the ground near mangroves (Vovides et. al., 2021).
Figure 11 is the best fitting SEM of the factors affecting eastern oysters near red mangroves linking several different variables (Vovides et. al., 2021). The latent variable GRNDOY represents ground oyster abundance and is measured by the number of live oysters per oyster clump. It is influenced by OYABUN, which is the abundance of oysters on prop roots, since pieces of oyster clusters break off and fall to the ground. Environmental variables such as SEDIMENT (firmness), FETCH (wave exposure), SAL_MN (mean salinity), distances to inlets (INLET), and freshwater discharges (DISCH) affect oysters, reflecting the stress of wave energy, sand scour, and unstable salinity. MANG_KM, the length of nearby mangrove shoreline, indirectly increases ground oysters by boosting prop-root oysters but directly decreases them, likely due to higher predator presence. The variables in the right column of Figure 11 represent the measurement indicators used to build the latent variables for oyster size and abundance. MAXSHELLEN, BOT15SHELLLEN, and MID15SHELLLEN measure oyster size on different parts of the prop root, while BOT15_LIVOY, MID15_LIVOY, OY/PRPROOT, and CLUMPDIAM measure how many oysters are present and how large the clusters are. Furthermore, N_OY_GRND is the number of oyster clumps found on the ground in a 2×2 m quadrant, and LIVE/CLUMP is the average number of live oysters within each clump (Vovides et. al., 2021).
The numbers along the relationship arrows represent the standardized path coefficients. This means they convey the strength and nature of the relationship. A positive number means the first variable increases the second whereas a negative number means the first variable decreases the second. Moreover, a higher number (in absolute value) portrays a stronger effect.
After analyzing many SEMs, Akaike’s inflation criterion (AIC) can be used to determine which SEM best represents the relationship (Fig. 11). This criterion compares models by balancing accuracy and simplicity (Vovides et. al., 2021). The results of this test showed oyster size and abundance on prop roots is governed by both direct and indirect effects. For instance, longer shorelines with mangroves increased oyster abundance, supporting the idea mangroves help oysters by providing a safe habitat. However, on the other hand, the high salinity variability (which is correlated to being further from ocean inlets) had negative effects on oysters.
Thus, mathematical modeling using SEM can clarify the complex network of ecological forces at play in the oyster-mangrove relationship. By acknowledging many variables are acting simultaneously, the model explains how the red mangrove tree can support and sustain the eastern oyster and, together, they create a better, safer ecosystem.
Quantifying Distinctive Properties of Rhizophora mangle
Mangroves are a remarkable species that boast high carbon productivity and survival in toxic and saline environments. They play a vital role in absorbing, transforming and storing atmospheric CO2 into coastal sediments for a long period of time. This enhances ecosystem health and supports biodiversity (Alongi, 2014). Similarly, their distinctive propagules are viviparous and float away until they anchor and produce dense prop‑root structures that spread laterally across shifting mudflats, enabling stable vertical and horizontal expansion under tidal influence (Sousa et al., 2007). Modeling and quantifying the unique growth and productivity traits of red mangroves provides insight about the factors influencing their survival, helping us better understand how mangroves survive and thrive in rough environments.
Mangrove Carbon Productivity Modeling
In this section, we will look at an analysis of gross primary productivity (GPP) of the red mangrove using a machine learning-based mangrove carbon production model (ML-MCP). This model incorporates various stress indicators such as sea water level (SWL), diurnal temperature range (DTR), salinity index (SI), vapor pressure deficit (VPD), temperature influence index (TI), canopy quantum yield (E0), and the light-limited photosynthetic rate (PI) to provide a highly precise predictive model that enables mapping and monitoring carbon production of mangroves. This allows for better understanding of the carbon sinking quality of mangroves and its connection to multiple environmental factors (Alsafadi et al., 2025). A short overview of the factors used in the machine learning process follows.
Salinity Index (SI)
Salinity is a stress factor that can negatively impact the ability of mangroves to take in sufficient amounts of water by reducing the water pressure and inducing osmotic pressure. The salinity index helps to quantify the effect of the salinity on stomatal conductance, represented by a monotonically decreasing quadratic curve. It is calculated using the following relationship (Eq. 13):

Where SI is the salinity index, S is the salinity of the soil or tide, and st is the salinity threshold at 80 parts per thousand (ppt) for mangroves. Thus, a higher SI indicates a smaller S to st ratio (Alsafadi et al., 2025).
Temperature Influence Index (TI)
The photosynthetic rate decreases with temperatures higher or lower than optimal because of the effect on enzymatic activity (Yamasaki et al., 2002). The effect of the temperature can be modeled using Equation 14:

Where T is the local temperature (Alsafadi et al., 2025) and the constants are temperature coefficients obtained from data fitting (Alsafadi et al., 2025).
Canopy Quantum Yield (E0)
Canopy quantum yield is a measure of the efficiency of a mangrove forest to turn light into fixed carbon during photosynthesis. It is measured in units of grams of carbon fixed per megajoule of light energy. The quantum yield is a piecewise function because it changes based on how dense the canopy is. It is represented by Equation 15:

Where LAI represents leaf area index and qi are constants determined from red mangrove data fitting, in this case q1=-0.258, q2=0.9752, q3=0.624, q4=-1.551. The E0 decreases as the canopy gets denser, which is captured by the second piece of the function. This allows to model how the shading of the leaves in a dense canopy can affect the quantum yield of the red mangrove tree (Alsafadi et al., 2025).
Light-limited Photosynthetic Rate (PI)
This variable represents the maximum rate of photosynthesis given the availability of light. It highlights the potential of a plant to convert energy into biomass. It is calculated using Equation 16:

Where E0 is the canopy quantum yield and I is the incident shortwave radiation flux (mainly radiation from the sun) (Alsafadi et al., 2025). The radiation flux is the energy passing through a surface per unit of time (Robertson & Frédéric Vitart, 2019).
Other Factors
The other factors that were used in modeling GPP were SWL which is an observed variable, DTR, which is the difference between the daily maximum and minimum of air temperature (Cheng et al., 2014), and VPD, which is the difference between the amount of moisture the air can hold when saturated (saturation vapor pressure) and the actual amount of moisture the air holds (actual vapor pressure) (Shuyang, 2014).
Machine Learning Modeling
While linear models provide a good prediction, significant improvements can be made using a machine learning model that is equipped with various modeling methods such as Extreme gradient boosting (XGBoost), Random tree forest (RF), Multilayer Perceptron (MLP), and a Support vector machine (SVM). XGBoost is used for regression tasks, it boosts gradients from weaker learners to provide prediction accuracy. It builds an ensemble of trees in a sequential manner where each new tree’s errors are corrected. RF is used as a classification tool; it builds a forest of decision trees trained on random subsets of data and averages their predictions to reduce overfitting. MLP is a type of artificial neural network with multiple layers of interconnected neurons that learn complex nonlinear patterns in data. SVM classifies data by finding the optimal plane that maximizes the margin between different classes in a high-dimensional space, in other words, separates data into groups by drawing the best possible line or boundary between them. Further discussion of the details of these machine learning algorithms is outside the scope of this review, but the results of the predictions are gathered using a voting regressor (VR) and provide useful insight into how different factors influence the red mangrove’s carbon productivity (Alsafadi et al., 2025).
The results indicate that the factors in the red mangrove carbon productivity can be positive or negative effects. The most significant positive effect corresponded to TI and PI, indicating that as PI and TI increase, GPP also increases. The negative effects are SI and E0, which means if these variables decrease, GPP will increase. Among these effects, the quantum yield E0 has the strongest negative effect on GPP and PI has the strongest positive effect on the carbon productivity (Alsafadi et al., 2025). Other variables did not significantly affect GPP. Together, these trends help explain how red mangroves respond to environmental stress and which conditions most strongly boost or restrict their carbon-sequestration capacity. Accordingly, several biological and ecological countermeasures have evolved to mitigate the negative effects of SI and E₀. For instance, to counter high salinity (SI), red mangroves employ ultrafiltration at the root level and selective ion exclusion to maintain osmotic balance. To offset reductions in quantum yield (E₀), they protect and stabilize their photosynthetic machinery through mechanisms such as enhanced antioxidant production, repair of PSII reaction centers, and pigment adjustments that optimize light harvesting under stress. These adaptations help maintain GPP even under challenging environmental conditions.
Conclusion
Rhizophora mangle is constantly designing for its growth, stability, and survival within a shifting, saline world. The tree must divide its limited biomass across multiple tasks, and each adaptation requires a mathematical solution to that constraint.
The tree must intercept as much sunlight as possible in a crowded canopy without shading its own leaves. Its design solution is a bijugate phyllotaxis that fixes leaf pairs at a non-random divergence angle. This geometric configuration optimizes light capture while minimizing overlap of the leaves. Furthermore, to survive, the tree must be tall enough to reach sunlight but also remain anchored and oxygenated in unstable, waterlogged soil. Its design solution is a fractal root network, a self-similar geometry that expands surface faster than it uses biomass. In addition, the mangrove must maintain stability and productivity within its dynamic coastal ecosystem. Its solution is to integrate with another foundational species through a mathematically balanced relationship modeled by structural equation modeling. The red mangrove provides substrate and protection; the oyster filters and recycles nutrients. Their mutual dependence constitutes a co-engineered system quantified through direct and indirect path coefficients. Finally, the tree must continue fixing carbon under fluctuating salinity, light, and temperature. Its design solution is a physiological feedback system expressible through mathematical modeling. By adjusting variables such as canopy quantum yield, temperature influence, and salinity index, Rhizophora mangle continuously recalibrates its photosynthetic efficiency.
Through these mathematical design solutions, Rhizophora mangle transforms environmental constraints into solvable equations. Its survival is not accidental, but rather, algorithmic and a living demonstration of how nature engineers integrate mathematics into their very survival.
References
References
Alongi, D. M. (2014). Carbon Cycling and Storage in Mangrove Forests. Annual Review of Marine Science, 6(1), 195–219. https://doi.org/10.1146/annurev-marine-010213-135020
Alsafadi, K., Srivastava, A. K., Halder, K., Wang, F., Yang, S., & Cao, W. (2025). A machine learning framework for modeling and upscaling mangrove carbon productivity (ML-MCP). Agricultural and Forest Meteorology, 375, 110821. https://doi.org/10.1016/j.agrformet.2025.110821
Chacin, D., Bell, S., & Stallings, C. (2025, February). Red mangrove (Rhizophora mangle) roots serve as additional valuable habitat for the eastern oyster (Crassostrea virginica) in a subtropical estuary. Science Direct. https://www.med.upenn.edu/pmi/events/https-www-sciencedirect-com-scienc…
Cheng, J., Xu, Z., Zhu, R., Wang, X., Jin, L., Song, J., & Su, H. (2014). Impact of diurnal temperature range on human health: A systematic review. International Journal of Biometeorology, 58(9), 2011–2024. https://doi.org/10.1007/s00484-014-0797-5
Chi, F., Streit, K., Tavkhelidze, A., & Kurth, W. (2022). Reconstruction of phyllotaxis at the example of digitized red mangrove (Rhizophora mangle) and application to light interception simulation. in silico Plants, 4(1). https://doi.org/10.1093/insilicoplants/diac002
Gardenia. (n.d.). Rhizophora mangle (red mangrove). Gardenia.net. https://www.gardenia.net/plant/rhizophora-mangle
Gere, J. M., & Goodno, B. J. (2012). Mechanics of materials (8th ed.). Cengage Learning. https://mechfamily-ju.com/storage/images/files/file_1731426546RLh80.pdf
Heemsoth, A. (2020). Mangrove Tannin: What is it? https://www.livingoceansfoundation.org/mangrove-tannin-what-is-it/
Ige, P. O., & Komolafe, O. O. (2022). Tree Slenderness Coefficient Models for Biodiversity Conservation in International Institute of Tropical Agriculture Forest Ibadan, Nigeria.
Kamal, S. (2016). Assessing structural complexity of mangroves and its implications for ecosystem services (Doctoral dissertation, Griffith University). https://doi.org/10.25904/1912/3225
Kamal, S. (2016). Figure 2.4. Aligned 3D models of R. stylosa stilt roots with a Kinect (violet) and a terrestrial laser scanner (pink) [Figure]. In Assessing structural complexity of mangroves and its implications for ecosystem services (Doctoral dissertation, Griffith University). https://doi.org/10.25904/1912/3225
Kuang, Q. (2024). Fractal dimension: Introduction, example, and application (U.U.D.M. Project Report No. 2024:18) [Bachelor’s thesis, Uppsala University]. DiVA Portal. https://www.diva-portal.org/smash/get/diva2%3A1880660/FULLTEXT01.pdf
Matthews, B. (2024, July 10). Bailey-Matthews National Shell Museum & Aquarium. Facebook. https://www.facebook.com/shellmuseum/posts/in-a-healthy-environment-the…
Méndez-Alonzo, R., Moctezuma, C., Ordoñez, V. R., Angeles, G., Martínez, A. J., & López-Portillo, J. (2015). Root biomechanics in Rhizophora mangle: anatomy, morphology and ecology of mangrove's flying buttresses. Ann Bot, 115(5), 833-840. https://doi.org/10.1093/aob/mcv002
Rhizophora mangle (Red Mangrove). Gardenia. Retrieved November 4 from https://www.gardenia.net/plant/rhizophora-mangle
Royal Botanic Gardens, Kew. (2024). Rhizophora mangle L. [Photograph]. Plants of the World Online. https://powo.science.kew.org/taxon/urn:lsid:ipni.org:names:30061148-2
Robertson, A. W., & Frédéric Vitart. (2019). Sub-seasonal to seasonal prediction : The gap between weather and climate forecasting. Elsevier Inc.
Santos, E. R., Vestena, L. R., & Belmonte Serrato, F. (2022). The Role of Yerba Mate (Ilex paraguariensis) in the Redistribution of Rainfall by Interception. RAEGA - O Espaço Geográfico em Análise, 55, 78-92. https://doi.org/10.5380/raega.v55i0.81030
Sousa, W. P., Kennedy, P. G., Mitchell, B. J., & Ordóñez LB. M. (2007). Supply-side ecology In Mangroves: Do propagule dispersal and seedling establishment explain forest structure? Ecological Monographs, 77(1), 53–76. https://doi.org/10.1890/05-1935
Strauss S, Lempe J, Prusinkiewicz P, Tsiantis M, Smith RS. Phyllotaxis: is the golden angle optimal for light capture? New Phytol. 2020 Jan;225(1):499-510. doi: 10.1111/nph.16040. Epub 2019 Aug 2. PMID: 31254398.
Shuyang, S. (2014, December 30). Vapor pressure. Chemistry LibreTexts. https://chem.libretexts.org/Bookshelves/Physical_and_Theoretical_Chemistry_Textbook_Maps/Supplemental_Modules_(Physical_and_Theoretical_Chemistry)/Physical_Properties_of_Matter/States_of_Matter/Properties_of_Liquids/Vapor_Pressure
Takvorian, M. (2022). Rhizophora mangle. Retrieved October 15 from https://animaldiversity.org/accounts/Rhizophora_mangle/
Tanzania Journal of Forestry and Nature Conservation, 91(1), 20-31. https://www.researchgate.net/publication/359437980_Tree_Slenderness_Coe…
Tomlinson, P. B. (2016). The Botany of Mangroves. Cambridge University Press.
Tomlinson, P. B., & Wheat, D. W. (1979). Bijugate phyllotaxis in Rhizophoreae (Rhizophoraceae). Botanical Journal of the Linnean Society, 78(4), 317-321. https://doi.org/10.1111/j.1095-8339.1979.tb02574.x
Vovides, A. G., Wimmler, M.-C., Schrewe, F., Balke, T., Zwanzig, M., Piou, C., Delay, E., López-Portillo, J., & Berger, U. (2021, May 5). Cooperative root graft networks benefit mangrove trees under stress. Nature News. https://www.nature.com/articles/s42003-021-02044-x