Table of Contents
Keywords: oak, Quercus, mutualistic relationships, growth, fractal geometry, branching angles, Fibonacci sequence
Abstract
Oak trees, renowned for their extraordinary century-long lifespans, owe their endurance to evolutionary design solutions that can be explained through mathematical principles. This paper examines how the growth pattern of oaks follows optimized scaling relationships that balance mechanical stability and resource efficiency over time. The architecture of branches reveals fractal patterns and ideal angles that enhance light capture while minimizing mechanical stress, contributing to structural resilience. Similarly, the fractal geometry and venation of oak leaves prove to be examples of efficient spatial organization and fluid transport networks that maximize photosynthetic output. Finally, the mutualistic relationships between oaks and ectomycorrhizal fungi can be modeled as dynamic systems of resource exchange, which helps maintain equilibrium across changing environmental conditions. Together, these mathematical frameworks explain how evolution allows oaks to persist, adapt and thrive as a dominant species in diverse ecosystems for millions of years.
Introduction
As Galileo Galilei once said, “The book of nature is written in the language of mathematics” (Galilei, 1957). Patterns, sequencing, and geometry are abundant in nature and explain numerous natural phenomena, from the formation of snowflakes to the spirals of a galaxy. The beauty of mathematics and the symmetry found in almost all organisms are inherently intertwined. Oak trees (Quercus), with their imposing size and longevity, display this symmetrical beauty within the growth of their branches and the venation patterns of their leaves. The mathematical principles behind the inner workings of the tree, as well as their mutualistic relationships with other organisms, have long served as evolutionary advantages that have ensured their survival. (see Oak Physics for an extensive introduction on Quercus)
Oak Tree Growth Style
Oak Diameter Growth
Within the Quercus genus, growth rates vary from one species to the next. An influential factor of diameter growth is the tree’s crown (Shifley, 2004). A tree’s crown class (dominant, codominant, intermediate or overtopped) describes the position of an individual tree in the forest canopy (Fig. 1) and creates differences between species (Fig. 2) (DeYoung & Sutton, 2016, p. 129; Shifley, 2004). Figure 2 shows the importance of crown class, as a dominant or codominant oak will grow faster in diameter than an overtopped or intermediate oak (Shifley, 2004).
Dominant trees extend above the general level of the canopy and usually have the largest crowns in the stand. Codominant trees make up the general level of the canopy and are shorter than dominant trees. Intermediate trees are just below the general canopy level and are generally narrow and/or one-sided, and shorter than dominant and codominant trees. Overtopped, or suppressed, trees are well below the general canopy level, and their crowns are generally short, sparse, and narrow (DeYoung & Sutton, 2016, pp. 129-130).

Fig. 1. The overall shape of the different crown classes, where “D” refers to the dominant class, “C” refers to the codominant, “I” refers to the intermediate and “S” refers to the suppressed (or overtopped) crown class (DeYoung & Sutton, 2016, p. 130).

Fig. 2. The effect of tree crown class on diameter growth between oak species, where dbh is the diameter at breast height (Shifley, 2004).
Tree crown class results from competition between growing trees in a finite space. The average annual diameter at breast height (dbh) growth for a stand tree (a contiguous area that contains several trees that are relatively homogeneous or have common characteristics) decreases as stand age and basal area increase (Brack, n.d.; Shifley, 2004). However, the dominant and codominant trees that are well positioned in the canopy continue to grow rapidly, affecting those with smaller or crowded crowns. Therefore, even if a tree achieves a dominant or codominant crown class it must maintain its position in the canopy, or it will eventually lose to competitors (Shifley, 2004).
Thinning and Diameter Growth
Crown class can be manipulated by thinning, which is the felling or removal of certain trees in a stand to improve the quality of the remaining stand (Stewardship and Outreach Section Department of Natural Resources, n.d.; Shifley, 2004). Dominant and codominant trees will exhibit increasing diameter growth, across a wide range of diameters and ages, as a response to increased thinning intensity. It will often take two years for maximum diameter growth response to thinning. Thinning allows trees to increase their crown area and capture growing space allowing them to maintain faster growth rate for years. However, trees with small, poorly formed crowns, such as intermediate and overtopped crown classes, may not respond to thinning, or the response may be delayed by three to five years, but when stands are very young these crown classes are more likely to respond to thinning with increased diameter growth than are larger trees. Furthermore, oaks in stands less than 10-years old may not increase their diameter growth in response to thinning, so a variable response has been seen in dominant and codominant trees of such an age (Shifley, 2004). Dominant and codominant trees, unlike intermediate and overtopped trees, receive more sunlight due to their height, which allows them to grow more (DeYoung & Sutton, 2016, pp. 129-130).
Oak Height Growth
The height growth of dominant and codominant oaks is less affected by stand density, unlike diameter growth. Different oak species exhibit different height growth patterns; scarlet and black oaks grow rapidly at first but slow down after 50 or 60 years, while the white oak will be 3.048 to 4.572 m taller than the black oak after 100 years. Crown class not only affects diameter growth, but also height growth, where intermediate and overtopped trees are affected by competitors. Oaks that are unable to maintain a favorable crown position (dominant or codominant) may become shorter (Shifley, 2004).
A study done by Hilt and Dale attempted to find equations predicting height of an even-aged upland oak. For a logical equation, they tried to meet the following conditions: (1) height equals breast height (1.37 m) when dbh is zero, (2) height increases as a decreasing rate as dbh increases, (3) height increases at a decreasing rate for a given dbh as age increases, and (4) height increases for a given dbh and age as site index increases. The final equation (Eq. 1), which satisfied these conditions most and followed the site curve data of Figure 3 was the following:

Where Hs is the mean height of the site trees, A is the stand age and S is the site index (Hilt & Dale, 1982).

Fig. 3. Curve of height as a function of age and site index, from which Equation 1 was based off (Hilt & Dale, 1982).
Furthermore, since growth patterns differ from one species to another a study conducted by McCreary on growth patterns of blue and valley oak seedlings showed the following results. The average height increment of blue oak seedlings in the first year was approximately 25 cm, and after that the average was over 2.3 m in height (Fig. 4). For the last two years of the study the first flush of growth was about two weeks with relatively little height increment, and by mid-April most seedlings had stopped elongating. In year 3, the second flush increment accounted for 68% of total height growth, and 83% in year 4 (McCreary, 1991).

Fig. 4. Average total height of blue oak seedlings each year for four years (McCreary, 1991).
In the case of the valley oak, the average yearly height growth was a little larger than that of the blue oak and the height reached after three years was close to 2 m (Fig. 5). A similar general growth pattern of that of the blue oak was observed for the valley oak, but there was greater variability in the valley oak seedlings growth pattern than the blue oak ones. For example, from April to mid-June of year 2 and 3 the valley oak seedlings were elongating, unlike the blue oak where there was a three-week period around mid-April where the seedlings were inactive (McCreary, 1991). These results show the differences in growth patterns within the Quercus genus which are due to the species characteristics and its interactions with its environment. Oak trees tend to grow fast at the beginning of their life, and then their growth rate slows down but does not fully stop; however, that is not the case for all organisms. Although some do keep growing like the oak tree, others, such as mammals, will hit a plateau (Clatterbuck, 2002)

Fig. 5. Average total height of valley oak seedlings each year for three years (McCreary, 1991).
Architecture of Oak Branches
Space-Filling Fractal Growth
The remarkable spread of an oak tree’s canopy (Fig. 6), often forming a wide dome shape, is not random.

Fig. 6. Photograph taken by Barbara Taylor of a southern live oak, more specifically an Angel Oak (Quercus virginiana) found in South Carolina, USA, with a large arching canopy and horizontally extended branches (Taylor, n.d.).
In fact, it reflects a mathematical principle known as fractal growth. Oaks possess a branching process that repeats similar geometric rules at multiple scales, from major limbs to twigs. Each new limb forms at a specific ratio of length and angle relative to its parent branch. This relationship derives from Lindenmayer systems (L-systems), which mathematically describe recursive plant growth (Prusinkiewicz & Lindenmayer, 1990). A simplified expression of this pattern can be modeled as the following Equation 2:
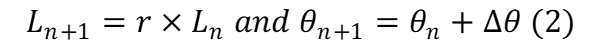
where Ln is the length of a parent branch, r is the proportional reduction in length (typically around 0.7-0.8 in oaks), θn is the angle of a parent branch, and Δθ represents the angular divergence between successive limbs (Prusinkiewicz & Hanan, 1989). This pattern repeats itself at progressively smaller scales, producing a self-similar structure, so the shape of the whole oak canopy can be visualized with the shape of its smaller branches. Such self-similarity is described by the fractal dimension D (Jiménez-Guzmán & Vega-Peña, 2024), a value between 1 and 3 that quantifies how densely the branches fill three-dimensional space (where D=1 represents a line-like form and D=3 indicates a fully space-filling structure). According to Arseniou and MacFarlane (2021), the mean of the fractal dimensions of a wide variety of trees in their study is estimated to be 2.277 (Arseniou & MacFarlane, 2021). However, oak fills the space more effectively than other trees by having a higher fractal dimension that ranges from 2.35 to 2.75 (Jiménez-Guzmán & Vega-Peña, 2024). This explains their distinctive broad, dome-shaped canopies, which is a geometric strategy optimized for light interception in open environments where sunlight arrives from many directions.
The fractal pattern ensures that the ratio between light-intercepting area and branching volume remains nearly constant. For oaks, this balance means that as the tree expands outward, it maintains an efficient photosynthetic area without excessively increasing biomass (Binkley et al., 2013). In other words, it allows the tree to “fill” its environment, maximizing energy capture while minimizing structural instability. This growth pattern likely emerged as a design solution to environmental constraints. Early oaks that competed in dense forests grew vertically, but as many adapted to open areas like savannas and fields (Kremer & Hipp, 2019), the ones that developed horizontally spreading canopies gained an advantage in light capture and mechanical balance.
Structural Strength Through Branching Angles
As for the geometry of oak boughs, it can be explained using torque equilibrium, a principle from physics that describes how rotational forces act around a pivot. The bending moment M (or torque) exerted on a branch is defined by Equation 3 for the torque:

where F is the downward force of the limb’s mass or wind load, R is the length of the branch from its base, and θ is the growing angle relative to the trunk. When the angle is small, meaning the branch grows closer to the trunk, sin(θ) is also small, resulting in a lower bending moment (Günay & Sönmez, 2003). This geometry minimizes torque and maximizes structural stability, as less rotational force acts on the limb’s base. On the other hand, as the branching angle increases and approaches a horizontal orientation, sin(θ) approaches one, producing the maximum possible torque for a given length and load. This increase in torque makes the branch more susceptible to bending and failure under wind or weight, but it allows for greater lateral spread and light capture (As et al., 2017). Due to this mechanical trade-off, many trees have evolved to favor angles that reduce excessive torque by minimizing the sine component, a structural solution that prevents their trunks from splitting under high loads. Most trees minimize torque, and therefore bending stress, by keeping R small with narrow branch angles of less than 45°. However, a total of 79% of oaks deviate from this usual optimal geometry by growing broad horizontal limbs at 45°-67.5° (32%) and 67.5°-90° (47%), thus increasing R significantly (Hodžić & Ballian, 2020). Mathematically, this should increase the bending moment, but oaks compensate by producing tension wood, the specialized reaction wood oaks generate on the upper side of a limb, effectively increasing the second moment of area I and enhancing resistance to bending. The bending stress is described by the following Equation 4:

where σ is the bending stress experienced at the outer edge of the branch, M is the bending moment from equation (3), y is the distance from the neutral axis (the line through a cross-section of a branch experiencing zero stress), and I is the second moment of area, a geometric property that represents how the cross-section’s shape resists bending (Burgess & Pasini, 2004). Oaks minimize the resulting stress by growing thick boughs that increase I, and by forming dense wood tissue that reinforces their limbs (As et al., 2017). Evolutionarily, this became a design solution to different ecological pressures. As previously mentioned, in open habitats where wind and light competition are intense, wide-spreading limbs with bigger θ allow for greater canopy coverage and light interception, even at the cost of higher torque (Mediavilla & Escudero, 2023). To prevent failure under these conditions, using the photosynthetic advantages of larger canopies, oaks invest in thicker branches that mechanically balance the added bending moment. In fact, the southern live oak shown in Figure 6 is a good example of this principle in practice. Native to the coastal plain region in South Carolina, these trees develop wide horizontally spreading crowns that can reach up to 45.7 meters in diameter, which is nearly twice the length of a tennis court (National Wildlife Federation, n.d.). In contrast, oaks exposed to strong winds often produce steeper limbs with smaller θ to reduce bending stress and prevent structural damage. The reduction in sin(θ) directly lowers both the torque and the bending stress, allowing the tree to resist dynamic loads more effectively without the need for excessive wood thickening (Hodžić & Ballian, 2020).
Mathematical Modelling of Oak Leaf Structure
The morphology and spatial organization of oak tree leaves reveal how deeply mathematical principles are woven into nature. Their self-similar patterns, lobed edges, and spiralling arrangement provide a framework for understanding the beauty and efficiency of oak leaf growth. These patterns are not random either — they are evolutionary adaptations that ensure the tree makes the best use of limited resources such as light, water, and space, to survive and thrive.
Fractal geometry of oak leaves
Fractal geometry is defined as a branch of mathematics that studies irregular or fragmented geometric structures that exhibit self-similarity (i.e., the property of an object having the same shape when viewed at different scales), allowing for a more detailed description of spatially nonuniform phenomena in nature (Al-Kadi, 2017). It is characterized by shapes that are unable to be represented by classical Euclidean geometry and possess no characteristic scale.
Oak leaves are characterized with a pinnate venation, indicating that they have a single, prominent vein running through the center of the leaf, and smaller veins branching out towards the leaf edges, as seen in Figure 7 (Hernandez & Park, 2022). This dendritic branching process repeats down to the finest levels, exhibiting fractal patterns and the same mathematical rules at each degree of branching.

Fig. 7. Macrophotograph of a Quercus robur leaf, depicting the dendritic venation pattern (Conge, n.d.).
The venation pattern of oak leaves can be modeled by Murray’s Law (Eq. 5), which describes the relationship between the radius of a parent vessel (rp) and its daughter branches (rd) (Price et. al., 2013).

In a study conducted by Price and colleagues, they found that across all oak and similar species leaf vein networks, both radius tapering and the ratio of daughter to parent branch areas for leaf veins follow closely to the expected results from Murray’s Law. Thus, modelling oak leaf venation with Murray’s Law suggests that leaf venation networks are optimized for efficient fluid transport by balancing hydraulic resistance and vessel number (Price et al., 2013). This also confirms that the fractal geometry of oak leaves’ venation contributes greatly to the tree’s efficiency of transporting water and nutrients to all regions of the leaf.
Furthermore, many common oak species such as white oak (Quercus alba) or red oak (Quercus rubra) are easily recognized by their distinctive, lobed shaped leaves, with a bristle-tipped, jagged edge, as seen in Figure 8 (Keeler, 2005). This specific shape exhibits aspects of self-similarity and can be modeled using fractal dimension analysis. Fractal dimension is a non-integer value used to quantify the complexity and “jaggedness” of the oak leaf’s outline. This is accomplished through a “box-counting method”, where a grid of boxes is superimposed over an image of the leaf, and the number of boxes containing a part of the leaf are counted at increasingly finer scales (Ng et al., 2002). A subsequent log-log plot of the resolution scale () vs. the number of windows occupied (N) is produced to determine the fractal dimension, or the slope of the graph (D). This method ensures a more accurate representation of the leaf’s roughness than what is possible through Euclidean geometry modelling. The fractal dimension of any object can also be produced mathematically, as seen below in Equation 6 (Bayirli et al., 2015).

In a study conducted by Bayirli et al. to determine different plant leaves’ fractal dimensions using the box-counting method, Quercus alba leaves were found to have a fractal dimension of 1.711, as estimated below in Figure 8 (Bayirli et al., 2015). This fractal dimension indicates that a given object is more complex than a one-dimensional line but less complex than a two-dimensional plane. Thus, a value of 1.711 suggests that the outline of the oak leaves have a significant degree of space-filling and structural elaboration, which is an evolutionary adaptation for efficient water and nutrient transport (Ng et al., 2002).

Fig. 8. Example modeling of fractal dimension of Quercus alba leaves using the box-counting method, adapted from Bayirli et al. Created by A. Cheng, 2025.
Furthermore, they found a positive linear correlation between fractal dimensions of leaves and the cell density of the image surface, shown in Figure 9. After determining that the cell density value of the surface of Quercus alba leaves was the greatest of all ten species examined, they deduced that Quercus alba has very little geometric difference between leaves (Bayirli et al., 2015). This also implies a greater degree of complexity and spatial organization in how the cells are arranged within the leaf structure.

Fig. 9 The relationship between fractal dimension (D) and cell density () of the image surface of various tree species (Bayirli et al., 2015).
Fibonacci Sequence for Their Arrangement on the Stem
Phyllotaxis is the spatial arrangement and geometry of leaves on a given stem, characterized by the divergence angles between the organs, with the most common angle (i.e. the golden angle) being 137.5o (Kuhlemeier, 2007). In nature, the golden angle ensures each leaf receives the maximum amount of sunlight and minimizes overcrowding or self-shading. Additionally, the principle of phyllotaxis is crucial for oak trees as it aids in the efficient transport of water and nutrients between the leaves and the main stem (Okabe, 2024). Oak trees exhibit spiral phyllotaxis, which is often associated with the Fibonacci sequence - a series of numbers where each number is the sum of the two preceding ones (Brain, 2024). It is represented by the formula below, and its relationship to the golden ratio enables the creation of spiral shapes.

Oak trees have a 2/5 phyllotaxis, as seen in Figure 10 (a), meaning that every fifth leaf emerges above one below it after two turns of a spiral of successive leaves, and thus, five straight ranks will be visible along the stem (Okabe et al., 2019). This follows with the Fibonacci sequence rules, as 2/5 is obtained from 1/2 and 1/3 after adding their numerators and denominators, respectively. Successive leaves on the developed stem will make constant angles of 144o, determined from 360o x ⅖ = 144o (Okabe, 2015). However, the divergence angle at the shoot tip is equal to the golden angle of 137.5o, as seen in Figure 10 (b), allowing neighboring leaves to form five winding spirals at the tip.

Fig. 10. Modified figure from Okabe and colleagues of two types of leaf arrangement: whorled (a) and spiral (b) phyllotaxis. (a) 2/5 phyllotaxis of mature oak leaves, with five vertical rows denoted with dotted lines. (b) At the shoot tip (center circle), leaves form two (dashed) and three (dotted) curved rows as they are arranged at a divergence angle of 137.5o (Okabe et al., 2019).
The Mathematics of Mutualism
“Rooted in Chemistry: Chemical Mechanisms Within Oak Trees” describes the mutualistic relationship between oaks and mycorrhizal fungi, focusing on the chemical basis of nutrient exchange. Ectomycorrhizal fungi (EMF) surround the oak’s roots and extend a network of hyphae (the Hartig net) into the soil, allowing for the exchange of carbon, nitrogen, phosphorus, and micronutrients (Martin & van der Heijden, 2024). While this chemical foundation explains how these exchanges occur, the persistence of this relationship over generations can be understood through mathematics. Modeling this relationship using concepts from game theory, evolutionary stability, and network theory helps explain why oak-fungi mutualism remains advantageous for both partners.
Mutualism as a Strategic Game
The oak-fungus relationship can firstly be described using game theory. As explained by Dixit et al. (2015), game theory provides a mathematical framework for analyzing how the choices of one participant affect the outcomes of others, allowing interactions between “players” to be modeled and compared strategically. In EMF interactions, the players are the oak and its fungal partner. The oak provides photosynthetically derived carbon to the fungus, while the fungus supplies essential nutrients such as phosphorus and nitrogen in return. Each partner adjusts how many resources to share and to keep, with every exchange affecting its overall fitness. Over evolutionary time, these trade-offs determine strategies that each player uses to achieve long-term survival and reproductive success while conserving energy.
This reciprocal exchange can be compared to the Prisoner’s Dilemma, one of the best-known models in game theory. In this game, both players gain the most when they cooperate, but each is tempted to “cheat” by holding back resources while taking advantage of the other’s effort. When both cooperate, the players share a moderate benefit. When one cheats and the other cooperates, the cheater gains more while the cooperator loses, and if both cheat, both gain nothing (Dixit et al., 2015). The same logic applies to the oak-fungus relationship. Both partners thrive when they exchange resources freely, yet short-term conservation of carbon or nutrients could disrupt the partnership (Archetti & Scheuring, 2003; Archetti et al., 2011). This payoff can be demonstrated with arbitrary numbers (for example, +5, +8, −2, and 0) that have relative magnitudes showing how different choices affect the outcome (Dixet et al., 2015). This can be illustrated using the following payoff matrix (Table 1):
Table 1. Conceptual payoffs between oak (vertical) and fungi (horizontal), created by J. Neufeld, 2025.
Fungus: High Investment (Generous nutrient exchange) | Fungus: Low Investment (Minimal nutrient exchange) | |
|---|---|---|
Oak: High Investment (High carbon allocation) | (+5, +5) Mutual cooperation | (-2, +8) Fungal cheating |
Oak: Low Investment (Minimal carbon allocation) | (+8, -2) Oak cheating | (0, 0) Mutual defection |
This 2×2 matrix captures the central evolutionary stress in the oak-mycorrhizal mutualism, mirroring the Prisoner’s Dilemma logic, where cooperation is collectively best but individually risky. Mathematically, the short-term possible payoffs are ranked:
T > R > P > S
T (temptation to defect) represents the short-term benefit of cheating, R (reward) is the gain from mutual cooperation, P (punishment) is the outcome when both defect, and S (sucker’s payoff) is the loss suffered by a player when the other cheats (Dixit et al., 2015). While cheating yields a higher immediate payoff (T > R), the combined benefit of mutual cooperation, represented as 2R, exceeds any single act of cheating. Over a long period of time, natural selection favors this repeated cooperation, since stable exchange between oaks and fungi provides greater long-term fitness than short-term cheating (Bronstein & Bshary, 2004).
In evolutionary terms, this long-term state is described as an Evolutionarily Stable Strategy (ESS). Once established in a population, ESS is a strategy that cannot be replaced with any alternative because it provides equal or greater fitness to organisms using it (Maynard Smith & Price, 1973). In the oak-fungus relationship, mutual cooperation persists because individuals that maintain balanced exchange tend to achieve higher overall reproductive success than those that cheat (Fellbaum et al., 2006). Mechanisms such as partner choice and sanctioning reinforce this stability: oaks direct more carbon to cooperative fungi that supply phosphorus or nitrogen efficiently, while reducing allocation to exploitative partners (Werner & Kiers, 2015). Over time, this feedback ensures that mutual investment remains as the ESS.
Optimization of Resource Exchange
This same principle leads to Kummel and Salant’s (2006) optimization model, where the oak distributes carbon among fungal partners until each provides nutrients at an equal return, representing the most efficient use of resources. In this model, each fungal partner, f, has an exchange function shown in Equation 8:

In this function, Nf represents the amount of nitrogen obtained from a given fungal partner, while rf(Nf) denotes the corresponding carbon cost required to “pay for” that nitrogen. The oak's goal is to minimize the total carbon it spends while still meeting its overall nitrogen requirement (NG) (Eq. 9); (Kummel & Salant, 2006):

Here, H(NG) represents the smallest total carbon cost possible for obtaining all the nitrogen the oak needs, considering the total number of fungal partners (F) that are symbiotically associated with the oak’s roots. This optimization has the constraint that the total nitrogen provided by all fungal partners (NG being nitrogen gained) must exactly equal the oak’s total nitrogen demand (Eq. 10); (Kummel & Salant, 2006):

At equilibrium, the oak distributes its carbon so that the marginal carbon cost (the extra carbon needed to gain one more unit of nitrogen) is equal across all fungal partners. Every extra bit of carbon the oak sends to any fungus provides the same benefit in return. This is shown in Equation 11:
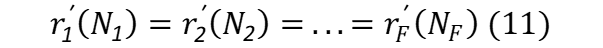
This condition means the oak is using its carbon as efficiently as possible. Each gram of carbon yields the same nutrient benefit no matter which fungus receives it, so the oak can’t improve its outcome by moving carbon from one fungus to another. This represents the ESS of the mycorrhizal system, showing a self-regulating network where both oak and fungi maximize long-term efficiency and stability (Kummel & Salant, 2006).
Network Models: EMF Linking Between Trees
Beyond the level of a single oak and its fungal partners, these same mathematical principles extend to entire forest networks. EMF form underground “webs” that link oaks, pines, and other species through shared nutrient pathways (Simard et al., 2012). Globally, these networks are one of the Earth’s largest carbon sinks, with an estimated 13 billion metric tons of CO₂ being cycled through mycorrhizal fungi each year (Hawkins et al., 2023).
This forest connectivity can be understood using network theory, where different trees act as nodes and fungal hyphae as the connecting edges. The image below (Fig. 11) illustrates four different ways connections such as these can be modeled mathematically: regular, random, small-world, and scale-free networks.

Fig. 11. Visual representations of random, small world, and scale-free networks, adapted from Selvarajoo, 2019. Created by J. Neufeld, 2025.
Regular networks have evenly spaced, uniform connections, and random networks connect nodes unpredictably. Small-world networks have many short-distance connections with a few long-distance links for fast communication, while scale-free networks feature a few highly connected “hubs” that make them efficient and resilient, like the fungal hubs linking trees in forest EMF systems (Selvarajoo, 2019). Among these network types shown above, evidence suggests that most mycorrhizal networks exhibit a scale-free network with small-world properties (Simard et al., 2012; Liu et al., 2021), meaning they contain a few highly connected fungal hubs and many locally clustered connections with short path lengths between trees (Simard et al., 2012). This structure allows resources to move efficiently across forests while maintaining stability if individual connections fail. [link to the maths of fungus, 2024]
In a scale-free network, the probability P(k) that a node (a tree or fungal hub) has k connections follows a power law (Eq. 12); (Barabási & Albert, 1999):

This shows that in a scale-free network, most nodes have only a few connections while a few hubs have many. This power-law form is characteristic of a Pareto distribution, where large values occur much less frequently than small ones, meaning nodes with many connections become rarer. In EMF systems, this explains why a few dominant fungal hubs connect many trees, maintaining efficient and stable nutrient flow across the forest (Simard et al., 2012; Liu et al., 2021). Preferential attachment emerges, with new roots or hyphae more likely to connect to already well-connected hubs. The result is a network that is self-organizing, efficient, and resistant to damage. If one link fails, others compensate through alternate pathways (Simard et al., 2012). Small-world properties add another layer of efficiency. Trees that are close to each other are connected through short paths, allowing carbon, nitrogen, and signaling molecules to move rapidly across the network (Simard et al., 2018). This combination of short path lengths and highly connected hubs minimizes energy costs while maximizing stability (Figueiredo et al., 2021). The persistence of the mutualistic relationship between oaks and mycorrhizal fungi shows how nutrient exchange between partners can create a mathematically stable, self-regulating system that plays a vital role in Earth’s ecosystems.
Conclusion
The oak tree demonstrates how mathematics can provide evidence for biological design solutions. Across every level of the oak’s structure, mathematical relationships validate how the oak’s form is optimized for efficiency and survival. The oak’s mechanism of growth follows mathematical logic that balances its height and strength. Growth models show that oaks adapt their rate of development to use energy wisely and maintain support, ensuring they can compete even in dense forests. At the structural level, the geometry of oak branches provides a design solution. By growing at wide angles, oaks capture more sunlight, but they also face greater bending stress. Torque and bending stress equations show how the tree compensates by thickening its branches and producing dense wood. This includes the formation of reaction wood, which develops in response to mechanical stress and helps the tree resist bending. The arrangements of the oak’s leaves and canopy further express mathematical order. Fractal vein networks and Fibonacci-based leaf configuration maximize nutrient transport and sunlight exposure. These patterns show that the oak’s structure is organized for efficiency, not random growth. Underground, the oak’s mutualism with ectomycorrhizal fungi operates as a mathematically stable system modeled by game theory, optimization equations, and network systems. This exchange allows both partners to gain essential nutrients while conserving energy. Together, these design solutions in the oak show that nature’s patterns are not random, but guided by mathematical order, where every pattern contributes to the strength and survival of the oak.
References
References
Al-Kadi, O. S. (2017). Fractals for biomedical texture analysis. Biomedical Texture Analysis, 131–161. https://doi.org/10.1016/b978-0-12-812133-7.00005-3
Archetti, M., & Scheuring, I. (2003). Mutualism or cooperation among competitors promotes coexistence and competitive ability. Ecological Modelling, 163(1–2), 17–23. https://doi.org/10.1016/S0304-3800(03)00069-3
Archetti, M., Scheuring, I., Hoffman, M., Frederickson, M. E., Pierce, N. E., & Yu, D. W. (2011). Economic game theory for mutualism and cooperation. Ecology Letters, 14(12), 1300–1312. https://doi.org/10.1111/j.1461-0248.2011.01697.x
Arseniou, G., & MacFarlane, D. W. (2021). Fractal dimension of tree crowns explains species functional‐trait responses to urban environments at different scales. Ecological Applications, 31(4). https://doi.org/10.1002/eap.2297
Barabási, A.-L., & Albert, R. (1999). Emergence of scaling in random networks. Science, 286(5439), 509–512. https://doi.org/10.1126/science.286.5439.509
Bayirli, M., Selvi, S., & Cakilcioglu, U. (2015). Determining different plant leaves’ fractal dimensions: A new approach to taxonomical study of plants. Bangladesh Journal of Botany, 43(3), 267–275. https://doi.org/10.3329/bjb.v43i3.21593
Binkley, D., Campoe, O. C., Gspaltl, M., & Forrester, D. I. (2013). Light absorption and use efficiency in forests: Why patterns differ for trees and stands. Forest Ecology and Management, 288, 5–13. https://doi.org/10.1016/j.foreco.2011.11.002
Brain, M. (2024, September 5). How evolution works. HowStuffWorks Science. https://science.howstuffworks.com/life/evolution/evolution.htm
Brack, C. (n.d.). Stands. The Australian National University. https://fennerschool-associated.anu.edu.au/mensuration/stand.htm
Bronstein, J. L., & Bshary, R. (2004). Game structures in mutualistic interactions: What can the evidence tell us about the kind of models we need? Santa Fe Institute Working Paper. https://wiki.santafe.edu/images/3/38/Game_Structures_in_Mutualistic_Interactions.pdf
Burgess, S. C., & Pasini, D. (2004). Analysis of the structural efficiency of trees. Journal of Engineering Design, 15(2), 177–193. https://doi.org/10.1080/09544820410001658517
Clatterbuck, W.K. (2002). Growth of a 30-year cherrybark oak plantation 6 years after thinning. United States Department of Agriculture Forest Service. https://www.srs.fs.usda.gov/pubs/gtr/gtr_srs048/article/gtr_srs048-clatterbuck01.pdf
Conge, H. (n.d.). Oak leaf, close-up. Science Photo Library. Retrieved November 9, 2025, from https://www.sciencephoto.com/media/135046/view/oak-leaf-close-up.
Dixit, A. K., Skeath, S., & Reiley, D. H. (2015). Games of strategy (4th ed.). W. W. Norton & Company. https://studylib.net/doc/25823956/games-of-strategy-4th-fourth-edition-
DeYoung, J., & Sutton, A. (2016). Forest measurements: An applied approach. Open Oregon Educational Resources. November 22, 2025, https://openoregon.pressbooks.pub/forestmeasurements/
Fellbaum, C. R., Mensah, J. A., Cloos, A. J., & Pfeffer, P. E. (2006). Mutualistic stability in the arbuscular mycorrhizal symbiosis: Exploring hypotheses of evolutionary cooperation. Ecology, 87(11), 2473–2480. https://pubmed.ncbi.nlm.nih.gov/16922314/
Figueiredo, A. F., Boy, J., & Guggenberger, G. (2021). Common mycorrhizae network: A review of the theories and mechanisms behind underground interactions. Frontiers in Fungal Biology, 2, 735299. https://doi.org/10.3389/ffunb.2021.735299
Galilei, G. (1957). The Assayer (p. 171). S. Drake Abridged and Trans., Stanford University. (Original work published 1623) https://web.stanford.edu/~jsabol/certainty/readings/Galileo-Assayer.pdf
Günay, E., & Sönmez, M. (2003). Mechanical Behavior of Wood under Torsional and Tensile Loadings. G. U. Journal of Science, 16(4), 733-749. https://www.researchgate.net/publication/228683427_Mechanical_Behavior_of_Wood_under_Torsional_and_Tensile_Loadings
Hawkins, H.-J., Cargill, R. I. M., Van Nuland, M. E., Hagen, S. C., Field, K. J., Sheldrake, M., Soudzilovskaia, N. A., & Kiers, E. T. (2023). Mycorrhizal mycelium as a global carbon pool. Current Biology, 33(11), 560–573. https://doi.org/10.1016/j.cub.2023.02.027
Hernandez, J. O., & Park, B. B. (2022). The leaf trichome, venation, and mesophyll structural traits play important roles in the physiological responses of oak seedlings to water-deficit stress. International Journal of Molecular Sciences, 23(15), 8640. https://doi.org/10.3390/ijms23158640
Hilt, D. E., & Dale, M. E. (1982). Height prediction equations for even-aged upland oak stands. United States Department of Agriculture Forest Service. https://doi.org/10.2737/ne-rp-493
Hodžić, M. M., & Ballian, D. (2020). Quality of pedunculate oak provenances in Bosnian-herzegovinian provenance test based on branching angle and stem form. Forestist, 70(2), 95–104. https://doi.org/10.5152/forestist.2020.20008
Jiménez-Guzmán, G., & Vega-Peña, E. V. (2024). Temporal Dynamics of Tree Crown Fractal Dimension in Two Species of Deciduous Oaks. The Botanical Review, 90, 109-129. https://doi.org/10.1007/s12229-023-09298-6
Keeler, H. L. (2005). Our native trees and how to identify them: A popular study of their habits and their peculiarities. Kent State University Press.
Kremer, A., & Hipp, A. L. (2019). Oaks: An evolutionary success story. New Phytologist, 226(4), 987-1011. https://doi.org/10.1111/nph.16274
Kuhlemeier, C. (2007). Phyllotaxis. Trends in Plant Science, 12(4), 143–150. https://doi.org/10.1016/j.tplants.2007.03.004
Kümmel, T., & Salant, S. W. (2006). The economics of mutualisms: Optimal utilization of mycorrhizal mutualistic partners by plants. University of Michigan, Department of Economics. https://escholarship.org/content/qt14b5d950/qt14b5d950_noSplash_7e898dd7e9c06edd8b5ac21041510ca8.pdf
Martin, F. M., & van der Heijden, M. G. A. (2024). The mycorrhizal symbiosis: Research frontiers in genomics, ecology, and agricultural application. New Phytologist. https://doi.org/10.1111/nph.19541
Maynard Smith, J., & Price, G. R. (1973). The logic of animal conflict. Nature, 246(5427), 15–18. https://doi.org/10.1038/246015a0
McCreary, D. D. (1991). Seasonal growth patterns of blue and valley oak seedlings established on Foothill Rangelands. United States Department of Agriculture Forest Service. https://research.fs.usda.gov/treesearch/28396#:~:text=Abstract,suitable%20environmental%20conditions%20are%20maintained
Mediavilla, S., & Escudero, A. (2023). Branch architecture in relation to canopy positions in three Mediterranean Oaks. Oecologia, 201, 915–927. https://doi.org/10.1007/s00442-023-05358-1
https://doi.org/https://doi.org/10.1199/tab.0108
National Wildlife Federation. (n.d.). Southern Live Oak. https://www.nwf.org/Educational-Resources/Wildlife-Guide/Plants-and-Fungi/Southern-Live-Oak
Ng, M., Lau, R., Tsang, L., & Wells, R. (2002). Fractal dimension of leaves. The Physics Factbook. https://hypertextbook.com/facts/2002/leaves.shtml
Okabe, T. (2015). Biophysical optimality of the Golden Angle in Phyllotaxis. Scientific Reports, 5(1). https://doi.org/10.1038/srep15358
Okabe, T. (2024). Evolutionary origins of fibonacci phyllotaxis in land plants. Heliyon, 10(6). https://doi.org/10.1016/j.heliyon.2024.e27812
Okabe, T., Ishida, A., & Yoshimura, J. (2019). The unified rule of Phyllotaxis explaining both Spiral and non-spiral arrangements. Journal of The Royal Society Interface, 16(151), 20180850. https://doi.org/10.1098/rsif.2018.0850
Price, C. A., Knox, S.-J. C., & Brodribb, T. J. (2013). The influence of branch order on Optimal Leaf Vein geometries: Murray’s law and area preserving branching. PLoS ONE, 8(12). https://doi.org/10.1371/journal.pone.0085420
Prusinkiewicz, P., & Hanan, J. (1989). Lindenmayer Systems, Fractals, and Plants. Springer-Verlag.
Prusinkiewicz, P., & Lindenmayer, A. (1990). The Algorithmic Beauty of Plants. Springer-Verlag.
Selvarajoo, K. (2019, September 12). Large scale-free network organization is likely key for biofilm phase transition [Review]. Engineering Biology, 3(4), 67–71. https://doi.org/10.1049/enb.2019.001
Shifley, S. R. (2004). Oak growth and response to thinning. United States Department of Agriculture Forest Service. https://research.fs.usda.gov/treesearch/6542
Simard, S. W., Beiler, K. J., Bingham, M. A., Deslippe, J. R., Philip, L. J., & Teste, F. P. (2012). Mycorrhizal networks: Mechanisms, ecology and modelling. Fungal Biology Reviews, 26(1), 39–60. https://doi.org/10.1016/j.fbr.2012.01.001
Simard, S. W., Perry, D. A., Jones, M. D., Myrold, D. D., Durall, D. M., & Molina, R. (1997). Net transfer of carbon between ectomycorrhizal tree species in the field. Nature, 388(6642), 579–582. https://doi.org/10.1038/41557
Sternberg, G. (n.d.). Pruning oaks: Training the young to achieve grandeur Guy Sternberg. International Oak Society. https://www.internationaloaksociety.org/sites/default/files/files/document/19-ios-journal-24-sternberg-sm.pdf
Stewardship and Outreach Section Department of Natural Resources. (n.d.). A brief introduction to thinning for value. https://novascotia.ca/natr/Education/woodlot/shortversion/Thinning%20For%20Value.pdf
Taylor, B. (n.d.). Angel Oak. Charleston SC. https://www.charleston-sc.gov/153/Angel-Oak
Werner, G. D. A., & Kiers, E. T. (2015). Partner selection in the mycorrhizal mutualism. New Phytologist, 205(4), 1437–1442. https://doi.org/10.1111/nph.13113
Wolfe, B. E., & Tylianakis, J. M. (2021). When does mutualism offer a competitive advantage? A game-theoretic analysis of host–host competition in mutualism. bioRxiv. https://doi.org/10.1101/2021.07.13.452216