
Table of Contents
Keywords: Fractal, game theory, fir tree, abies, roots, evolutionary stable strategy, tragedy of the commons
Abstract
This paper analyzes the optimizations, strategies, and patterns present in fir trees from a mathematical perspective. Firs optimize height and leaf area with age in ways converse to the common trend in trees. The leaf-to-trunk area increases with height, which could benefit nutrient storage in harsh environments, outcompete nearby plants, and control soil pH. Next, the interactions among fir trees are analyzed using game theory to examine tree growth, seeding strategies, and root competition. The relationship between height and stem diameter is summarized in a strategy matrix, where the traits interact synergistically to optimize tree growth. The many possible benefits behind periodic mast seeding events found in firs are evaluated to determine why plants would choose a reproductive strategy that seems inefficient. Root proliferation in an area is dependent on abiotic and biotic factors, including the influence of other plants. Using game theory, it is found that plants must engage in a race to deplete soil nutrients or risk losing to competition. Finally, the fractal patterns found in the first, above- and below-ground, are introduced. Both the roots and branches of the fir are fractals, with highly regular, self-similar layouts that have several benefits. In roots, fractals aid nutrient absorption and plant stability. In branches, fractals span 3D space, providing available photosynthetic surfaces and mitigating snow buildup. The recursive algorithms behind fractals are explored, revealing the profound relationship between plants and math.
Introduction
As seen in the two previous papers, “Wonders of Forest Giants: Physical Properties Governing Fir Trees” and “Chemistry in Action: How Chemistry Facilitates the Survival of the Fir Tree”, the fir tree is a versatile tree that has evolved to have design solutions rooted in physics and chemistry. Mathematics is no different, with the fir tree solving overcoming adversity with mathematical concepts. This results in the fir tree existing in a highly predictable manner, with many of its characteristics represented by mathematical models. Mathematics shows that the fir tree opposes the general trend of a negative relationship between height and leaf area, with leaf area increasing with greater height. Additionally, the relationship between diameter and stem height can be represented in a game-theoretic matrix. The fir’s roots exhibit a similar interplay to the height and diameter, both within the same tree and with roots from different organisms. Depending on the situation, the game-theoretic matrix for root behaviour will predict a different outcome for the tree alone or for the tree and another organism. By this, the way the fir tree propagates its roots depends on the behaviour of other organisms around it, resulting in different root propagation behaviour. Game theory also comes into play in how the fir tree decides to optimize the spread of its seeds to maximize the chance that an offspring will take root. Furthermore, fractals govern the above and below-ground appearance of the tree. Fractals can be observed in the roots, whereby the structure and propagation of the roots grow in a manner that is almost predictable without the influence of outside organisms. The same is true regarding the growth of primary, secondary, tertiary, etc., types of branches. Whereby their growth results in the ionic conical shape of the fir. Throughout this paper, these topics will be further explored. The mathematical design solutions the fir tree has developed will also be presented to round out the marvellous way in which it has developed design solutions across three distinct but interconnected domains to sustain its iconic longevity.
Relationship between the Height of a Tree and its Leaf Area
In most tree species, the leaf area to sapwood area ratio decreases as the tree becomes older and taller. The leaf area to sapwood area ratio is described by formula 1:

Where D is the atmospheric vapour pressure deficit, gs is canopy conductance to water vapour, ks is sapwood permeability of the hydraulic pathway, ΔΨ is the soil-to-leaf water potential difference including the effect of gravity, η is the viscosity of water at a given temperature, and h is the tree height. It is important to note that this formula has several limitations when applied to a tree; these limitations are further explored in the 2002 paper by McDowell et al. The current hypothesis for this is that the leaf area to sapwood area ratio must decrease to maintain leaf-specific hydraulic sufficiency since, as the tree grows taller, the path length increases, and gravity has a larger effect on the tree’s hydraulic conductance (McDowell et al., 2002). Thus, to sustain leaves growing at progressively greater heights, the tree must decrease the total number of leaves to provide the nutrients they need to survive. Otherwise, certain leaves would not receive sufficient nutrients, becoming weakened. Additionally, in Equation 1, if we assume all other variables are constant, then as h increases, the ratio decreases, providing a mathematical basis for the current hypotheses. As stated, this is generally true in most trees; however, in two studied species, Picea abies (Norway spruce) and Abies balsamea (balsam fir), it is not true. In fact, these trees showed an increase in the leaf area-to-sapwood area ratio with increasing height. This is evident in Table 1, which presents data from McDowell et al. (2002).
Table 1: Raw slope extracted from the regression function of different Pinus and Abies species.
| Species | n | Height (m) | Al:As | Raw slope |
|---|---|---|---|---|
| Pinus sylvertris | 14 | 5-25 | 0.19 | -0.008 |
| Pinus monticola | 21 | 4-44 | 0.22 | -0.004 |
| Picea abies | 28 | 7-31 | 0.36 | +0.017 |
| Abies balsamea | 50 | n/a | 0.71 | +0.031 |
In the table, the raw slope is a representation of the slope obtained by doing a regression of Al:As as a function of the tree’s height. In this, we see that both fir species have positive slopes, which is unusual. Given that the two studied fir tree species exhibited a positive regression slope, there must be a reason why fir trees deviate from the general trend of all other major tree species. As seen in “Wonders of Forest Giants: Physical Properties Governing Fir Trees”, fir trees grow primarily in cold, nutrient-poor mountainous regions. Thus, by retaining a larger canopy, it has been theorized that more nutrients can be stored higher up in the tree, facilitating easier redistribution in this area. During periods when nutrient transport is more difficult, such as during cold winter months, a larger canopy allows fir trees to maintain a nutrient store in the foliage, which can be redistributed in the canopy rather than attempting to bring nutrients all the way up the tree. Additionally, by retaining a larger upper canopy, the tree's height increases the area of shade it casts. This reduces light for lower-growing vegetation, allowing the tree to access more nutrients in the surrounding soil and permitting it to grow more (McDowell et al., 2002). Another possible theory for this relates to information presented in "Chemistry in Action: How Chemistry Facilitates the Survival of the Fir Tree", which shows that fallen fir needles change the pH of the soil surrounding the tree, allowing fungi to grow and decompose nutrients. If fir trees have plenty of fir needles as they grow taller, the area on which the needles will fall will also increase. This necessitates a larger total number of needles to maintain the same needle-to-square-meter ratio as in a shorter tree, thereby providing the correct pH change in the soil. This provides more space for fungi to inhabit and thus break down nutrients for the fir tree.
Fir Tree and Game Theory
Game Theory of Stem Allometry
The allometric relationship, which describes how a functional trait changes in proportion to body size, between stem height and diameter, reflects an interesting trade-off in a tree's strategy to secure carbon storage during vegetative growth and ensures gene transmission into future generations via reproductive growth (Fu et al., 2017). The best way to observe this trade-off is in a system with two components, height and diameter, where they interact and coordinate in a way that is reliant on endogenous and exogenous factors. To quantify the relationship between stem height and diameter growth, we can use Lotka-Volterra differential equations in which one species acts as a predator and the other as prey. Additionally, given that growth follows a logistic curve composed of exponential, linear, and asymptotic growth, we can incorporate this into the Lotka-Volterra equations to better describe the relationship. In the following relationship (Eq. 2 and Eq. 3), H is the height, D is the diameter of growth at age t, αH and αD represents the independent growth rates, KH and KD represent the maximum growth values, and rH and rD are the velocities of a trait to grow to its maximum value. Additionally, the dependent growth is determined by the phenotype of interactions; this dependence is described by the interaction HD and DH parameters and the scale parameters SH←D and SD←H (Fu et al., 2017).

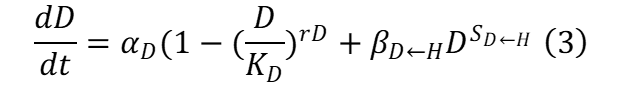
These relationships can be broken down into two different components. The first part is the representation of the tree’s independent growth that takes place by assuming that the target trait is in an isolated condition:


The second part is the representation that the tree’s dependent growth arises from the interaction of the target trait with its co-existing trait through a certain mechanism:


The sign and magnitude of the dependent growth determine the type of interaction observed between height and diameter. The various outcomes can be visualized in the following strategy matrix shown in Table 2.
Table 2: Game matrix showing the possible outcomes depending on the behaviour of dDb/dt and dHb/dt.
dDb / dt | |||||
dHb / dt | + | 0 | - | ||
| + | + | +/+ (mutualism) | +/0 (commensalism) | +/- (predation) | |
| 0 | 0 | 0/+ (commensalism) | 0/0 (synergism) | 0/- (amensalism) | |
| - | - | -/+ (predation) | -/0 (amensalism) | -/- (competition) | |
As shown in the strategy matrix, the outcome depends on the stance adopted. The various strategies used will result in six unique types of ecological interactions:
Mutualism: the two traits benefit from one another.
Synergism: no dramatic mutual benefit for both traits.
Competition: negative interactions between the two traits that may use the same limited pool of resources.
Commensalism: one trait benefits from another without affecting itself.
Predation: one trait benefits at the cost of the other.
Amensalism: one trait harms the other, despite providing no benefit to the former (Fu et al., 2017).
From this, we can understand how the changes in height and diameter are related. Given that they are related through a specific mechanism, there will be varying outcomes, as observed in the strategy matrix. For the fir tree, this poses an interesting dilemma, as seen in Wonders of Forest Giants: Physical Properties Governing Fir Trees, where diameter and height are positively correlated due to structural constraints. Consequently, the fir must ensure it can sustain a positive correlation between the two without violating the chosen relationship, as outlined in the strategy matrix. Thus, it is reasonable to believe that the height and diameter of the fir tree work in either a mutualism or a synergism manner, resulting in the best possible outcome for the tree’s growth.
Game Theory of Mast Seeding
Mast seeding is a phenomenon in which long-lived plants produce many seeds in some years and very few in intervening years. The mast seeding years are characterized as periodic, synchronous within a population, and highly variable in the number of seeds produced between mast and non-mast years. A study found that Abies balsamea met the criteria for highly variable seed production, and although the study's seven-year duration is too short to determine whether the production is periodic, it is fair to say that firs exhibit mast-seeding behaviour (Houle, 1999). It is also fair to question why the trees would develop this behaviour at all, since it comes with the cost of delayed reproduction. The fundamental question is whether there is a benefit to mast seeding over consistent reproductive production, or whether a factor limits production in certain years (Pearse et al., 2016). In fact, it may be a combination of many factors that leads to mast seeding, as seen in Table 3.
Table 3: Effects of hypotheses for mast seeding. Adapted from (Pearse et al., 2016).
| Hypothesis | Economy of scale? | Synchronous? | Variability? |
|---|---|---|---|
| Resource budget model | No | No | Yes |
| Predator satiation | Yes | No | No |
| Pollination efficiency | Yes | Yes | No, but could cause crops to fail some years |
| Weather cues | No | Yes | Yes, depending on cue and plant sensitivity |
Economy of scale (EOS) is the reduction in per-unit production cost resulting from increased output. A hypothesis for mast seeding behaviour must explain both the synchronous and variable characteristics of the phenomenon as well as provide the deeper evolutionary benefit – in other words, it must explain why seeding is an EOS (Pearse et al., 2016).
The resource budget model is widely used to analyze mast seeding in plants (Isagi et al., 1997). According to the model, the plant produces a quantity of stored organic molecules, known as photosynthate (Ps). When Ps reaches a certain threshold LT, Ps is reduced to LT - Ca , where Ca is the cost of fruiting. This model produces the periodicity and high variability of mast seeding (Isagi et al., 1997). However, the model alone doesn’t explain why populations synchronize mast seeding years or the EOS (Pearse et al., 2016).
Some alternative hypotheses are provided in Table 2. A plant may produce more seeds to satiate predators, allowing more seeds to escape predation (Isagi et al., 1997). This explains the EOS but not the year-to-year variability. There are higher cross-pollination ratios in years with high flowering, leading to EOS and synchrony, but not high variability. Certain weather cues, such as rainfall, temperature, and fire, would affect all members of a population similarly and may increase or decrease seed production. For example, it is beneficial to seed directly after a fire due to the low competition and nutrient-rich soil (Pearse et al., 2016).
In fir trees, high seed production was positively correlated with pollination efficiency and with dry conditions at the time of reproductive bud initiation (Houle, 1999). The trees didn’t have successive years of high seed production, which supports the resource budget model. The complex factors behind mast seeding are still being investigated, but the success of fir trees and the many other mast-seeding plants shows that nature finds unexpected benefits in seemingly disadvantageous strategies.
Game Theory in Roots
The amount of root proliferation per unit volume of soil, or root density, in plants is highly phenotypically flexible (Cabal, 2022). For a solitary plant, the basic model of its proliferation is an exploitative strategy, in which the plant maximizes nutrient uptake at the cost of growing new roots. It is beneficial to increase root density in an area up until a certain point. After this point, the benefit of each additional root decreases as roots begin competing for the same resources (Gersani et al. 2001). Additionally, root growth efficiency decreases with distance because resources must be transported farther from the plant (Cabal, 2022). The balance between these factors is important for solitary plant growth but becomes much more complicated when multiple plants are in close proximity.
The basic model of a plant can sense and respond to abiotic soil factors, including the nutrients it absorbs (Cabal, 2022). A sophisticated plant, as seen experimentally, is also able to recognize the presence of other plants. When multiple plants share a space, the best strategy for all involved is ideal free distribution (IFD). Following this strategy, the root density of plants would remain the same for solitary and sharing plants, assuming the resources per plant are constant. However, a different strategy is expected for both exploitative and sophisticated plant models and is supported by experimental data. This strategy is called the root tragedy of the commons (RTC) (Cabal, 2022).
The root tragedy of the commons is a situation in which individuals fully exploit a community resource for individual gain, leading to its depletion and collective loss. The RTC is considered an evolutionary stable strategy, meaning it cannot be displaced by another strategy without changes in the environment (Gersani et al., 2001). The strategy is resilient, even though individuals in an IFD community have a higher reproductive yield, because the depletion is borne by the community. At the same time, any gain comes from individual root proliferation. If one individual in a community were not to increase root density from the solitary to the shared condition, it would endure the same depletion in nutrients without any compensation through proliferation. Conversely, if a community were not to increase root density but an individual did, the individual would absorb the most nutrients and have the highest reproductive yield (Gersani et al., 2001). The RTC is the dominant strategy not because it is the best, but because it is so unfavourable not to follow.
The Fractal Nature of Abies Trees
Fractals can be snowflakes, coastlines, or branching systems such as trees and blood vessels. What do all these have in common? They are patterns that repeat themselves at different scales. Small parts of a fractal are similar to the entire pattern itself. Nature shows self-similarity at all scales, and no matter how closely you zoom into a fractal, you will find similar patterns recurring—a property called scale invariance. Fractals observed in nature will often exhibit non-integer fractal dimensions in the range between two and three.
Fractality Above Ground
Like most trees, the fir exhibits a degree of self-similarity. A branch can be viewed as a smaller version of the whole. This fractal nature is not merely an aesthetic observation but rather a design solution for competing needs. Each branch increases the effective area for photosynthesis, capturing light over a larger volume while limiting self-shading. Phloem and xylem are effectively transported in the fir’s fractal networks. Recursive branching distributes loads evenly. Bending stress is applied across sub-branches, which carry progressively smaller loads as fractal interactions increase. Fractal branching creates a very efficient internal network for the transportation of water and nutrients. The trunk and the main branches of the tree carry bulk flow, which splits into many twigs and vascular passages that deliver sap to the needles. The near-constant cross-sectional area across the branch levels helps maintain steady fluid pressure and minimizes flow resistance. The volume-to-area relationship in branching ensures that all leaves can be fed, regardless of their distance from the trunk, without the tree needing thick, heavy branches. (Ball, 2009)
The fractal argument starts with a trunk; segments then grow and split at species-specific angles, and length and thickness scale down by a constant factor until the point where energy or cellular size limits halt division. This is the point where needles form.
The recursive relationship benefits the tree as each segment is a smaller copy of the whole. The angle at which the branches spawn is fixed, but the length and diameter shrink at a near constant step with each fractal iteration. Each branching moment creates a fractal where the two daughter branches. Due to the fractal architecture, the fir's scaling follows a power law. Dating back to Leonardo da Vinci’s observations, the total thickness of branches after a split is equal to the parent branch. This can be represented by Equation 8:

Variable r represents the branch radius. The claim can be made that the cross-sectional area is roughly conserved following splitting (Gao & Newberry, 2025). This relationship is illustrated in Figure 2.
Figure 1 shows two trees that, at a mathematical level, ideally obey tree fractality. It can be observed that branching overlap occurs in the dimensionality range from one to two. In real tree environments, the radius is not perfectly conserved from mother to daughter branch, and the branching angle has variance. Nonetheless, the models can be used to visualize how real trees are quasi-fractal. Mode A is reflected along the vertical axis, whereas mode B does not contain vertical symmetry.

Fig. 1. (1,2)-dimensional ‘tree’ fractals generated to represent the idea of a tree being a fractal (Noah Deniaud). Images were generated in the Mathematica environment.

Fig. 2. Conservation of tree thickness as observed by Leonardo da Vinci circa 1500 (Gao & Newberry, 2025).
The resultant spire shape of the fir is not a mere accident but rather an adaptation to survive harsh winter weather. A fir tree’s frost resistance can be attributed to the fractal nature of the fir. Lower branches are sturdier, while upper ones are shorter, forming a natural cone that sheds snow efficiently. As snow accumulates, the flexible side branches of fir sag under the weight until they effectively interlock with the branch layer below, creating a continuous slope that allows the snow to slide off easily (Shea 2021). Heavy snow buildup is therefore mitigated. The conical shape of a fir tree minimizes light occlusion among branches and maximizes sunlight exposure (for photosynthesis). This can be modelled mathematically as a solid of revolution with height h and base radius r. The volume-to-surface-area ratio, V/A, is optimized in Equation 9 as:

Fractality of Roots
One rather beautiful aspect of fir trees is the nature of their root systems, seeing as they grow immensely in networks through the soil. This root system is not random, however; it is dictated by the fractality of the roots, as with many other soil-growing plants. Root fractality entails that the tree branches in self-similar fractal patterns, and it offers many benefits for the tree’s survival (Berntson et al., 1998)
The fractal nature of these roots is indicated by their fractal dimension, a numerical measure of their complexity and space-filling. The fractal dimension is given by Equation 10 below (Larsson, 2018).

The basis of this equation is that it looks at a given space in terms of boxes or grids (N) and determines how many boxes are needed to fill a space of repeated fractal structures. These boxes are of length ℓ, which provides a scale for the box size as the fractal structure gets smaller. The formula follows a logarithmic-ratio form, namely the ratio of the logarithm of N to the logarithm of 1/ℓ. As one zooms in on the structure’s roots (i.e., as r decreases), the number of boxes that cover the observed space increases exponentially. This means that the box length scales exponentially (Figure 3).

Fig. 3. Image depicting the exponential growth of fractal dimension in terms of boxes (Vanderbilt University, 2019).
Converting this exponential relationship to a logarithmic ratio yields a slope, Df, that indicates the amount of space the structure occupies (Equation 10). For the fir tree’s roots, a higher value of Df indicates that as the scale r is decreased, there are more fractal roots present in a complex, branched network. Inversely, a low Df value would imply that at a smaller level, there is less branching and that the growth pattern is less fractal. For instance, if the value of Df is closer to 1, this indicates a simple root system that essentially resembles a line. However, in 3D biological structures like roots, Df can range from 1 to 3. The Df range of 1-2 indicates a higher level of branching, though more resembling a planar structure. A Df value between 2 and 3 indicates a very branched fractal root system that covers a wide space rather than just a single plane (Fitter & Stickland, 1992). Given the very fractal nature of fir roots, fir tree roots would tend to reflect a Df value slightly above 2 in the range of 2.1-2.3, depending on the specific tree.
The fir tree utilizes this root fractality to its advantage, one such way being that it allows for an increase in the tree’s nutrient absorption. Given this scaled growth pattern of the roots to such a small degree, having these incredibly small root extensions increases the surface area upon which the nutrients are absorbed under the tree. With every additional fractal root in smaller degrees, not only can more of the soil be explored, but having these minuscule extensions allows for more absorption compared to the large primary roots (Dupuy et al., 2010). Fir trees also use the fractality of their roots to their advantage in competition with surrounding trees. As seen in Figure 4, having these fractal root branches under the tree allows the tree to secure the soil beneath it and to compete less with neighbouring trees for nutrients, leaving fewer soil spaces unused. (Dupuy et al., 2010).

Fig. 4. Image depicting fractal tree roots, highlighting the extensive root network for optimal absorption and the defence posed against competition from surrounding trees (Eytan Zlotorynski, 2020).
Finally, having these roots grow in a fractal pattern provides greater stability for the tree, as the large network of similarly branched roots acts as an anchor. As the overall root surface area increases with a higher fractal dimension, it becomes much more difficult for external forces like wind to uproot the tree, given the resistance posed by friction. Having these roots grow at increasingly smaller scales allows the stress from such external factors to be evenly distributed across the root system.
Conclusion
It has been said that math is the language of the universe, and it can certainly be seen in the characteristics of fir trees. Not only does math dictate so many of the tree’s qualities, but these specific compositions of the fir provide many survival advantages. As first noted, fir trees differ from many other species in that their leaf area-to-sapwood ratio increases with height. This growth is formulaic based on variables including tree height, sap permeability, and vapour pressure deficit. This increased ratio is an effective design, given that the large canopy helps store nutrients and shades light from competitive plants. Moreover, the tree’s dynamics between stem height and diameter is modelled by the Lotka-Volterra equations. Given this recognizable pattern, these two traits of the tree result in various combinations that offer mutualistic and synergistic relationships that benefit the tree. The tree also exhibits periodic mast seeding, which entails large seed production followed by low production years. This seeding follows a periodic-threshold model, offering higher long-term pollination success. Furthermore, it was discussed that the root structure of fir trees follows a fractal pattern, which can be quantified using fractal dimension. These fractal roots offer several design advantages, including increased nutrient absorption, reduced competition with neighbouring trees, and improved stability. Finally, the rest of the fir tree also exhibits fractality, primarily in the branching of its trunk and canopy. This branching is represented algebraically; for instance, the branch thickness relates to the split and parent branches. These fractal branching forms serve as a mathematical design solution, enabling efficient transport networks, load distribution, and other benefits. Given all of the qualities, it is evident that the fir tree’s mathematical structure solves many of its most important challenges.
References
References
Ball, P. (2009). Branches (pp. 96–103). OUP Oxford.
Berntson, G. M., Lynch, J., & Snapp, S. (1998). Fractal Geometry and the Description of Plant Root Systems: Current Perspectives and Future Applications (1st ed.). CRC Press.
Cabal, C. (2022). Root tragedy of the commons: Revisiting the mechanisms of a misunderstood theory. Frontiers in Plant Science, 13, 960942–960942. https://doi.org/10.3389/fpls.2022.960942
Dupuy, L., Gregory, P. J., & Bengough, A. G. (2010). Root growth models: towards a new generation of continuous approaches. Journal of Experimental Botany, 61(8), 2131–2143. https://doi.org/10.1093/jxb/erp389
Eytan Zlotorynski. (2020). The secret of increased (root) hair density. Nature Reviews Molecular Cell Biology, 21(11), 657–657. https://doi.org/10.1038/s41580-020-00302-0
Fu, L., Sun, L., Hao, H., Jiang, L., Zhu, S., Ye, M., Tang, S., Huang, M., & Wu, R. (2017). How trees allocate carbon for optimal growth: insight from a game-theoretic model. Briefings in Bioinformatics, 19(4), 593–602. https://doi.org/10.1093/bib/bbx003
Gersani, M., Brown, J. s., O’Brien, E. E., Maina, G. M., & Abramsky, Z. (2001). Tragedy of the commons as a result of root competition. Journal of Ecology, 89(4), 660–669. https://doi.org/10.1046/j.0022-0477.2001.00609.x
Houle, G. (1999). Mast seeding in Abies balsamea, Acer saccharum, and Betula alleghaniensis in an old-growth, cold-temperate forest of north‐eastern North America. Journal of Ecology, 87(3), 413–422. https://doi.org/10.1046/j.1365-2745.1999.00352.x
Isagi, Y., Sugimura, K., Sumida, A., & Ito, H. (1997). How Does Masting Happen and Synchronize? Journal of Theoretical Biology, 187(2), 231–239. https://doi.org/10.1006/jtbi.1997.0442
McDowell, N., Barnard, H., Bond, B., Hinckley, T., Hubbard, R., Ishii, H., Köstner, B., Magnani, F., Marshall, J., Meinzer, F., Phillips, N., Ryan, M., & Whitehead, D. (2002). The relationship between tree height and leaf area: sapwood area ratio. Oecologia, 132(1), 12–20. https://doi.org/10.1007/s00442-002-0904-x
Pearse, I. S., Koenig, W. D., & Kelly, D. (2016). Mechanisms of mast seeding: resources, weather, cues, and selection. New Phytologist, 212(3), 546–562. https://doi.org/10.1111/nph.14114
Gao, J., & Newberry, M. G. (2025). Scaling in branch thickness and the fractal aesthetic of trees. PubMed, 4(2), pgaf003–pgaf003. https://doi.org/10.1093/pnasnexus/pgaf003
Shea, S. (2021, June 12). Balsam Fir: A Favorite Christmas Tree. Northernwoodlands.org; The Center for Northern Woodlands Education. https://northernwoodlands.org/outside_story/article/balsam-fir-tree
Vanderbilt University. (2019). Fractals & the Fractal Dimension. Vanderbilt.edu. https://www.vanderbilt.edu/AnS/psychology/cogsci/chaos/workshop/Fractals.html