
Table of Contents
Keywords: Araucaria, Allometric Scaling, Structural Adaptation, Fractal Geometry, Photosynthetic Efficiency, Fibonacci Phyllotaxis, Grain Patterns, Tracheid Wall Thickness
Abstract
At the core of engineering, the foundational discipline of mathematics is an essential for the success of any project, and that is reflected even in nature. The Araucaria towers over the southern hemisphere by applying various mathematical principles in ingenious ways and this has guaranteed its continued success over millions of years.
Araucaria take advantage of allometric scaling growth patterns that prioritize structural stability, actively adjusting growth based on physical constraints in the environment
such as wind and efficient water transport. Going outside the familiar, they rely on fractal geometrical shapes at various levels to maximize their ability to photosynthesize within a crowded environment. From their leaves to their branches, Araucaria turns geometry into a means of light optimization, structural balance, hydraulic and reproductive efficiency. Even down to the level of their grain pattern, the Araucaria continue to demonstrate superior mathematical arrangements, minimizing wasted space using dense and uniform tracheid spacings which also contribute to greater trunk resilience.
Introduction
The growth morphology of Araucaria is not a result of biological chance but is meticulously orchestrated by mathematical order. The system of Araucaria follows the allometric scaling law, which ensures structural stability through the proportional relationship between height and diameter. Branching patterns form fractal geometric patterns that maximize light capture and material efficiency. Furthermore, the Fibonacci spiral arrangement optimizes the spatial arrangement of branches and leaves, achieving both photosynthesis and mechanical equilibrium. This mathematically repetitive structure suggests that Araucaria is not simply a product of biological adaptation but rather has evolved according to a geometric logic calculated by nature.
This geometric precision is consistent from the massive tree form to the microscopic cellular level. The arrangement and wall thickness of the tracheids follow an ideal geometric gradient to withstand the varying transport pressures and stress distributions with height. Its cellular structure simultaneously satisfies the three physical requirements of water flow, strength, and elasticity. The anisotropic grain structure of the wood distributes stress in multiple directions, minimizing crack propagation and maintaining structural elasticity under strong winds and vibrations.
Ultimately, these mathematical and structural adaptations demonstrate that Araucaria embodies the laws of physics in living form. They are not remnants of the past but are rather evolutionary computations where nature calculates and implements its own laws. Exploring the mathematics and dynamics hidden within Araucaria enables the opportunity to analyze the interaction between mathematics and nature.
Wind Influence on Allometric Scaling and Structural Adaptation in Araucaria
There are certain rates and rules for tree growth. The mathematical concept that describes these patterns is allometric scaling. Allometric scaling refers to the proportional change in the size of one part of an organism when the size of another part changes. In the case of trees, it examines how height (H) changes as trunk diameter (D) increases (West et al., 1999; Mäkelä, 2006). This relationship is usually expressed mathematically in Equation 1 where k is the proportionality constant that depends on species and b is the allometric exponent.
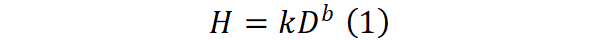
This formula succinctly and precisely captures a tree's morphological characteristics. When log-transformed, we get Equation 2 where the slope b and the y-intercept are log k (Niklas, 1995) (See Figure 1 for a graphical representation).


Fig. 1. Height–diameter log regression line for various tree species. The slope, b, represents the height–diameter growth rate (Niklas, 1995).
The allometric index b is a key variable that determines the morphological and structural characteristics of a tree. As b approaches 1, height and diameter increase at roughly the same rate, indicating balanced growth. When b is less than 1, the diameter increases more rapidly than the height, resulting in a short and thick tree. Conversely, when b is greater than 1, height increases more rapidly, resulting in a slender and tall tree. For most tree species, b values range from 0.5 to 0.9, reflecting physical constraints such as gravity, wind, and water transport efficiency (Thomas et al., 2015).
Trees of the genus Araucaria are a particularly intriguing example of heteromorphic growth relationships. They emerged approximately 200 million years ago during the Mesozoic Era and have maintained a largely unchanged form to this day, earning them the nickname "living fossils" of ancient conifers (Xie et al., 2024). They primarily grow in environments with high mechanical stress, such as windswept coastal cliffs or high mountain regions. According to Equation 1, the measured b value of Araucaria was reported to be approximately 0.5 to 0.7, and the k value was reported to be approximately 15 to 25 (Thomas et al., 2015; Xie et al., 2024). In other words, as the diameter increases, height increases gradually, exhibiting a growth pattern that prioritizes structural stability (Figure 2).

Fig. 2. Relationship between tree height (H) and diameter at breast height (DBH) for living Araucaria trees. Observed data (grey circles) and fitted allometric models (solid and dashed lines) show a nonlinear relationship following Equation 1, where b < 1 indicates height increases more slowly than diameter as trees grow (Xie et al., 2024).
This is a much slower rate than that of typical broadleaf trees (b ≈ 0.9). Mathematically, when b < 1, this is a phenomenon called sublinear scaling, where the tree's height increases at a rate equal to or more slowly than the square root of its diameter. Therefore, even if the total volume increases, the center of mass does not rise dramatically (Enquist et al., 2009). This structural advantage reduces the moment of force (See Equation 3) under high wind loads, minimizing the risk of tipping (Xu et al., 2023).

Here, b is not a simple statistical indicator but can be interpreted as a geometric ratio that determines the tree's morphological design. If the tree is simplified to a conical structure, its volume is approximated as seen in Equation 4:

And by substituting with Equation 1, we get Equation 5 which shows the rate of biomass growth expressed as a function of diameter growth.

In other words, a lower value of b allows for more efficient maintenance of volume (or biomass) for the same diameter increase, reducing structural burden. This is also related to the efficiency of energy distribution. Furthermore, the mechanical stability of wood is proportional to the second moment of area (See Equation 6).

Considering the bending stress due to wind load (See Equation 7), where σ is the bending stress, M is the bending moment, y is the perpendicular distance from the neutral (zero-stress) axis to the point where the stress is being evaluated, and I is the second moment of area.

As the diameter increases, the stability increases proportionally to D3. On the other hand, as height increases, the moment M increases proportionally to H, resulting in a structurally very favorable ratio when b < 1. Araucaria's low b value can be interpreted as a consequence of this dynamic relationship—a morphological evolution that minimizes wind-induced moment increases while ensuring maximum stability with minimal diameter increase (Xu et al., 2023) (Figure 3).

Fig. 3. Relationships between mean wind speed and height-diameter allometry parameters (a) Effect of mean wind speed on the allometric exponent (b) Effect of mean wind speed on the intercept of the height-diameter relationship. Each point represents the mean parameter estimate under different wind conditions of the species. The negative slope in (a) indicates that b decreases significantly as mean wind speed increases, suggesting that stronger wind exposure suppresses vertical growth relative to diameter expansion (Yang et al., 2025).
Several studies have consistently reported that the heteromorphic growth index 𝑏 value decreases with increasing wind speed. This is because, in windy environments, trees prioritize stem thickness over vertical growth to ensure structural stability (Thomas et al., 2015; Yang et al., 2025). The low b value of Araucaria (approximately 0.6 - 0.7) is an extreme example of this trend and can be considered the result of natural structural engineering evolved in high-wind environments. The relationship in Equation 1 is not simply a biological pattern; it follows the same mathematical logic as the stability principles of structures subjected to wind loads. For example, tall buildings and towers adopt tapered structures with a decreasing diameter toward the top to distribute wind loads. The morphology of Araucaria is a biomimetic model of this "natural tapering," with the pattern of lower b values in areas with higher wind speeds being interpreted as "an optimal design solution calculated by nature" (Xu et al., 2023).
Fractal Geometry: A Tactic for Photosynthetic Efficiency
While most people (with the exception of visual artists and architects) don’t often think about it, the world we live in is composed of shapes. An architect trying to build a structure such as the Eiffel Tower (see Figure 4) must consider both the overall shape of the structure, as well as the smaller shapes that work together to create the larger image. As with everything else on Earth, the design style was not developed by humans, but the roots of this style of geometrical building can be traced back to nature. From nature’s lens, shape is important for the differentiation between species as well as for organism function (Misterio et al., 2007).

Fig. 4. Image of the Eiffel Tower revealing both its overall triangular pyramid shape as well as smaller shapes such as triangles, squares, and semicircles (shown in yellow) that are combined to make the tower (Photograph courtesy of Benh Lieu Song Wikimedia, 2025).
Foundational Geometry
Geometry can be generally split into two different branches: Euclidean and non-Euclidean geometry. Most people are more familiar and comfortable working with the former, but through time, nature has evolved to predominantly use non-Euclidean geometry, particularly fractal geometry. To understand why this is so and the potential design benefits that are present, we must first develop a foundational understanding of what both branches of geometry are.
Euclidean geometry describes the common shapes that children learn in primary school: circles, squares, triangles, cubes, etc (Misterio et al., 2007). Mathematically, the dimension of all these structures are positive integers (whole numbers) where the zero dimension represents a point, one dimension is a line, two dimensions represent a surface and enclosed objects in three dimensions have volumes. The key thing to note about Euclidean geometry is that it only deals with objects on a flat plane, so geometric objects such as a sphere or hyperbolic saddle would not be covered under Euclidean geometry (See Figure 5) (Spencer, 1999). Many fundamental mathematical rules about shapes are only true in the context of Euclidean geometry. This includes rules such as the sum of the internal angles of a triangle must be 180°, Pythagoras' theorem, and the fact that two parallel lines can never intersect (Asadov, 2023).

Fig. 5. Comparison of Euclidean and non-Euclidean geometry (Maths with Arjun, https://www.youtube.com/watch?v=NXE40t5pWfc, 2023).
In contrast, fractal geometry, first characterized by Benoit Mandelbrot, is a new way of looking at what many consider to be “irregular shapes.” At its simplest, a fractal is a pattern that is repeated over different scales, a phenomenon that is also known as self-similarity (Fractal Foundation, n.d.). It is a pattern that is seen very often in nature. We find it in snowflakes, the structure of our lungs, river branching, blood vessels, lightning, neurons, and of course, in trees (Figure 6) where the components are almost mini versions of the whole object.

Fig. 6. Examples of fractal geometry seen in nature. Top row from left to right: river branching, lighting, brain coral, snowflake. Bottom row from left to right: flower, neurons, galaxy, fern leaves (Pardesco, 2022).
Unlike Euclidean geometry, objects that exhibit fractal geometry do not have integer dimensions and neither do they have units of measurement. Instead, these irregular shapes are measured by comparing its dimension across different scales (Misterio et al., 2007).
The technique used to determine fractal dimensions in 2D is called “Box Count” (Misterio et al., 2007). A grid is superimposed over a fractal image and the number of boxes covered by the image are counted. This is then repeated with smaller and smaller sized grids. Finally, the data is plotted on a scatter graph (as a log vs log) with the x-axis showing the grid size and y-axis showing the number of boxes counted (Figure 7). If this plot produces a linear graph, the image is considered to be a fractal and the slope of that line is the fractal dimension (Misterio et al., 2007).

Fig. 7. Box counting for Koch curve using the ‘Fractalyse’ program. (a) Boxes that cover any part of the Koch curve; (b) number of covered boxes with respect to their different sizes; (c) Graph of data using the log values showing the slope and fractal dimension (Rian & Sassone, 2014).
The equivalent to Euclidean dimensions for fractals is the dimension parameter D, which describes the complexity and space-filling nature of a fractal object. It defined as seen in Equation 8 below:

Where the total number of boxes in the first and second grids is G1 and G2 while the number of covered boxes is C1 and C2 (Misterio et al., 2007).
Varied Fractal Dimension: Araucaria’s Design Solution to Photosynthetic Competition
Fractal geometry isn’t just seen in rivers and lightning, but it is also a part of the Araucaria morphology and one of its primary tools to maintain efficient transport and spatial use. The presence of fractal branching in Araucaria leaves unlock what can be described as a ‘fourth spatial dimension’ (West et al., 1999). The additional dimension is very important for one of nature’s primary goals – efficiency.
With fractals, the Araucaria’s metabolic capacity is maximized as the organization allows the plant leaves to be able to capture more sunlight, increasing the surface area available for exchange within a small area. In addition, the fractal shape creates shorter transport distance and time, boosting internal efficiency (West et al., 1999). Further still, the use of fractal structures makes Araucaria more resilient, being able to distribute mechanically stress more efficiently throughout the whole plant rather than taking damage locally (Maina, 2025).
A study carried out in 2007 by Misterio and colleagues revealed an interesting trait about Araucaria heterophylla, also known as Norfolk Island Pine. Five leaf samples were obtained from varying stem heights, and their fractal dimensions were calculated. This led to the discovery that its fractal dimension varies based on the leaf location in the plant, with leaves found near the middle having the largest fractal dimension (See Figure 8 for results) (Misterio et al., 2007).

Fig. 8. Mean fractal dimension from Araucaria heterophylla leaves across varying stem heights. The order is consecutive by height with Leaf being the highest leaf tested and Leaf 5, the lowest (Misterio et al., 2007).
Although this phenomenon has not been properly studied, a potential hypothesis for this varied branching would be photosynthetic efficiency. Being in the southern hemisphere, Araucaria heterophylla competes with so many other nearby plants, but also with itself. While the tree’s conical shape (Figure 9) can help in ensuring that lower branches receive sunlight, that may not be sufficient as internal leaves are still blocked by their higher counterparts.

Fig. 9. Image showing the conical shape of Araucaria heterophylla (Oregon State University, 2025).
Having a varied fractal geometry performs the same function as a photographer arranging people in ‘windows,’ where faces are alternating between rows, for a group photo. This helps to ensure that as many leaves as possible have access to sunlight, maximizing photosynthetic efficiency.
Fibonacci Phyllotactic Branching in Araucaria: Evolutionary Geometry in Tree Architecture
Recall on phyllotaxis: Phyllotactic branching refers to the specific pattern which leaves, branches, or cones grow around a plant’s stem. It is the natural spiral/geometric pattern by which a plant organizes itself to grow efficiently and symmetrically.
Being ancient in nature, the genus Araucaria, has evolved towards refinement in terms of geometric optimised branching. Beyond their optimised manipulation of hydraulic transports (see Araucaria Physics) and their chemical defence mechanisms throughout their wood skeletons (see Araucaria Chemistry), mathematically, this genus has reached optimal Fibonacci phyllotactic branching maximising efficiency upon various traits. As for the Fibonacci pattern itself, it can be represented as in Equation 9, where there is a visible pattern of ascending order – 1, 1, 2, 3, 5, 8, 13, … – representing far more than a mere aesthetic trait. This manifestation is one of profound biological optimization, spatial efficiency, and evolutionary conservation, for which the geometry itself reflects the intersection between developmental biology, mathematics, and adaptation.

Mathematical Basis of Fibonacci Phyllotaxis
In mathematical terms, the Fibonacci sequence is defined recursively as seen in Equation 9. When translating to biological structures, this sequence manifests itself as spiral arrangements, where the number of turns in one direction versus the other corresponds to successive Fibonacci numbers (Figure 10).

Fig. 10. Geometric representation of a Fibonacci spiral (Zolotarev, n.d.).
In Araucaria, amongst other plants, this can be seen in parastiches – a spiral line that connects plant organs (like leaves, scales, or cone bracts) that are arranged helically around a stem or cone. As seen in Figure 11 there are two sets of spirals – one going counter-clockwise (CCW), and the other clockwise (CW) – which are the parastichies themselves.

Fig. 11. Microscope sketch of the spiral symmetry of Araucaria heterophylla, for which the transverse section of the growing point of a lateral branch. Notice a CCW red line labelled 7, and a CW purple line labelled 11. Their intersection is referred to as a parastichy pair – written as [7/11] (Church, 1904).
In traditional Fibonacci sequences, there are specific phyllotactic pairs – called Fibonacci phyllotaxis ratios – which follow the pattern: 3/8, 5/13, 8/21, etc., which can be expressed as Equation 10 and 11 (Gurevich, 2020).


Here, notice that:

Given Equation 11 is satisfied, the ratio expressed in Equation 10 is called the Golden Ratio. From here, application to phyllotaxis can be further explored, where a divergence angle θ – from Equation 12 – can be determined.


When plugging in the ratios 3/8 , 5/13, and 8/21, angles of 135°, 138°, 137.6° are respectively obtained, corresponding approximately to the divergence angle to the golden ratio/sequence.
In the explored genus, the pattern becomes particularly evident in the arrangement of leaf whorls (Figure 12) and cone scales, where each successive branch whorl is offset from the previous one by the near golden angle (Burrows, 2025). This creates visible spirals that ascend the trunk in left- and right- handed helices, enabling the most efficient packing of leaves, seeds or scales around a central axis, minimising self-shading and maximising exposure to light and air (Gurevich, 2020).

Fig. 12. Example of a Fibonacci spiral in the leaves of a monkey puzzle tree (A. araucana). The blue- and red-shaded leaves represent CW and CCW spirals originating from a common leaf (Hetherington, 2023: modified by Benjamin Albers).
This mentioned, questions arise when this sequence is not followed – such as the [7/11] parastichy pair found in Araucaria heterophylla. Why has evolution chosen to include this pair? Is the pair beneficial during seedling growth?
Developmental Mechanisms Underlying Fibonacci Patterning
When considering phyllotaxis at the molecular level, Fibonacci sequences arise from self-organising chemical gradients within apical meristem. It is believed that the hormone auxin accumulates in discrete maxima that determine where new primordia (incipient leaves or branches) will form (Smith et al., 2006). Although images or micrographs of Araucaria meristem have yet to be recorded, it is thought that relatively similar to angiosperms, as each new primordium develops, it depletes auxin locally and influences the position of subsequent primordia causing a distinct layering pattern at the tip. This contributes to the spatially repeating pattern that can be observed in Figure 12.
To understand why the tree “chooses” to include non-Fibonacci pairs is not a question of choice but rather of correction. Although it is not fully confirmed why Fibonacci spirals have not been perfected in Araucaria, hitting the golden angle every time is not realistic given all the random external conditions – such as mechanical and hormonal noise – that impact spiral generation. Trees constantly make corrections to the divergence angle as it keeps generating new primordia (Gurevich, 2020). Recall the common [7/11] parastichy pair from earlier, this translates to a divergence angle of 131˚ which is still close to the golden angle (137.5˚). The next pair may be slightly larger than the golden angle at 142˚ for example. This mentioned the reason why some non-Fibonacci pairs are far more common than others – such as the [7/11] pair – is not fully understood.
Evolutionary Advantages of Fibonacci Phyllotaxis
The Fibonacci sequential pattern can be found in various plants. This includes distant cousin pine trees, sunflowers, seashells. etc. In the case of Araucaria, this pattern can be especially applied to biomechanical properties. The next few paragraphs are on topics straight out of our biomechanical essay (see Araucaria Physics), where the sequence has its place in all sections.
1. Light capture optimization
That “golden angle” of roughly 137.5° keeps leaves and branches from piling up on one another, so self-shading is minimized. That matters in a crowded forest; even a small change in overlap can mean the difference between a sunlit leaf and one stuck in shade. For tall Araucaria that push above the canopy, like A. heterophylla, spreading photosynthetic surface area efficiently along the stem boosts carbon gain overall — important when light near the trunk is stingy.
2. Hydraulic efficiency
People often focus on tracheid alignment and xylem scaling, and rightly so, but branch placement plays its part too. By spacing demands along the trunk, the spiral pattern prevents hydraulic “bottlenecks” — think of it as routing water flow across many smaller channels rather than forcing everything down a single, overloaded pipe. The result is reduced localized strain on conductive tissues.
3. Structural balance
Fibonacci-arranged branches yield near-symmetry around the axis, which improves mechanical stability. When mass is more evenly distributed, torsional stress drops — a lifesaver for trees that face coastal gales or the shifting weight of crowns on 50–70-meter specimens.
4. Reproductive efficiency
Cones with Fibonacci spirals pack seeds tightly while minimizing overlap, squeezing in maximum density without crushing developing embryos. Fossil Araucaria cones from the Jurassic and Cretaceous already show these parastichy patterns, so this geometry has been conserved for well over 100 million years.
Conclusively, on the topic of Fibonacci phyllotaxis in Araucaria, there remains a lot to learn about their persistence in keeping the sequence consistent. Although it may not be the first thing that comes to mind when thinking of tree design solutions, it has certainly been proven that Fibonacci sequences have rooted themselves deeply in Araucaria bioinformatics.
Fine Grain Patterns
The Araucaria evolved natural geometry in its fine grain which offers great structural strength and flexibility. The xylem is a tissue that transports water and nutrients from the root into the stem. In modern conifers, 90% of the xylem’s composition is made up of tracheids, whereas they constitute 95% of the Araucaria’s xylem (Esteban et al., 2024). These tracheids are long prisms which are joined longitudinally, parallel to the axis of the trunk, and they are the main structural elements of the grain’s pattern. Araucaria tracheids have diameters around 25 to 35 µm, which allows them to be packed very tightly. The tree has approximately 1300 tracheids per mm2 arranged in a hexagonal shape (see Figure 13), which allows for perfect tiling and minimizing wasted space (Evans et al., 1970).

Fig. 13. Transversal section of the Araucaria bidwillii tracheids (Osterkamp et al., 2024).
This dense and uniform packing of tracheids results in evenly distributed weight along the wood fibers, making it more resistant to bending or breaking. This dense and uniform packing of tracheids results in evenly distributed weight along the wood fibers, making the more resistant to bending or breaking. It is also very efficient for water transport, since the straight tubes greatly increase the flow of water, and the dense packing allows a maximized transport from the roots (Cuny et al., 2023).
Tracheid Wall Thickness
Some interesting geometric changes occur in tracheid structure as the amount of growth rings increase in trees of the Araucaria genus. The further tracheids are from the pith (i.e., the older growth rings at the center), the larger the diameter becomes, the thicker the tracheid walls become and the longer the tracheids get (see Figure 14).

Fig. 14. Radial variation in a) tracheid length, b) tracheid wall thickness and c) tracheid diameter as growth ring number (x-axis) increases (Santos et al. 2015).
This is called a “Typical Radial Pattern,” where cell properties change when moving away from the center to the bark (Santos et al. 2015). As the tree grows, it gets taller and more growth rings appear further from the center. Tracheids adapt to the tree’s height which is why the ones far from the pith (younger) are longer. The tracheid radius changes with the tracheid’s length following the Hagen-Poiseuille Law (Equation 13), which states that:

where
Δp is the pressure difference
L is the length of the pipe
µ is the dynamic viscosity of the fluid
Q is the volumetric flow rate
R is the pipe radius
Since the flow rate (Q) is inversely proportional to the length (L) and proportional to the radius (R4), the radius slightly increases with the length (Elias, 2024). The increase in cell wall thickness is necessary for mechanical support of the tree’s growing height, so it trades off some hydraulic efficiency for a stronger grain which can withstand more weight (Santos et al. 2015). This design solution allows tracheids to adapt to the demands of the tree’s various life stages.
The Araucaria’s finely grained stem makes use of tracheid geometrical properties to maximize the efficiency of water and nutrient transport from the roots and to strengthen its wood anatomy to increase its resistance to bending and breaking.
Conclusion
In summary, the Araucaria has stood for millions of years as a living synthesis of mathematical precision. Its adaptations demonstrate a maximization of geometrical and mechanical efficiency. The Araucaria’s use of the allometric scaling law provides a stable structure through its height-diameter relationship. Fractal geometry in its branching patterns maximizes light absorption efficiency. This genus’ branches and leaves are arranged to follow the Fibonacci spiral, which benefits photosynthesis and mechanical strength. Moreover, the tracheid properties and geometric pattern in the fine grain ensure efficient water flow and structural strength.
From this small sample size, it is clear to see that the Araucaria rose to the top through a series of well-designed mathematical structures that have clearly withstood the test of time. This harmony between mathematics and biological adaptations transforms the Araucaria from a mere botanical organism into a model of natural engineering. To study the Araucaria is to examine nature’s way of weaving mathematics into the making of every living being. Anyone aspiring to build structures that will last generations thriving through the fluctuations of climate and seasons has a lot to learn from Araucaria.
References
References
Asadov, A. (2023). Applications of Geometry: Understanding the Differences and Similarities between Euclidean and Non-Euclidean Geometrie. Research & Reviews: Journal of Statistics and Mathematical Sciences, 9(1). https://doi.org/10.4172/J Stats Math Sci.9.1.004
Burrows, G. E. (2025). Ovulate cone and seed biology of Wollemia Nobilis (Araucariaceae) and comparison with Agathis microstachya and Araucaria cunninghamii. Australian Journal of Botany, 73(6). https://doi.org/10.1071/bt25036
Chung, Y. A., Ke, P., & Adler, P. B. (2023). Mechanistic approaches to investigate soil microbe‐mediated plant competition. Journal of Ecology, 111(8), 1590–1597. https://doi.org/10.1111/1365-2745.14156
Church A.H. (1904) On the Relation of Phyllotaxis to Mechanical Laws. London: Williams and Norgate, 1904, 353 p. https://doi.org/10.5962/bhl.title.57125
Cuny, H. E., Rathgeber, C., Frank, D., Fonti, P., & Fournier, M. (2014). Kinetics of tracheid development explain conifer tree‐ring structure. New Phytologist, 203(4), 1231–1241. https://doi.org/10.1111/nph.12871
Elias, K. (2024). Law of Hagen-Poiseuille. CARPentry. https://carpentry.medunigraz.at/examples/tutorials/tutorials.06_fluid.0…
Enquist, B. J., West, G. B., & Brown, J. H. (2009). Extensions and evaluations of a general quantitative theory of forest structure and dynamics. Proceedings of the National Academy of Sciences, 106(17), 7046–7051. https://doi.org/10.1073/pnas.0812303106
Esteban, L. G., de Palacios, P., Heinz, I., Gasson, P., García-Iruela, A., & García-Fernández, F. (2023). Softwood anatomy: A Review. MDPI. https://www.mdpi.com/1999-4907/14/2/323
Evans, P. D., Mundo, I. A., Wiemann, M. C., Chavarria, G. D., McClure, P. J., Voin, D., & Espinoza, E. O. (1970). Identification of selected CITES-protected Araucariaceae using dart TOFMS. US Forest Service Research and Development. https://research.fs.usda.gov/treesearch/55216
Fractal Foundation. (n.d.). Branching fractals. Fractal Foundation Online Course - Chapter 1 - FRACTALS IN NATURE. https://fractalfoundation.org/OFC/OFC-1-1.html#:~:text=A%20fractal%20is…;
Gurevich, D. (2020). Discrete lattices on the single bearing spiral: From botany to music. Symmetry: Culture and Science, 31(4), 449–463. https://doi.org/10.26830/symmetry_2020_4_449
Krauss, K. W., Twilley, R. R., Doyle, T. W., & Gardiner, E. S. (2006). Leaf gas exchange characteristics of three neotropical mangrove species in response to varying hydroperiod. Tree Physiology, 26(7), 959–968. https://doi.org/10.1093/treephys/26.7.959
Maina, M. (2025, May 26). Fractals in nature - the hidden geometry of the natural world. Innova Writers. https://blogs.innova.co.ke/fractals-in-nature/#:~:text=Branching%20patt…;
Maths with Arjun. (2023, January). What Does Non-Euclidean Geometry Mean. YouTube. https://www.youtube.com/watch?v=NXE40t5pWfc
Misterio, J., Ravindra, K., Rivero, R. D., McCloud, H., Burr-Alexander, L., & Ravindra, N. (2007). Variation of fractal dimension of leaves based on stem position. 2007 Annual Conference & Exposition Proceedings, 12.1585.1-12.1585.12. https://doi.org/10.18260/1-2--2852
Niklas, K. (1995). Size-dependent allometry of tree height, diameter and trunk-taper. Annals of Botany, 75(3), 217–227. https://doi.org/10.1006/anbo.1995.1015
Oregon State University. (2025). Landscape plants. Araucaria heterophylla | Landscape Plants | Oregon State University. https://landscapeplants.oregonstate.edu/plants/araucaria-heterophylla&n…;
Osterkamp, I. et al. (2024). Changes of wood anatomical characters of selected species of araucaria- during artificial charring - implications for palaeontology. Acta Botanica Brasilica. https://www.academia.edu/94430076/Changes_of_wood_anatomical_characters…;
Georgelin, E., & Loeuille, N. (2015). Evolutionary response of plant interaction traits to nutrient enrichment modifies the assembly and structure of antagonistic‐mutualistic communities. Journal of Ecology, 104(1), 193–205. https://doi.org/10.1111/1365-2745.12485
Pardesco. (2022). Fractal geometry. https://pardesco.com/blogs/news/fractal-geometry?srsltid=AfmBOophg11KoH…;
Pellecchia, M., Güntert, P., Glockshuber, R., & Wüthrich, K. (1998). NMR solution structure of the periplasmic chaperone FimC. Nature Structural Biology, 5(10), 885–890. https://doi.org/10.1038/2325
Rian, I. M., & Sassone, M. (2014). Fractal-based generative design of structural trusses using iterated function system. International Journal of Space Structures, 29(4), 181–203. https://doi.org/10.1260/0266-3511.29.4.181
Sandy Hetherington. Plant Evolutionary Biologist, & Holly-Anne Turner. PhD Candidate. (2023, June 16). How a 400 million year old fossil changes our understanding of mathematical patterns in nature. The Conversation. https://theconversation.com/how-a-400-million-year-old-fossil-changes-o…;
Santos, C. M., Starzynski, R., Longui, E. L., Romeiro, D., Lima, I. L. de, & Florsheim, S. M. B. (2015). RADIAL VARIATION OF TRACHEID FEATURES, SPECIFIC GRAVITY AND GROWTH RINGS IN Araucaria angustifolia (Bertol.) Kuntze PLANTED IN CUNHA-SP. Revista Do Instituto Florestal, 27(2), 127–135. https://doi.org/10.4322/rif.2015.009
Smith, R. S., Guyomarc’h, S., Mandel, T., Reinhardt, D., Kuhlemeier, C., & Prusinkiewicz, P. (2006). A plausible model of Phyllotaxis. Proceedings of the National Academy of Sciences, 103(5), 1301–1306. https://doi.org/10.1073/pnas.0510457103
Spencer, P. (1999, April 19). Euclidean geometry. Question Corner -- Euclidean Geometry. https://www.math.toronto.edu/mathnet/questionCorner/euclidgeom.html#:~:…;
West, G. B., Brown, J. H., & Enquist, B. J. (1999). The Fourth Dimension of Life: Fractal geometry and allometric scaling of organisms. Science, 284(5420), 1677–1679. https://doi.org/10.1126/science.284.5420.1677
Wikimedia. (2025, October 9). Eiffel Tower. Wikipedia. https://en.wikipedia.org/wiki/Eiffel_Tower
Xie, A., Gee, C. T., & Griebeler, E. M. (2024). Modelling height–diameter relationships in living Araucaria (Araucariaceae) trees to reconstruct ancient Araucarian conifer height. Palaeontology, 67(2). https://doi.org/10.1111/pala.12693
Yang, C., Liao, R., Huang, S., Cheng, Y., & Zhou, S. (2025). Wind speed and soil properties drive the height-diameter allometric pattern of island plants. Frontiers in Plant Science, 16, 1548664. https://doi.org/10.3389/fpls.2025.1548664
Zolotarev, V. (n.d.). Golden Ratio Fibonacci. A spiral for harmony, composition, logos and designs. correct proportions. Vecteezy. https://www.vecteezy.com/vector-art/5851724-golden-ratio-fibonacci-a-sp…