
Table of Contents
Keywords: Coral population dynamics, bilateral symmetry, biradial symmetry, symmetry, reaction-diffusion models, paleozoic corals, fractal geometry, hyperbolic geometry, conservation
Abstract
Coral reefs exhibit a multitude of growth forms and patterns, inspiring many applications of design in society today. Understanding these fundamental patterns stems from a mathematical analysis of these organisms on an individual and colony-wide scale. This paper aims to analyze coral reefs using the mathematical notions of geometry, symmetry, population growth and dynamic models. Fractal geometry is a branch of geometry that deals with self-similarity and repeated patterns on different scales; it can be used to analyze corals to provide more accurate descriptions of texture and morphology of septa and calyces which cannot be achieved using classical Euclidean geometry. Hyperbolic geometry is also useful for describing corals, as it can be used to describe the frills and properties of surface area that help corals maximize nutrient absorption. Like most objects in the natural world, corals display forms of symmetry that are not only beautiful to observe but also serve evolutionary purposes. Corals exhibit radial and bilateral symmetry, which, when investigated further, is found to be related to the number of mesenteries and septa contained by the organism. Finally, this paper will discuss the use of mathematical models for describing population dynamics and the large-scale growth models of coral colonies around the world, providing insight into the crisis they face and the potential for recovery after human disturbances.
Introduction
Corals exhibit incredibly beautiful and complex growth patterns both on the individual scale of single polyps and the large-scale development of coral colonies. These growth forms rely on a multitude of factors such as temperature, light exposure, and wave action and can be classified into types such as fringing, barrier, atoll, and more. Fascinatingly, although each species of coral displays unique colours, shapes and structures, a mathematical analysis of the symmetry and geometry of these organisms reveals significant similarities in the fundamental structures that compose them.
As mentioned in Coral Physics, coral reef colonies are made up of individual polyps that secrete their own skeletal walls called corallites with fascinating displays of radial symmetry related to the number of mesenteries and septa that they have. The skeletal elements of these single polyps are joined to those of their neighbours through the coenosteum, resulting in different overall colony forms depending on the type of coral. The process of formation of the coral skeleton relies on chemical processes of biomineralization involving pH and ions, as discussed in Coral Chemistry. However, despite the heavy reliance on the coral’s environment for skeletal development, common patterns in symmetry and geometry can be found in corals all around the world. These forms become particularly interesting when considering branches of mathematics other than Euclidean geometry, such as fractal and Gaussian geometry, as topics such as negative curvature and fractal dimension become of interest.
Mathematical analyses are not only useful for studying the physical structures and appearance of corals but are also incredibly helpful for depicting population dynamics and growth models at larger scales. This is becoming increasingly important as coral reefs are falling more and more in danger due to climate changes that are crucially affecting the pH and ocean environment of these organisms, meaning these models could be part of the preliminary steps in saving these captivating ocean creatures.
Geometry
Fractal Geometry
Fractal geometry is a branch of mathematics that can be incredibly useful for describing the complex, rough, and porous structures found in corals. This area of mathematics describes shapes with uneven contours like those found in nature and is complementary to Euclidean geometry. The principal requirement for an object to be considered fractal is to display inherent and repeating similarities, i.e. zooming in and out of the fractal pattern will show different-sized copies of the same shape (Pardesco, 2024). The main concept in fractal geometry is the quantification of fractal dimensions, which allows us to describe the roughness and texture of objects. The distance, surface, or volume being measured, is taken as a unit of measurement which is then covered with boxes. Boxes with dimensions corresponding to various possible distances between two points in the structure need to be included in order to define its dimension; in other words, the boxes are used as a “ruler” to be able to analyze the structure at many scales to study the self-similarity at all magnifications. The fractal dimension of lines is 1, surfaces have a fractal dimension of 2, and solid bodies have a fractal dimension of 3. Dimension characterises how the length between two points increases as scale decreases and is proportional to roughness (Martin-Garin et al., 2007).
One of the most common examples of fractal sets is the Mandelbrot set shown in Figure 1. It is generated using an iterative algorithm, meaning it builds upon previously obtained answers to solve complex problems. The algorithm starts with a complex number c, and each for iteration the result is squared then added to the original value c. The process is repeated for each point in the complex plane and if the absolute value remains bounded after enough repetitions, it is part of the Mandelbrot set (Pardesco, 2024).

Fig. 1. The Mandelbrot set which exhibits repeated patterns at increasing magnifications. (Zaczyński, 2023).
A study used the fractal approach to study 4 corals: Aplosmilia, Eusmilia, Dichocoenia, and Montastraea. The study used to Box Method, which involves laying a square mesh grid of different sizes over the image of the object and counting how many boxes are needed to cover it completely. A software called HarFA was used to implement this method, with boxes of sizes 2-100 pixels. NB defined the number of black squares that fully covered the object, NBW quantified the number of squares that partially covered the object, and NW was the number of squares that did not cover the object at all. NB and NW were used to calculate the fractal dimensions δB and δW which are useful for Euclidean objects like circles, lines, etc. NBW was used to calculate the fractal dimension δBW which is useful for objects with rough and jagged perimeters. A statistics software called STATVIEW was used to create four columns: AX, AY, BX, and BY. AX and AY contained log (r) (r being the box size) and log (NBW) while BX and BY remained blank. A Richardson plot was created with log(r) on the x-axis and log (NBW) on the y-axis, giving a log function with an apparent inflection point (shown by the arrow in Figure 2). This inflection point was found by transferring the last data columns of AX and AY into BX and BY to create a new bivariate plot, providing two slopes given by equation 1 (Martin-Garin et al., 2007):


Fig. 2. Richardson Plot of box size versus the number of black and white boxes need to cover the object (in a log-log coordinate system) (Martin-Garin et al., 2007).
Using two slopes instead of one allowed them to find the Euclidean slope (equal to 1) and a second data line of slope that did not equal 1 and was related to the texture of the object. The coefficients of both least squares of regression (a mathematical regression analysis that helps determine the line of best fit for a set of data) are identified as the fractal dimensions. Textural fractal dimension (δt) is used to describe details at the septal level while structural fractal dimension (δs) describes the characteristic morphology and overall structure of the corallite. Morphologies that had more complex septa and calices had higher δt and δs values; furthermore, higher δs was related to lower variability in δt than in cases of lower δs. This class of geometry is very useful, as it allows us to study morphology of the surface between the living body and skeleton of a coral (also known as the polyp/skeleton interface) which is important for its overall shape (Martin-Garin et al., 2007).
Hyperbolic Geometry
The coral reef has negative curvature (Fig. 3) and is an example of a finite, hyperbolic plane in nature. Hyperbolic patterns are inherently non-Euclidean as they do not align with the fundamental assumptions of Euclidean geometry. For instance, in Euclidean geometry, the sum of the angles in a triangle is always exactly 180°, but in hyperbolic geometry, the sum of the angles in any triangle is always less than 180° (Bolyai, 2013). This property stems from the negative curvature of hyperbolic surfaces, which causes lines and shapes to behave differently from flat Euclidean spaces.

Fig. 3. An example of negative curvature, which is often referred to as a saddle because of its shape (Hurley, 2023).
The Universal Hyperbolic Theorem explains a fundamental property of hyperbolic geometry and highlights a unique characteristic that is not found in Euclidean geometry. It states, “In hyperbolic geometry, for every line l and every point P not on l there pass through P at least two distinct lines parallel to l. In fact, there are infinitely many lines parallel to l through P (Bolyai, 2013).” This relationship is depicted in Figure 4, where multiple lines pass through a point and display the possibility of infinite parallels.

Fig. 4. The existence of infinite parallels as outlined in the Universal Hyperbolic Theorem (Bolyai, 2013).
The development of hyperbolic geometry is beneficial for corals as its negative curvature increases the surface area of the coral itself in limited space. This increased surface area leads to greater efficiency in nutrient absorption from the coral’s surroundings. While they may display hyperbolic geometry, corals do not appear as perfect, infinite hyperbolas. Polyp growth is limited by the surrounding environment. It is still important to maximize surface area, therefore the result of the negative curvature of polyps in the limited space is frilled, crenulated structures that optimize surface area (Fig. 5), allowing for efficient nutrient absorption and interaction with symbiotic algae (Fields, 2010).

Fig. 5. A vibrant coral colony with frilly, hyperbolic structures characterized by their negative curvature, with maximized surface area allowing for efficient nutrient absorption and interaction with its environment (Ruffles, Corals, and the Hyperbolic Plane, 2012).
While these structures and their benefits for corals are fascinating, it presents the question of quantifying coral growth. The frilly and random structure of the polyps can be quantified using a reaction-diffusion model for growth which considers nutrient concentration and diffusion.
Reaction-Diffusion Models for Growth
A reaction-diffusion type mathematical model was derived by considering a water tank filled with coral larvae. Nutrients were provided to the surface of the tank. The coral consumed these nutrients and in return produced their solid skeleton. The relationship between the nutrients and products is demonstrated in Equation 2 (Mistr & Bercovici, 2003).
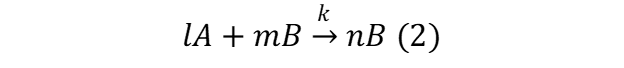
Equation 2. Relation between absorbed nutrients and solid products, where k is a positive rate constant, l, m and n are the respective stoichiometric constants such that l + m = n.
The change in the nutrient concentration over time, ∂A/∂t, is influenced by two different factors: the diffusion of nutrients through the tank and the rate at which they are consumed by the coral. Similarly, the growth of the skeleton, represented by B, depends on the reaction rate and nutrient availability. These relationships can be expressed mathematically in Equation 3 and Equation 4.

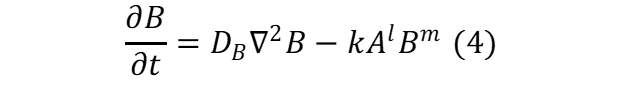
Equation 3, 4. The reaction-diffusion dynamics of coral growth, where DA and DB are the diffusion coefficients for A and B, respectively, and AlBm is the reaction term, indicating how nutrients are consumed, and products are formed.
This model shows that nutrient diffusion ensures non-uniform growth but demonstrates the relationship between nutrient concentration and growth speed. Areas with higher nutrient concentrations experience faster growth than regions with lower concentrations. These nutrient imbalances create the frilled and hyperbolic patterns displayed by corals (Mistr & Bercovici, 2003).
It is important to note the available space for growth in an environment plays a critical role in the overall structure of corals. Confined spaces lead to more pronounced negative curvature, and tightly packed, crenulated structures, while open environments that are not constrictive to growth lead to broad patterns that expand farther outward (Mistr & Bercovici, 2003).
Reaction-diffusion models highlight the dynamic and adaptive nature of coral growth and provide a mathematical explanation for how hyperbolic structures arise in coral reefs. These patterns are not only aesthetically striking but also biologically efficient, demonstrating the profound connection between mathematical principles and natural forms.
Symmetry
Symmetry occurs everywhere in nature from the bilateral symmetry in starfish to the radial symmetry in corals. Most of the time, symmetry is developed for evolutionary purposes (i.e. kangaroos are bilaterally symmetrical because they can be split by an axis with their left foot and right foot mirroring each other, giving them the ability to walk). Additionally, symmetry can be useful in mathematical modeling. For example, the symmetry of rectangles is used to approximate the area under the curve (i.e. an integral) by taking the limit as the number of rectangles approaches infinity.
Hexacorals vs Octocorals
Recall from Coral Physics that marine invertebrates, such as corals and jellyfish, are part of the phylum Cnidaria. Corals, themselves, belong to the Anthozoa class. This class is divided into three subclasses: octocorallians, hexacorallians, and ceriantharians (https://userweb.ucs.louisiana.edu/~scf4101/Bambooweb/MoreAboutCoral.htm). A key difference between hexacoral and octocoral is the fact that octocorals are typically soft corals while hexacorals are hard corals. Unlike hexacorals who have hard exoskeletons, octocorals have small calcareous sclerites in their body, providing structure (Fabricius, 2024) while hexacorals are known as reef builders (https://www.endangeredspeciesinternational.org/coralreefs.html).
All corals exhibit a radial and bilateral symmetry. The Google definition of radial symmetry is the “symmetry around a central axis,” which is characterized by the number of mesenteries or septa corals have. As mentioned in Coral Physics, mesenteries are soft tissues that provide structural support to the coral polyp. The number of mesenteries is typically equal to the number of tentacles in a coral (fig. 6). Additionally, the radial symmetry could also be characterized by the septa. Septa are the plates that divide the corallite (which is the skeletal part of the coral) (https://cdhc.noaa.gov/coral-biology/coral-skeleton/).
Conversely, bilateral symmetry refers to “having equal arrangement of parts about a vertical plane” (Animal Characterization Based on Body Symmetry). Hexacorals and octocorals differ in their radial symmetry. Hexacorals exhibits six pairs of mesenteries, giving them a hexameral symmetry while octocoral have eight pairs of mesenteries, or tentacles. Hexacorals exhibit both a hexaradial and biradial symmetry (Grebelnyi & Ivanova, 2023), which is attributed to its two siphonoglyphs, placed at opposite ends of the flattened pharynx. Siphonoglyphs are grooves along the actinopharynx that aid in water movement throughout the polyp (fig. 6). Furthermore, hexacoral’s septa are arranged hexametrical as well. On the other hand, octocorals only exhibit octaradial symmetry from their mesenteries and their septa (fig. 7). Interestingly, the radial symmetry in all corals is acquired during the formation of mesenterial pairs where one mesentery is formed on one side and the other mesentery is formed on the opposite side (Grebelnyi & Ivanova, 2023). Octocorallia has a bilateral symmetry where two mesenteries have ciliated grooves used to funnel water our while the remaining mesenteries have gonads.

Fig. 6. Illustrates the anatomy of a coral with its mesenteries and actinopharynx (Coral Polyp Anatomy).

Fig. 7. Octocoral’s bilateral symmetry (Malakhov, 2016).
Symmetry of Paleozoic Corals
Paleozoic corals refer to corals originating from the Paleozoic era, which occurred 541 million years ago to 252 million years ago (Paleozoic). Paleozoic corals existed until the Permian extinction, which is theorized to kill about 90 percent of the planet’s species (Hoffman). Occurring 250 million years ago, the Permian extinction resulted in less than 5 percent of the marine animal survival. Known as the one of the mass extinctions, the Permian extinction was caused by the warming of Earth’s climate and its associated oceanic changes followed by extreme volcanic activity (https://samnoblemuseum.ou.edu/understanding-extinction/mass-extinctions…). While most are extinct, Paleozoic corals had unique shapes that continues to be seen in corals today. There are currently 5 known orders of Paleozoic corals: Rugosa, Tabulata, Heterocorallia, Cothoniida, and Kilbuchophyllida. These Paleozoic corals exhibited interesting and unique symmetry.
Paleozoic corals’ symmetry is evaluated based on their cross-sectional shapes, considering the number of septa (and their locations). For example, symmetry can be characterized by a conical or an auloporoid shaped base with rounded and elliptical cross-sectional shapes. The conical shape provides a radial symmetry while the auloporoid shape is more bilateral. Interestingly, Paleozoic corals share the characteristic of auloporodity. Described by the “curvature of the conical bases of corallites in the initial stage of growth,” auloropoidity is strongly pronounced in Tabulata and Rugosa corals (Ospanova, 2023). The term auloporidity originates from the structure that is characteristic of the genus Aulopora. Since the septa develop in the coral skeleton, researchers theorize that it may be affected by porosity development (refer to Coral Physics for more about porosity).
Interestingly, corals’ bilateral symmetry is attributed to harsh oceanic conditions (i.e. strong currents). A bilateral symmetry provides greater bodily stability due to the nature of the curved axis. The bilateral symmetry was most pronounced in Rugosa corals. Rugosa corals were tetracorals that had a plane of symmetry, distinguished by the position of the cardinal septum and attachment scar being on the same side (Rozhnov, 2014). As mentioned before, this symmetry is caused by the development of formation of the septa. First, the planula develops, followed by the development of a long aseptal calyx. After, the cardinal septum and the counter septum appear (on opposite sides of each other). Then, a united axial septum begins to form when the cardinal and counter septum come in contact by their internal edges. Finally, the remaining pairs of septa appear, forming a beautiful pattern distinctive to Rugose corals (Rozhnov, 2014) (fig. 8). More importantly, tetraradial corals today originate from the Rugosa corals. Conversely, other Paleozoic corals had a variety of corals that had different types of symmetry. Examples range from Heliolitida which had 12-ray symmetry (meaning they had 12 septa formations) to Oskaria corals that only had 6-ray symmetry (Ospanova, 2023).

Fig. 8. Formation of septa, which causes a beautiful pattern to appear in Rugosa corals (Rozhnov, 2014).
As a result, Paleozoic corals’ symmetry continues to be seen today, with corals still exhibiting bilateral and radial symmetry to this day. This symmetry evolved to stabilize corals from harsh oceanic environments including currents, strengthening their bases.
Population Dynamics
Population Growth Factors
Coral polyps reproduce through a process known as spawning, where once a year, following a full moon, coral colonies simultaneously release billions of gametes into the water. This synchronous spawning tactic maximizes the probability of reproductive success. The high concentration of gametes in the water both increases the likelihood of sperm encountering eggs and decreases the distance that sperm must travel to encounter an egg. In addition, the high number of gametes is a defense mechanism against predation, as predators that may prey on coral gametes are overwhelmed by the sheer number of sperm and eggs in the water. Mass spawning is also beneficial in promoting genetic diversity and mutations. Many different coral colonies releasing gametes simultaneously increases the probability of producing offspring with beneficial survival adaptations.
Coral spawning occurs once a year over several days and is affected by several factors, including water temperature, solar exposure, lunar patterns and precipitation. Coral spawning first begins following a full moon, since light levels are lower during the shift from full moon to new moon. Lower light levels make it more difficult for predators to detect coral polyps, leading to a higher survival rate for the new coral larvae (University of Tokyo, 2024). The first spawning date is heavily influenced by the temperature of the water in the 60 days preceding it: higher average water temperature will lead to an earlier first spawning date. Spawning peaks when the water reaches an ideal temperature, which varies by species, but falls between 25-29°C. Precipitation and daylight cycles reinforce these temperature cues, indirectly affecting spawning timing (Sakai et al., 2024). When ideal conditions are met, as high as 80-90% of the coral population will release their gametes during this peak window.
However, coral population growth is not guaranteed following reproduction, as coral larvae must be able to survive and settle within the reef. The growth of a coral colony is contingent on a host of factors from size of the reef to fecundity rate of the polyps. These factors were explored by Tom Shlesinger and Robert van Woesik in a study that attempted to apply a mathematical model to estimate the impact of each of these factors on the growth rate of 2 species of corals: Dipsastraea favus and Platygyra lamellina. Using integral projection models (IPMs), population growth can be estimated as a function of colony size and time. The general form of an IPM is:

where nt(x) represents the initial size distribution of members of the colony and nt+1(y) represents the size distribution at the second recorded time. K(y,x) represents what is referred to as the full kernel and is made up of a growth/survival kernel and a fecundity kernel. The growth/survival kernel is simplified to the product of the survival probability at size x and the growth from x to y. The fecundity kernel is more comprehensive, being made up of factors more specific to the studied species such as fecundity rate and establishment probability (Merow, 2014). In Shlesinger and van Woesik’s study (Shlesinger & van Woesik, 2021), this kernel was represented as the product of the probability of both the colony and an individual polyp within the colony being fertile, the function representing the maximum number of oocytes a colony of a given size can produce, the size distribution of larval recruits, and the establishment probability of the recruits. The full kernel is then used to generate a large matrix where each cell represents the probability for the colony to grow from size x to size y at any given point in its life cycle. The eigenvalue of this matrix can then be taken to represent the growth rate of the colony per interval of time. The study found similar growth rates in colony size for both species: 1.67 ± 1.08 cm for Dipsastraea favus and 1.82 ± 1.01 cm for Platygyra lamellina (Shlesinger & van Woesik, 2021). However, the eigenvalues for each colony were different (1.097 and 0.957 respectively). This would suggest that despite both colonies seeing similar increases in size over the same interval from 2015 to 2018, the population of Dipsastraea favus increased by approximately 7.1% whereas the population of Platygyra lamellina decreased by 4.3%.
This study related the factors that contribute to growth to the size of the colony. In theory, larger colonies will release more gametes and have more area available for larval settlement, leading to increased growth. Figure 9, the graph below, seems to support this.

Fig. 9. graphs relating reproductive factors to colony size for both Dipsastraea favus (in blue) and Platygyra lamellina (in green). It should be noted that size is given on a log scale, not linear. A value of 2.3 represents e2.3 or approximately 10 cm. Fecundity represents the number of oocytes per colony. F) represents the size frequency distribution of coral recruits (Shlesinger & van Woesik, 2021).
For each of these factors, colony size benefits reproduction and survival chances. As seen in graphs A and D, every mortality observed occurred among colonies less than 10 cm in diameter. Furthermore, the reproductive ability of the coral colony increased exponentially with size (graph c), leading to significantly higher reproductive success (graphs d and e). This data supports the evolutionary advantage of mass spawning, as corals find reproductive success is size and numbers.
Autocatalytic Growth Patterns of Coral
As discussed above, coral colony size has a direct impact on reproductive success. It is one of the most influential factors in coral growth both in encouraging and in limiting reproduction. Coral growth can be estimated as a differential equation based on a reaction-diffusion system. The equation below (Lam & Lou, 2022) describes coral growth as a function of size and time based on existing coral mass and the availability of nutrients.

In the above equation, C(x, t) is a function of coral biomass at a given time and position. D∇2C is referred to as the diffusion term, where D is the diffusion coefficient representing the ability of coral to spread across an area and ∇2 is the Laplace operator representing the tendency of coral biomass to diffuse from areas of high density to areas of low density. R(C, N) is the reaction term which models growth rate as a function of existing biomass and nutrient availability. -μC is the mortality term and accounts for the natural rate of death among the coral colony. Diffusion allows coral to spread account across space over time, leading to the development of colonies. As the equation shows, the rate of growth is higher among large colonies due to protection from predation, increased settlement area, and higher release of gametes, among other factors.
However, one important benefit of size is nutrient trapping. Large colonies of corals can slow water flow, keeping particles, including coral larvae and nutrients, closer to the body of the reef. Increased nutrient availability facilitates coral growth, thus growing the colony, and further enhancing the nutrient-trapping ability of the reef. This creates a feedback loop, referred to as localized growth amplification, where within a reef, there will be hotspots of enhanced development, causing corals to expand disproportionately towards areas with favorable conditions (Mistr & Bercovici, 2003). Over time, this leads to the development of well-defined patterns in coral growth, such as ridges or stripes, which are aligned with water flow around the coral colony. The autocatalytic growth tendency of corals makes them highly susceptible to changes in environmental conditions earlier in reef development, and less so once the reef is already established. Changes in water flow or nutrient availability can cause smaller reefs to grow in a different direction since they are less resistant to wave forces than larger reefs. For this reason, initial water conditions can have a dramatic effect on the patterns formed by reef growth. This pattern is continuously propagated by localized growth and feedback loops as the reef grows.
Nutrient availability is also a major factor in limiting coral growth. While autocatalysis promotes growth, resource limitations ensure that corals do not grow unchecked. The finite availability of nutrients means that coral polyps must compete with other nearby polyps for resources. When the colony overgrows in a certain area, the demand for nutrients exceeds the supply, effectively halting the growth of the reef in that direction. In addition to nutrients, corals also compete for light. A study out of Bar-Ilan University examined corals as light collectors, finding that there is a negative correlation between reef size and photon collection per unit area, as shown in figure 10 below.

Fig. 10. Photon absorption density as a function of coral area. (A) represents Acropora coral and (B) represents Millepora (Stambler & Dubinsky, 2005).
As shown in the graphs above, light absorption per unit area decreases as the size of the colony grows. This is indicative of competition for light between coral polyps. Since corals rely on the energy provided through photosynthesis by zooxanthellae, light becomes a limiting factor in coral growth, as zooxanthellae are unable to provide enough energy once the colony becomes too big.
Reef Crisis Population Dynamics
In recent decades, coral reefs have suffered alarming declines in biodiversity and biomass, driven by human-induced environmental disturbances. These disturbances can be classified as near-field or far-field impacts. Near-field impacts include immediate, localized stressors such as point-source pollution and overfishing, which directly impact coral reefs within proximity to human activities. By contrast, far-field impacts refer to global environmental changes—like climate change, sea-level rise, and ocean acidification—that influence coral reefs even in remote areas far from human settlements. As human populations grow and migrate further inland, these far-field impacts are expected to increase due to processes like watershed degradation and sediment deposition, which funnel pollutants into ocean ecosystems and worsen the strain on coral reefs (Riegl et al., 2009). The relationship between human density, which increases near-field and far-field impacts, and the biomass of two coral reef biomes is depicted in Figure 11 below.

Fig. 11. Trajectory of coral cover and human density in A) the Caribbean and B) the Persian Gulf. Notice the inverse relationship between the two lines, signifying that the success of our species has a direct negative correlation with the biomass of the coral reef (Riegl & Glynn, 2020).
From an ecological standpoint, the effects of human-driven disturbances on coral reefs can be broadly grouped into three main categories: increased mortality, slowed recovery, and habitat destruction (Riegl & Glynn, 2020). Accounting for these effects on a single coral colony leads to a bleak conclusion, with little to no opportunity for survival. However, coral reefs cannot be considered as independent entities. Coral populations usually grow in discrete patches with well-defined boundaries, making them particularly suitable for analysis through the island biogeography model. This defines each coral colony as an analog to an island-dwelling species, which is heavily dependent on migration rates and habitat sizes (Riegl & Glynn, 2020). This model allows coral reefs to be viewed as part of a metapopulation—a network of smaller, interlinked populations that are geographically separated yet capable of exchanging individuals or genetic material via migration.
The metapopulation model allows ecologists to predict how coral reefs could recover after human disturbances, especially in fragmented or degraded environments (Riegl & Glynn, 2020). In a metapopulation, certain reef patches may face local extinctions due to severe disturbances, but nearby healthy patches can act as “rescue” sites by dispersing coral larvae to repopulate these areas—a process known as the rescue effect (Hansen, 1999). This dynamic helps damaged reefs regenerate and supports the metapopulation's overall stability, enhancing the coral ecosystems' resilience. Near-field impacts benefit most from this impact, as their range is often limited to the origin site (Riegl & Glynn, 2020). This allows coral colonies that weren’t impacted to quickly recolonize the region and return to previous levels of biodiversity. This process can be modelled mathematically using the Levins model, or Equation 7, with the following parameters: the probability a patch is occupied (P), the colonization rate (c), and the extinction rate (e) (Levins, 1969).

This model assumes colonization occurs when larval dispersion from other patches encounters an unoccupied patch. If the first term of the equation, which is dependent on the colonization rate, is higher than the second, which depends on the extinction rate, the metapopulation can “rescue” other colonies. The Levins equation is an analog of logistic growth, with the carrying capacity of the metapopulation occurring when the population is at equilibrium or when the growth rate is zero as shown in Equation 8 (Levins, 1969).
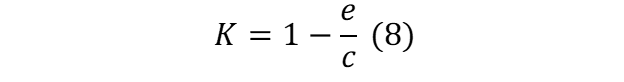
Therefore, the equilibrium patch occupancy depends on the ratio between the extinction and colonization rates of the metapopulation. Coral metapopulations with higher colonization rates and lower extinction rates will, therefore, have a higher carrying capacity. Furthermore, the growth rate of new patches is simply described as the colonization rate minus the extinction rate. This means a metapopulation that has a higher colonization rate will be able to “rescue” other colonies even when the extinction rate rises from a disturbance (Levins, 1969).
The Levins model, unfortunately, is not a great representation of crisis dynamics for coral reefs. As a deterministic model, the Levins model struggles with metapopulation processes that are typically stochastic. For example, the Levins model cannot be used to calculate the viability of a coral colony. Additionally, each colony's reproductive strategies and dispersal technique have implications for the colonization and extinction rates that the model does not account for (Keymer, 2000).
More comprehensive models utilize two additional parameters: area (a) and the distance scalar between two colonies (τ). Each model can sustain equilibrium points, which is the set number of occupied patches the metapopulation can sustain (Riegl & Glynn, 2020). For example, the Levins model has an equilibrium point at the carrying capacity mentioned above. The propagule rain model displays a linear colonization function, unlike the Levins model. This model assumes the surrounding seawater of a patch is consistently saturated with propagules or the gametes needed to recolonize. When the number of patches is low enough, the probability of rescue is incredibly high. This model also has one stable equilibrium point (Riegl & Glynn, 2020). On the other hand, the core-satellite model assumes that larger patches will consistently replenish any destroyed smaller patches around them. Under this assumption, the colonization rate is either always above the extinction rate or vice versa. Therefore, this model's equilibrium points are at either the maximum number of patches possible or none! If the probability of rescue does not vary linearly or follows some other unknown relation, more complex equilibrium points, including unstable ones, can exist (Riegl & Glynn, 2020). These models are graphically depicted in Figure 12 below.

Fig. 12. A) Each coral colony can be considered a patch, which can colonize another patch that is not occupied (c). Each patch also has a chance to go “extinct” (e) and empty the patch for future colonization. B) The Levins model, where red represents the probability of colonization, and blue represents the same for extinction. Notice the single equilibrium point that shifts depending on the extinction rate. C) The propagule rain model, which instead has an equilibrium point that depends on the colonization rate. D) The core-satellite hypothesis assumes the colonization rate is always above the extinction rate. The distance of the two equilibrium points depends on the values of c and e. E) If the rescue effect varies nonlinearly depending on extraneous variables, more complicated equilibrium points can exist that can be unstable (Riegl & Glynn, 2020).
Conclusion
From the fundamental fractal structure of each polyp’s exoskeleton to the population dynamics that define the recovery of entire reef biomes, the mathematical complexity of the reef is essential to the stability and survival of the biome. The very fundamental unit of the coral, the polyp, excretes an aragonite exoskeleton that is uniquely fractal. The skeleton also exhibits hyperbolic geometry with negative curvature. Both factors act as a design solution to lower nutrient concentrations, as fractality and negative curvature increase the rate of nutrient absorption by increasing the colony’s surface area. Coral polyps also exhibit radial symmetry, which varies between Hexacorallians and Octocorallians. The origin of this pattern can be traced to Paleozoic corals, which utilized this pattern to sustain harsher oceanic conditions.
The entire survival of the reef depends on the fecundity of the coral population, which persists under synchronized spawning. Integrative population models can accurately model the future growth or decline of a reef depending on the fecundity of the population. A key property to the success of the colony lies in its size, with larger colony sizes conferring a competitive advantage. As humanity continues to overwhelm the biome, recovery and rehabilitation have been found to occur naturally if each reef falls under a metapopulation.
Understanding the geometry, symmetry, and dynamics of the reef is crucial for developing effective conservation strategies. By analyzing their reproductive strategies, geometric development, and metapopulation characteristics, ecologists can design targeted intervention strategies that harness the coral’s natural resilience. As our world continues to grow more and more hostile to the reefs, the coral’s best chance at survival lies in leveraging their mathematical complexity for conservation.
References
References
Animal Characterization Based on Body Symmetry. LibreTexts Biology. https://bio.libretexts.org/Bookshelves/Introductory_and_General_Biology/General_Biology_(Boundless)/27%3A_Introduction_to_Animal_Diversity/27.02%3A_Features_Used_to_Classify_Animals/27.2A%3A_Animal_Characterization_Based_on_Body_Symmetry
Coral Polyp Anatomy. Coral Disease & Health Consortium. https://cdhc.noaa.gov/coral-biology/coral-biology/
Coral Reefs. Endangered Species International. https://www.endangeredspeciesinternational.org/coralreefs.html
Coral Skeleton. Coral Disease Health & Consortium. https://cdhc.noaa.gov/coral-biology/coral-skeleton/
End- Permian Extinction. The University of Oklahoma: Sam Noble Museum. https://samnoblemuseum.ou.edu/understanding-extinction/mass-extinctions/end-permian-extinction/
Fabricius, K. (2024). Soft corals of the Great Barrier Reef. Australian Institue of Marine Science. https://eatlas.org.au/content/soft-corals-great-barrier-reef
Fractal geometry. Pardesco. (n.d.-a). https://pardesco.com/blogs/news/fractal-geometry?srsltid=AfmBOopbPBbk6IdGq8R1HLlMBscslMXA3h3ytmF1snYTaOONxMB77pUz
Hurley, S. (2023, December 4). Is the Universe Curved?. Explaining Science. https://explainingscience.org/2023/12/01/is-the-universe-curved/
Hoffman, H. J. The Permian extinction - when life nearly came to an end. National Geographic. https://www.nationalgeographic.com/science/article/permian-extinction
Keymer, J., Marquet, P., Velasco-Hernández, J., & Levin, S. (2000). Extinction thresholds and metapopulation persistence in dynamic landscapes. https://www.semanticscholar.org/paper/Extinction-Thresholds-and-Metapop…
Levins, R. (1969). Some Demographic and Genetic Consequences of Environmental Heterogeneity for Biological Control. Bulletin of the Entomological Society of America, 15(3), 237–240. https://doi.org/10.1093/besa/15.3.237
Malakhov, V. (2016). Symmetry and the tentacular apparatus in Cnidaria. Russian Journal of Marine Biology, 42, 287-298. https://doi.org/10.1134/S1063074016040064
Martin-Garin, B., Lathuilière, B., Verrecchia, E. P., & Geister, J. (2007c). Use of fractal dimensions to quantify coral shape. Coral Reefs, 26(3), 541–550. https://doi.org/10.1007/s00338-007-0256-4
Mistr, S. and Bercovici, D. (2003) A Theoretical Model of Pattern Formation in Coral Reefs. Ecosystems, 6, 61-74.
http://dx.doi.org/10.1007/s10021-002-0199-0
Merow, C., Dahlgren, J.P., Metcalf, C.J.E., Childs, D.Z., Evans, M.E.K., Jongejans, E., Record, S., Rees, M., Salguero-Gómez, R. and McMahon, S.M. (2014), Advancing population ecology with integral projection models: a practical guide. Methods Ecol Evol, 5: 99-110. https://doi.org/10.1111/2041-210X.12146
More details about corals. Louisiana University. https://userweb.ucs.louisiana.edu/~scf4101/Bambooweb/MoreAboutCoral.htm
Ospanova, N. (2023). About Symmetry of Paleozoic Corals and Its Relation with the Gravity. The National Academy of Sciences of Tajikstan, Institue of Geology, Earthquake Engineering and Seismology, 5(08), 256-259. https://www.ss-pub.org/aeer/about-symmetry-of-paleozoic-corals-and-its-relation-with-the-gravity/
"Paleozoic." Youth and Education in Science. https://www.usgs.gov/youth-and-education-in-science/paleozoic (accessed.
Riegl, B. M., & Glynn, P. W. (2020). Population dynamics of the reef crisis: Consequences of the growing human population. Advances in Marine Biology, 87(1), 1–30. https://doi.org/10.1016/bs.amb.2020.07.004
Sakai Y, Yamamoto HH, Maruyama S. Long-term aquarium records delineate the synchronized spawning strategy of Acropora corals. Royal Soc Open Sci. 2024;11(5):240183. doi: 10.1098/rsos.240183
Shlesinger T, van Woesik R. Different population trajectories of two reef-building corals with similar life-history traits. J Anim Ecol. 2021 May;90(5):1379-1389. doi: 10.1111/1365-2656.13463. Epub 2021 Mar 17. PMID: 33666226; PMCID: PMC8252767. Zaczyński, B. (2023, October 21). Draw the Mandelbrot set in Python. Real Python. https://realpython.com/mandelbrot-set-python/