
Table of Contents
Keywords: Algorithms, foraging, pheromones, cooperative transport, eusocial, clustering
Abstract
Ants are eusocial creatures that showcase collective intelligence by solving complex problems through simple local interactions. Their behaviors—foraging, clustering, cooperative transport, and task allocation—have inspired powerful algorithms for optimizing and problem-solving in decentralized systems. Using pheromonal communication and probabilistic decision-making, ants efficiently distribute tasks and coordinate activities without central control. Models of behaviors like brood sorting and cooperative transport reveal these natural strategies' remarkable scalability and adaptability and provide valuable insights for fields like swarm robotics and dynamic systems. Recent innovations in ant-inspired algorithms, including memory-based enhancements and pheromone-guided techniques, underscore the transformative potential of bio-inspired solutions in solving computational and organizational challenges.
Introduction
Ants must collaborate to accomplish large-scale tasks like acquiring food for the colony, building nests, transporting prey and sorting brood. An explanation of how ants communicate is crucial to understand the collective intelligence in ants. To perform coordinated activities, ants use stigmergy which is a form of indirect communication through the environment. This is primarily done with the use of chemical substances that ants produce and secrete from their glands, called pheromones (Morgan, 2009). For instance, when an ant finds food, it deposits pheromones along its return path to guide other local ants to the source and these local ants also deposit pheromones (Fig. 1). This positive feedback loop helps the colony identify optimal foraging routes (Thienen et al., 2014).

Fig. 1. A model of foraging ants with two task-dependent pheromones. Communication between the ants in the model is mediated through changes to the environment by deposition of two attractive pheromones. When ants are searching for food, they deposit pheromone A and follow pheromone B. Those searching for the nest deposit B and follow A (Malíčková et al., 2015).
This system allows ant colonies to operate without centralized control meaning that they rely on local interactions among individuals to achieve coordinated outcomes (Pratt, 2010). The collective act of foraging is crucial for the colony’s survival. Through local interactions, ants can cover larger areas, communicate food locations and optimize their paths, all while reducing the time and energy spent.
Furthermore, in this collective behavior, ants need to make a lot of decisions. Individual decision-making is based on probabilistic assessments of local cues during foraging and transport. Additionally, ants organize their brood by probabilistically picking up and dropping items based on local similarity. This combination of stigmergy and probabilistic decision-making of ants has inspired various computational models and algorithms which will be described throughout this paper.
Computer Simulations of Ant Foraging Behavior
Computer simulations modeled by real ant behavior can be used to analyze and understand the algorithms ants use to forage. Ant navigation through complex foraging trail networks can be simplified and generalized into a binary tree structure model, as seen in Fig. 2. Such a foraging pattern has been observed in species like the seed harvester ant, Messor barbarus, and certain army ants.

Fig. 2. Binary tree model of path choice. At each branching point (small circle), each ant can choose between two possible paths. The number of branching levels is called the "altitude" of the tree. In this example, the tree has an altitude of 3, resulting in 8 potential foraging sites.
Within the binary tree, any branching point with two possible path choices starts with an equal bias (50-50%) for each path. This means that, at this point, an ant at the branch point is equally likely to select one or the other. However, ants can update their bias to optimize their foraging strategies. When returning from one path, ants deposit positive or negative feedback pheromones to promote or discourage other ants from behaving similarly, depending on the success of their forage. As incoming nestmates arrive at the branch point, they can detect these pheromones and act accordingly. This recruitment behavior updates the bias and determines the probability of another ant taking that path. Over time, accumulated positive and negative feedback allows one path to become the dominant choice. If the bias value of any path reaches 100% or 0%, it is then considered “fixed,” so all ants passing that branch point will take the fixed route (Stickland, 1995). Here, it is essential to note that, using this model, an individual ant's memory and previous choices do not influence their selection paths – their choices are purely probabilistic.
This feedback mechanism closely mirrors backpropagation algorithms used to train neural networks. As ants use pheromones to update bias, neural networks backpropagate errors in predictions to adjust the weights of connections between neurons, either strengthening or weaking them depending on the feedback signal. Similarly, to how pheromone concentrations begin favoring particular paths over time, weight adjustments in a neural network start to improve their predictive accuracy over time (Elliott, 2001). Both of these systems demonstrate how iterative feedback mechanisms are useful for optimizing behavior for accuracy and efficiency.
Influencing Factors in Ant Decision-making in the Context of Foraging
While more abundant food sources result in positive pheromone updates, other factors also impact the bias toward a particular path and, subsequently, foraging efficiency. This includes an ant's " influence" (I) on their nestmates and nest departure-return rates (R).
Set by the parameter I in computer simulations, the influence on nestmates is dictated by the effect of pheromones deposited per returning ant. A higher influence factor implies that ants have more impact on their nestmates' decisions. In the simulation, if every returning ant deposits positive pheromones, then with an influence factor of I = 5%, the first ant to return from a newly explored path will shift the bias from 50%-50% to 55%-45% in favor of the path it took (Stickland, 1995).
Regarding foraging frequency, nest departure rates in the algorithm simulation are set by R, which denotes the time interval between which ants depart from their nest to forage. A lower R value implies ants leave the nest more frequently. With this, ants that have left the nest move between branch points in one period of t (i.e. from t to t + 1). So, for a tree with an altitude value of a, it takes each ant Δt = 2a time to leave and return to the nest.
In real life, not all path lengths to food sources are equivalent in distance. The species Linepithema humile and Lasius niger have been observed prioritizing shorter path lengths to food sources. Since lesser travel distances accelerate return rates, “positive” pheromones are deposited on the trail more frequently, quickly increasing bias over such paths. As demonstrated in Fig. 3, this constantly updating algorithm optimizes foraging efficiency by ensuring ants acquire sustenance consistently and quickly (Stickland, 1995).

Fig. 3. Simulation results of ants foraging on a network of pheromone trails. When ants’ choices at branching points include bias, foraging efficiency increases threefold compared to when there is no directional bias (Garnier, 2011).
It is vital that ants optimize their foraging behavior based on multiple factors (i.e. one specific factor does not single handedly “dictate” decision-making). For example, when influence (I) over nestmates is high and departure-return rates are low, pathways can be fixed by fewer ants, thereby leading to quicker colony decisions, as seen in Fig. 4 (Stickland, 1995).

Fig. 4. The impact of the influence factor (I) and the ants' departure rate (R) on the time to establish a fixed path from the nest to a foraging site. Here, graphs (a) and (b) respectively represent two influence factor values I=10% and I=1%. Different values of R are represented by distinct symbols: R = 1 by circles, R = 5 by squares, R = 10 by triangles, and R = 20 by inverted triangles.
The downside of this, however, is demonstrated through computer simulations shown in Fig. 5, where swift decisions lead to the severance of unexplored and possibly fruitful search sites. On the contrary, while yielding slow decision-making, low influence values and high foraging frequency lead to greater “tree” exploration.

Fig. 5. The impact of the influence factor (I) and the ants' departure rate (R) on the percentage exploration of a simulated tree of altitude a=7 (i.e. 128 possible foraging sites) (Stickland, 1995).
Limitations of Computer Simulations
In the real world, there are countless conditions like changing food availability or varying environmental conditions which will alter ant foraging behavior in ways that are not predictable by any computer simulation. Additionally, computer simulations do not consider how ants might change their decision-making processes when encountering hindrances like predators or unfamiliar terrain. Nevertheless, while simplifying the real-world dynamics that affect ant behavior, models like the one discussed here highlight foundational aspects of the algorithmic behavior in ants that enable optimized efficiency in foraging.
Algorithms Inspired by Ants’ Cooperative Transport
Social insect societies like ants exhibit decentralized colony behavior and demonstrate cooperative prey retrieval that allows them to transport objects much larger and heavier than a single ant could carry (Kube & al., 2000; Alkilabi et al., 2017). Ants use stigmergy which is the coordination of activities through indirect interactions. For this reason, in cooperative transport the movement by one ant is likely to modify the stimuli perceived by the other group members, which produces orientational or positional changes in these ants. This indirect coordination through the environment has been used to develop algorithms used in swarm robotics for coordinating distributed building behavior and foraging tasks by multirobot systems.
Quantifying the Relationship between Group Size and Transport Efficiency
When an ant finds prey, it tries to move it on its own, and if successful, it carries the item back to the nest. However, when an ant encounters resistance while trying to move prey, it stimulates the recruitment of other ants. In some species, if a group of ants is still unable to move the prey, specialized workers with large mandibles may be recruited to cut the prey into smaller pieces. Recruitment stops once the group can successfully carry the prey (Kube & Bonabeau, 2000). A study found that in Pheidologeton diversus, the number of ants (N) participating in transport scales with the burden weight (W) according to the relationship: N ∝ W. Similarly, another study observed that the total weight of the transporting ants (Wa) is proportional to the weight of the transported item (Wi): Wa ∝ Wi (Kube & al., 2000). Based on this information, they concluded that larger groups generally lead to higher carrying capacity. However there seems to be an optimal group size for maximizing transport efficiency because they observed that the transport velocity decreased with larger group sizes. The efficiency per ant is measured by the product of burden weight (W) and transport velocity (ν) divided by number of carriers (N), which increases with group size up to a certain point.

For instance, in Pheidologeton diversus, maximum transport efficiency was observed with groups of 8-10 ants, and it decreases significantly for large group sizes of over 12 carriers (Kube & Bonabeau, 2000). Observing how these factors can influence transport efficiency, swarm-based robotics use algorithms inspired by the ants’ cooperative transport. One team studied how ant mechanisms could be used to regulate a group of robots pushing a box (shown in Fig. 6).

Fig. 6. The lab environment used to test a group of robots moving a round box between two goal positions.
The results of this study (shown in Fig. 7) suggest that box-pushing may be more or less efficient depending on the number of robots required to complete the task (Kube & Bonabeau , 2000).

Fig. 7. The mean execution time of moving a 42 × 42 cm2 box 2.5 m towards a goal position as a function of the number of robots. For each plot the number of trials as well as the minimum and maximum run times are indicated. A box side is approximately twice the robot’s diameter and increasing the number of robots increases robot interference as they compete for the limited space available (Kube & Bonabeau, 2000).
Analyzing Transport Trajectories Efficiency with Sinuosity
Studies of real ants have used the sinuosity (S) of objects’ trajectories to evaluate the efficiency of cooperative transport. Sinuosity is defined as the ratio of the object's path length traveled by the object (P) to the straight-line distance between its starting and ending position (ΔOpos). Both P and ΔOpos are measured with reference to the object’s center of mass (Alkilabi et al., 2017).

Higher sinuosity values indicate less efficient transport. This is because very sinuous trajectories are generated by frequent changes in transport directions which is generally the result of poor coordination between the ants while pushing the object. Conversely, lower sinuosity values approaching the minimum value of 1 imply a more direct path and a higher level of coordination among the transporting ants. This usually means that the ants made a consensus on the direction of transport quickly and maintained coordination during the entire duration of the transport (Alkilabi et al., 2017).
This same measurement was used to analyze the performance of a group of e-puck robots programmed to transport an object. Using Equation 2, the study observed how the sinuosity of the robot increased in a few cases (shown in Fig. 8). The mass and length of the object being transported influenced the sinuosity of the path. They saw that heavier and longer objects tend to result in higher sinuosity. Additionally, rotational movements of the object, more frequent with heavier objects, contribute to increased sinuosity. In general, sinuosity provides valuable insights into the relationship between object characteristics and the efficiency of group transport in robot swarms (Alkilabi et al., 2017).

Fig. 8. The graph shows the results of four tests conducted with a single physical robot. Each box refers to the number of repositioning events on a set of ten trials that last for 60 seconds. The experimental conditions L (light), H (heavy), S (short), and R (long) refer to trials with different types of objects (Alkilabi et al., 2017).
Probabilistic Decision-making in Cooperative Transport
Ants use pheromones for coordination during cooperative transport. Their decisions are influenced by local cues and the actions of their nestmates. A key factor in their decision-making process is the resistance encountered when attempting to move prey. The decision to transition from solitary to group transport is therefore probabilistic and based on the perceived difficulty of the task and resistance encountered. Moreover, when transport stalls are due to opposing forces or obstacles, ants engage in realigning and repositioning behaviors. The frequency of these adjustments increases over time and reflects a probabilistic response to the lack of progress (De Rango et al., 2017).
Researchers have developed probabilistic routing tables to guide robots in a swarm towards target locations. Instead of having fixed paths, probabilistic routing tables maintain a probability distribution for choosing the next hop towards a destination. This distribution is updated based on the "pheromone" values, which represent the desirability of different paths. Each robot maintains a routing table that contains information about the possible path to reach the target. The probability (p) of a robot (k) moving from its current cell (ctk) to a neighboring cell (c) is calculated as follows:
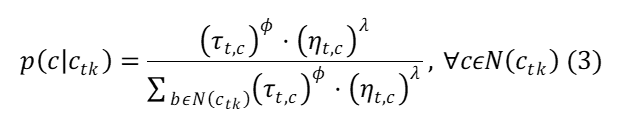
Where p(c|ctk) is the probability of robot k moving from cell ctk to cell c; τt,c is the total number of pheromones in cell c; ηt,c is the heuristic variable to prevent robots from getting trapped; φ and λ are constants that balance the influence of pheromone levels and the heuristic variable; and N(ctk) is the set of accessible neighboring cells to the robot's current cell .
This formula captures the probabilistic nature of a robot’s decision-making process. It is more likely to move to cells with higher pheromone levels (shown in Fig. 9), but the heuristic variable and the constants ϕ and λ introduce variability and prevent deterministic behavior. The probabilistic routing tables are used to guide robots in a swarm toward a target, which is the reason why these tables are also called pheromone tables (De Rango et al., 2017).

Fig. 9. Robots during exploration “spray” a pheromone that propagates in the neighbor’s cells. The quantity in each cell depends on the distance. The cell in which the robots are moving has a higher quantity and decreases with distance (De Rango et al., 2017).
Moreover, to further mimic ants, robots are programmed to use probabilistic decision-making mechanisms based on sensory feedback. In a study, robots are equipped with optic-flow sensors that allow them to detect changes in their position relative to the environment. This feedback helps them adjust their pushing forces and coordinate with other robots to move the object towards a goal. If the object moves, the robot is less likely to reposition itself. However, if the object remains stationary or moves in an unexpected direction, the robot will reposition itself more frequently to find a more effective pushing point. This probabilistic adaptation to the object's behavior allows the robots to collectively find directions of transport and sustain the transport even in the absence of direct communication (De Rango et al., 2017).
Algorithms Inspired by Division of Labor in Ants
Division of Tasks in Ants: Dynamic Task Allocation
The division of tasks among eusocial insects is very important for the ecological success of their colony, because it allows individuals to specialize in specific tasks and carry them out simultaneously with a similar efficiency. Depending on the species, common tasks among ants include gathering food (foraging), tending to the offspring (brood care), and protecting the nest from invaders or parasites (defense) (Ware & Wilson, 2022).
Task performance in social insects differs from the classical division of labor seen in hierarchical systems—such as packs or human teams—where efficiency is often maximized by having individuals specialize in a single task and avoid switching roles. Instead, ants follow a system called dynamic (or flexible) task allocation, which means that the group dynamically adjusts their roles based on current needs, shifting as demand changes for some specific tasks (a decentralized approach to labor). So, one role is not exclusive to a section of the colony. For example, a worker forager can also take tasks like patrolling depending on certain cues. However, this does not mean that every ant can perform every task (Pinter-Wollman et al., 2012). There is a certain division in the system. For example, physiological differences among individuals’ ants define their roles. Worker ants are typically sterile and lack the reproductive capabilities of the queen, whose primary function is to produce offspring.
Task Response Threshold
The way roles are distributed is through the task response threshold, which is a concept based on environmental cues. If these cues exceed the worker's threshold, they will perform the task until the cues no longer meet the threshold. Individuals who have the lowest thresholds for a task at any given time perform it, thus ensuring that there are always some workers performing every task (Pinter-Wollman et al., 2012). Individuals vary in thresholds, and those that happen to have lower thresholds are more likely to become “specialists” for that task, implying that some individuals have a certain preference for a particular task without being restricted to it. Interestingly, when the demand for a role in the colony changes, the colony can recruit more workers for that task by lowering the response thresholds through pheromone signals or social interaction, such as physical contact.
Temporal Polyethism
A common feature of ants’ allocation of tasks is that, on average, the eldest ants tend to perform the most dangerous tasks, such as foraging and colony defense. In contrast, the youngest ants typically engage in brood care and nest maintenance (Tofts, 1993). This age-based division of labor is known as temporal polyethism, where tasks are distributed among workers according to their age—a pattern clearly illustrated in Fig. 10. Interestingly, this feature is still consistent with the dynamic, complex task allocation in the ants colony. It has been suggested that temporal polyethism arises from intra-colony competition: younger workers compete for access to the brood area, effectively displacing older workers, who then shift toward riskier roles such as foraging (Robinson et al., 1994).

Fig. 10. The average age of worker ants performing 4 different tasks, all related to foraging, plotted against time in two different instances (a and b), showing the formation of a tasks-based age spectrum (Tofts, 1993).
Model Illustrating Task Organization in Colonies
The system used by ants and other eusocial insects to allocate different roles is very complex and well-organized. It has advantages over hierarchical systems often used by other species, such as being adjustable as the group grows, being resilient to environmental changes, and allowing individuals to perform simple tasks that overall show a complex behavior (Kang & Theraulaz, 2016).
To understand this system, it is possible to use a mathematical model that illustrates how ant colonies distribute workers to different tasks. The model, proposed by Yun Kang in the Bulletin of Mathematical Biology (Kang & Theraulaz, 2016) and simplified below, highlights how colony size, social collaboration, and temporal polyethism influence task organization in ants.

Equation 4 represents the colony size, where N is the colony size, Ti is the number of ants working on a certain task and m represents the number of tasks (Kang & Theraulaz, 2016).
One key implication of this equation is that the colony size is extremely important to the organization of ants. Larger colony size (N) allows more workers to be allocated to tasks (Ti) and thus there are more individuals performing each task (i). Colony size is positively related to both reproductive and non-reproductive roles
In this model, task allocation of the colony at time (t) is represented by:


Equation 6 is the general equation for the change of number of ant workers available for a task. N' is the rate of change of total number of workers available; N is the colony size; r is the reproduction rate of queens; n is a constant; s denotes the nonlinear effect of collaboration; Tj is the number of workers performing task j; μj is the death rate, could also be seen as the rate at which workers stop performing a task (Kang & Theraulaz, 2016).
This equation is based on three main ideas. First, each worker has a different genetically determined response threshold for a specific task. Second, a worker’s interactions with others influence their task performance, meaning that an ant is more likely to engage in a task when another is performing it. Third, each task has its own demand that changes over time, depending on external environmental factors (Ferguson-Gow et al., 2014).
Among other things, the general equation implies two important details. First, is that when the colony size N is large, there is an increase in workers being able to perform a task but eventually reaches a limit because of b+Ns . Second, the collaboration factor (S) impacts the change of number of available workers, thus also influencing the allocation dynamic. The factors are always positive and correlated to the number of tasks (m). For instance, when m = 2, S = 2, since the more tasks there are, the more possibilities of collaboration between individuals. This shows the social influence of task allocation; if one worker sees another ant performing a task, it is more likely to join.
Temporal Polyethism Model
Considering that temporal polyethism is difficult, since it requires a method to know an ant's age other than allowing them to die. Certain assumptions must then be made to be able to model this mechanism (Tofts, 1993).
For this model, it is assumed that newborn workers are born in the task status i=1, which would be brood care, paired with the rate rN2b+N2. Then, the rest of the older ants (task groups i>2) is combined with a maturation rate: i-1
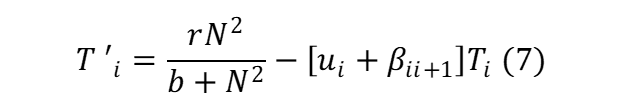
Equation 7 is a simplified version of the Task Organization Model with temporal polyethism by Yun Kang, where Ti is the number of workers performing task i, and the colony size remains N (Kang & Theraulaz, 2016).
This model for temporal polyethism shows how beneficial it is for ants to allocate tasks based on age. It brings several advantages, such as reducing colony vulnerability by allowing older and potentially stronger ants to take riskier roles.
Modeling task allocation systems in general allows the exploration of how colonies balance between growth, meaning investing resources in tasks that support reproduction, and survival, allocating more to defense and foraging. This balance of roles can be applied in many other systems that require productivity, resilience, and adaptability.
Algorithm Inspired by Brood Sorting in Ants
One of the critical features of eusocial insects is the care of broods by young adults (Franks & Sendova-Franks, 1992). When clustering, ants gather items together to form heaps. One example of the phenomenon is the species Pheidole pallidula, which clusters corpses to create a cemetery. When sorting, ants will distinguish the different types of objects and arrange them with specific properties spatially. Leptothorax unifasciatus is another species that performs this activity. Larvae are arranged according to sizes in the nests of Leptothorax unifasciatus (Handl et al., 2006). These ants compactly cluster their eggs and smaller larvae at the center of the nest brood area and the larger larvae at the periphery of the brood cluster to optimize thermal regulation, resource allocation, and protection, demonstrating emergent self-organizing behaviors (Dorigo et al., 2006).
In ant colonies, brood sorting is a crucial behavior that helps maintain the efficiency and health of the colony. Ants optimize the distribution of resources and specialized care within the nest. Each ant performs actions based on local cues, leading to an organized arrangement where the youngest and most vulnerable brood receives attention. This behavior ensures that resources like food and labor are allocated effectively, supporting colony growth and resilience (Hölldobler & Wilson, 1990).
Basic Principle and Core Mechanisms
Ant-based clustering and sorting, a distributed sorting algorithm, is a local distributed heuristic that operates on the principle of simplicity. As Handl, Knowles, and Dorigo describe, this algorithm is based on simple, individual rules followed by each ant, leading to complex, organized structures without any central control (Handl et al., 2004).
Ant-based clustering operates on a unique principle, distinct from traditional algorithms such as k-means or agglomerative clustering. Instead of gradually constructing or refining an explicit representation of a data set’s partitioning, ant-based clustering generates the partitioning implicitly. The final spatial distribution of the data contains all information on the number of clusters and the cluster memberships of individual data items. This outcome is achieved without explicitly defining an optimization criterion or global goal. It emerges self-organized from local actions and positive feedback only (Handl et al., 2004).
The basic model uses ant-like robots, which only move randomly. The probability of ant-like robots picking up an object depends on how isolated the object is when they come across an object. How isolated an object is from others is proportional to how similar objects are encountered: the fewer objects, the greater the probability. While carrying an object, the probability of dropping it increases if there are many similar objects in the vicinity (Deneubourg et al., 1991). These two rules work together to reach maximum efficiency.
Initially, scattered objects are picked up by ants and dropped near similar ones, forming small clusters. These clusters grow through a positive feedback loop. Larger clusters become increasingly attractive to carriers, absorbing isolated objects and smaller clusters. As clusters of the same type expand, they crowd out dissimilar objects, isolating them and facilitating their relocation (Fig. 11). This process leads to emergent sorting without central control, highlighting the self-organizing nature of the algorithm.

Fig. 11. Layouts of elements on a 52x52 grid. Different symbols represent elements sampled from different distributions. A (left): Initial layout. b (right): Layout after 50 cycles using a population of basic clustering agents (Lumer & Faieta, 1994).
A new frame is created to apply the mechanism. The environment is set into a square network of points. At time zero, several ant-like robots and objects of type A and B are placed randomly. Only one entity is allowed per point. At each time point, the ant-like robots move in 4 directions, and they cannot go further if the destination is outside the grid or the destination point has been occupied. The probability of picking up can be calculated as:

where f is an estimation of the fraction of nearby points occupied by objects of the same type, and k+ is a constant (Deneubourg et al., 1991).
If an ant has picked up an object, then at each step, it finds itself at an unoccupied point, and it decides whether to put the object down. The probability can function as follows:

where f is as before and k- is a constant.
In 1994, Lumer and Faieta improved the function of estimation of the fraction of nearby points into a neighborhood function:

where i is a given grid position, δ(i,j) ∈ [0,1] is a dissimilarity function defined between points in data space, α ∈ [0,1] is a data-dependent scaling parameter, and σ2 is the size of the local neighborhood L (typically σ2 ∈ {9,25}).
Algorithm Extensions and Developments
The basic ant-based clustering algorithm has significantly improved since its initial formulation. Researchers have enhanced the original model by incorporating additional biological insights from ant colonies. For instance, Martin et al. (Martin et al., 2002) introduced a short-term memory mechanism inspired by how real ants remember recently visited locations, reducing repeated visits to the same areas and improving clustering efficiency. This modification led to faster convergence rates while maintaining the algorithm's ability to form distinct clusters. Another notable enhancement came from Chen et al. (Chen et al., 2004), who implemented a pheromone-based attraction mechanism inspired by ant foraging behavior, where virtual pheromone trails guide clustering agents toward promising regions of the solution space, enhancing the algorithm’s exploratory capabilities and mimicking the decentralized decision-making observed in natural ant colonies."
These bio-inspired modifications demonstrate how continued observation of natural ant behavior can inform algorithmic improvements. The success of these enhancements supports the value of maintaining close connections between biological observations and algorithmic development (Handl & Meyer, 2007). Recent studies have shown that incorporating multiple aspects of ant behaviors such as their tendency to follow environmental gradients and their ability to assess local density patterns—can lead to more robust clustering solutions (Zhang & Wu, 2019). As our understanding of ant colony dynamics continues to grow, new insights may inspire further refinement to these algorithms, potentially addressing current limitations in convergence speed and parameter sensitivity.
Conclusion
Acquiring high-quality food at fast rates is crucial for the survival of ant colonies – colonies would starve otherwise. As ants live in a wide range of complex environments, with many obstacles and other precarious factors, it is often difficult to find food sources and develop optimal paths to them. To address this, ants have developed an iterative feedback system of pheromone deposition and detection to communicate and coordinate their foraging activity. Through decentralized decision-making and prioritizing quality and proximity, this mechanism can be modelled as an algorithm to demonstrate how ants locate new food sources swiftly and consistently, ensuring the colony’s survival.
Without organized labor, colonies could not respond dynamically to environmental changes or transport food and would be especially vulnerable to predators. Through complex task allocation, influenced by task response thresholds and temporal polyethism, ants can coordinate responsibilities, dynamically switching roles as needed. For instance, younger workers may focus on brood care, while older ants take on riskier tasks like foraging. This flexibility enables colonies to optimize their workforce and respond to environmental demands without rigid hierarchies. This behavior can be understood by modelling scaling relationships between group size and burden weight, efficient metrics like transport velocity and sinuosity and probabilistic decision-making.
Ultimately, ants' survival depends on their ability to adapt to complex, resource-limited, and unpredictable environments. With their feedback system and decentralized decision-making, ants efficiently coordinate foraging, brood care, nest defense, and many other types of labor. Only through effective algorithmic communication and coordination do ant colonies remain dynamic and resilient.
References
References
Alkilabi, M. H. M., Narayan, A., & Tuci, E. (2017). Cooperative object transport with a swarm of e-puck robots: robustness and scalability of evolved collective strategies. Swarm Intelligence, 11(3–4), 185–209. https://doi.org/10.1007/s11721-017-0135-8
Chen, L., Xu, X.-H., & Chen, Y.-X. (2004). An adaptive ant colony clustering algorithm. Proceedings of 2004 International Conference on Machine Learning and Cybernetics (IEEE Cat. No.04EX826), 4, 1387–1392. https://doi.org/10.1109/icmlc.2004.1381990
Czaczkes, T. J., Grüter, C., Ellis, L., Wood, E., & Ratnieks, F. L. W. (2012). Ant foraging on complex trails: Route learning and the role of trail pheromones in Lasius niger. Journal of Experimental Biology, jeb.076570. https://doi.org/10.1242/jeb.076570
David Morgan, E. (2009). Trail pheromones of ants. Physiological Entomology, 34(1), 1–17. https://doi.org/10.1111/j.1365-3032.2008.00658.x
De Rango, F., Palmieri, N., Yang, X., & Marano, S. (2017). Swarm robotics in wireless distributed protocol design for coordinating robots involved in cooperative tasks. Soft Computing, 22(13), 4251–4266. https://doi.org/10.1007/s00500-017-2819-9
Deneubourg, J. L., Goss, S., Franks, N., Sendova-Franks, A., Detrain, C., & Chrétien, L. (1991). The dynamics of collective sorting: Robot-like ants and Ant-like robots. From Animals to Animats, 356–364. https://doi.org/10.7551/mitpress/3115.003.0048
Dorigo, M., Birattari, M., & Stutzle, T. (2006). Ant colony optimization. IEEE Computational Intelligence Magazine, 1(4), 28–39. https://doi.org/10.1109/mci.2006.329691
Elliott, S. J. (2001). Active Control of Nonlinear Systems. In Signal Processing for Active Control (pp. 367–409). Elsevier. https://doi.org/10.1016/B978-012237085-4/50010-7
Ferguson-Gow, H., Sumner, S., Bourke, A. F. G., & Jones, K. E. (2014). Colony size predicts division of labour in attine ants. Proceedings of the Royal Society B: Biological Sciences, 281(1793), 20141411. https://doi.org/10.1098/rspb.2014.1411
Franks, N. R., & Sendova-Franks, A. B. (1992). Brood sorting by ants: Distributing the workload over the work-surface. Behavioral Ecology and Sociobiology, 30(2). https://doi.org/10.1007/bf00173947
Garnier, S. (2011). From Ants to Robots and Back: How Robotics Can Contribute to the Study of Collective Animal Behavior. In Y. Meng & Y. Jin (Eds.), Bio-Inspired Self-Organizing Robotic Systems (Vol. 355, pp. 105–120). Springer Berlin Heidelberg. https://doi.org/10.1007/978-3-642-20760-0_5
Handl, J., & Meyer, B. (2007). Ant-based and swarm-based clustering. Swarm Intelligence, 1(2), 95–113. https://doi.org/10.1007/s11721-007-0008-7
Handl, J., Knowles, J., & Dorigo, M. (2004). Strategies for the increased robustness of ant-based clustering. Lecture Notes in Computer Science, 90–104. https://doi.org/10.1007/978-3-540-24701-2_7
Handl, J., Knowles, J., & Dorigo, M. (2006). ANT-based clustering and topographic mapping. Artificial Life, 12(1), 35–62. https://doi.org/10.1162/106454606775186400
Hölldobler, B., & Wilson, E. O. (1990). The ants. Springer-Verlag.
Kang, Y., & Theraulaz, G. (2016). Dynamical Models of Task Organization in Social Insect Colonies. Bulletin of Mathematical Biology, 78(5), 879–915. https://doi.org/10.1007/s11538-016-0165-1
Kube, C., & Bonabeau, E. (2000). Cooperative transport by ants and robots. Robotics and Autonomous Systems, 30(1–2), 85–101. https://doi.org/10.1016/s0921-8890(99)00066-4
Lumer, E. D., & Faieta, B. (1994). Diversity and adaptation in populations of clustering ants. From Animals to Animats 3, 501–508. https://doi.org/10.7551/mitpress/3117.003.0071
Malíčková, M., Yates, C., & Boďová, K. (2015). A stochastic model of ant trail following with two pheromones. arXiv (Cornell University). https://doi.org/10.48550/arxiv.1508.06816
Martin, M., Chopard, B., & Albuquerque, P. (2002). Formation of an ant cemetery: Swarm intelligence or statistical accident? Future Generation Computer Systems, 18(7), 951–959. https://doi.org/10.1016/s0167-739x(02)00074-2
Pinter-Wollman, N., Hubler, J., Holley, J.-A., Franks, N. R., & Dornhaus, A. (2012). How is activity distributed among and within tasks in Temnothorax ants? Behavioral Ecology and Sociobiology, 66(10), 1407–1420. https://doi.org/10.1007/s00265-012-1396-2
Pratt, S. (2010). Collective intelligence. In Elsevier eBooks (pp. 303–309). https://doi.org/10.1016/b978-0-08-045337-8.00352-1
Robinson, G. E., Page, R. E., & Huang, Z.-Y. . (1994). Temporal polyethism in social insects is a developmental process. Animal Behaviour, 48(2), 467–469. https://doi.org/10.1006/anbe.1994.1260
Stickland, T. (1995). Complex trails and simple algorithms in ant foraging. Proceedings of the Royal Society of London. Series B: Biological Sciences, 260(1357), 53–58. https://doi.org/10.1098/rspb.1995.0058
Tofts, C. (1993). Algorithms for task allocation in ants. (A study of temporal polyethism: Theory). Bulletin of Mathematical Biology, 55(5), 891–918. https://doi.org/10.1007/bf02460691
Von Thienen, W., Metzler, D., Choe, D., & Witte, V. (2014). Pheromone communication in ants: a detailed analysis of concentration-dependent decisions in three species. Behavioral Ecology and Sociobiology, 68(10), 1611–1627. https://doi.org/10.1007/s00265-014-1770-3
Ware, J. L., & Wilson, M. (2022). Termites, Social Cockroaches. Elsevier EBooks. https://doi.org/10.1016/b978-0-12-822562-2.00015-3
Zhang, C., & Wu, B. (2019). Improvement of ant colony clustering algorithm based on pheromone updating strategy. Journal of Intelligent Systems, 28(1). [Original source: https://studycrumb.com/alphabetizer]